
肌肉mTOR通过NRF2,HIF和AKT/PKB信号通路控制铁稳态和铁
Agnès Conjard-Duplany1, Alexis Osseni2, Aline Lamboux3
1Laboratoire Physiopathologie et Génétique du Neurone et du Muscle (PGNM), Institut NeuroMyoGène, Université Claude Bernard Lyon 1, INSERM U1315, CNRS UMR 5261, 8 avenue Rockefeller, Lyon, 69008, France. agnes.duplany@univ-lyon1.fr.
Cellular and molecular life sciences : CMLS
|April 28, 2025

概括
哺乳动物目标的拉巴胺素 (mTOR) 缺乏会破坏肌肉的铁代谢,导致铁失调和肌肉病变. 精子胺补充剂可能有助于通过改善ferritinophagy恢复铁平衡和肌肉健康.
科学领域:
- 肌肉生理学 肌肉生理学
- 细胞铁代谢 细胞铁代谢
- 分子信号通道的分子信号通道.
背景情况:
- 拉巴胺素 (mTOR) 活性和铁平衡的平衡机械标对于肌肉完整性至关重要.
- mTOR与调节细胞铁水平有关,但其在肌肉铁代谢和肌肉病变中的特定作用尚未完全理解.
研究的目的:
- 为了研究mTOR缺乏,铁代谢和肌肉特异性mTOR淘汰 (mTORmKO) 小鼠中的肌肉病之间的关系.
- 阐明在mTOR缺陷肌肉中的铁失调背后的分子机制.
主要方法:
- 在mTORmKO小鼠的不同肌肉类型中分析铁含量,铁代谢蛋白 (TFR1,FTL,FPN) 和mRNA水平.
- 研究包括NRF2,HIF,AKT/PKB在内的信号通路及其对铁基因调节的影响.
- 评估精子胺补充剂对老年mTORmKO小鼠信号通路和铁代谢的影响.
主要成果:
- 尽管Ftl和FpnmRNA下调,mTORmKO小鼠显示出改变的铁模式和铁过剩标记 (TFR1降低,FTL和FPN蛋白增加) .
- mTOR 缺陷损害了NRF2和HIF介导的转录调节,并导致通过NRF2依赖机制和损害自的费里丁积累.
- 在老年mTORmKO小鼠中,精氨酸治疗使AKT/PKB-FOXO信号正常化,减少了总费里丁,并增加了索利乌斯肌肉中的内分泌体费里丁.
结论:
- mTOR在维持骨肌肉铁平衡中发挥着至关重要的作用.
- 不调节的铁代谢,特别是由于ferritinophagy受损而导致的费里丁积累,导致mTOR缺乏的肌肉病理.
- 精子胺显示出作为肌肉疾病的治疗剂的潜力,其特点是自阻塞和铁失调.
相关概念视频
 01:22
PI3K/mTOR/AKT Signaling Pathway
3.3K
The mammalian target of rapamycin (mTOR) is a serine/threonine kinase that regulates growth, proliferation, and cell survival in response to hormones, growth factors, or nutrient availability. This kinase exists in two structurally and functionally distinct forms: mTOR complex 1 (mTORC1) and mTOR complex 2 (mTORC2). The first form (mTORC1) is composed of a rapamycin-sensitive Raptor and proline-rich Akt substrate, PRAS40. In contrast, mTORC2 consists of a...
3.3K
 03:03
mTOR Signaling and Cancer Progression
3.6K
The mammalian target of rapamycin or mTOR protein was discovered in 1994 due to its direct interaction with rapamycin. The protein gets its name from a yeast homolog called TOR. The mTOR protein complex in mammalian cells plays a major role in balancing anabolic processes such as the synthesis of proteins, lipids, and nucleotides and catabolic processes, such as autophagy in response to environmental cues, such as availability of nutrients and growth factors.
The mTOR pathway or the...
The mTOR pathway or the...
3.6K
 02:23
Master Transcription Regulators
6.7K
Master transcription regulators are regulatory proteins that are predominantly responsible for regulating the expression of multiple genes. Often these genes work in concert to drive a complex process. Activation of a master transcription regulator can lead to a cascade of transcriptional activation necessary for that outcome. These regulators can directly bind to the regulatory sequences of the various genes involved, or they can indirectly regulate transcription by binding to regulatory...
6.7K
 01:31
Regulation of the Unfolded Protein Response
2.3K
Inositol-requiring kinase one or IRE1 is the most conserved eukaryotic unfolded protein response (UPR) receptor. It is a type I transmembrane protein kinase receptor with a distinctive site-specific RNase activity. As the binding mechanics of the misfolded proteins with the N-terminal domain of IRE-1 are unclear, three binding models — direct, indirect, and allosteric -- are proposed for receptor activation. Nevertheless, it is known that once a misfolded protein associates with IRE1, it...
2.3K
 01:19
Translocation of Proteins into the Mitochondria
3.0K
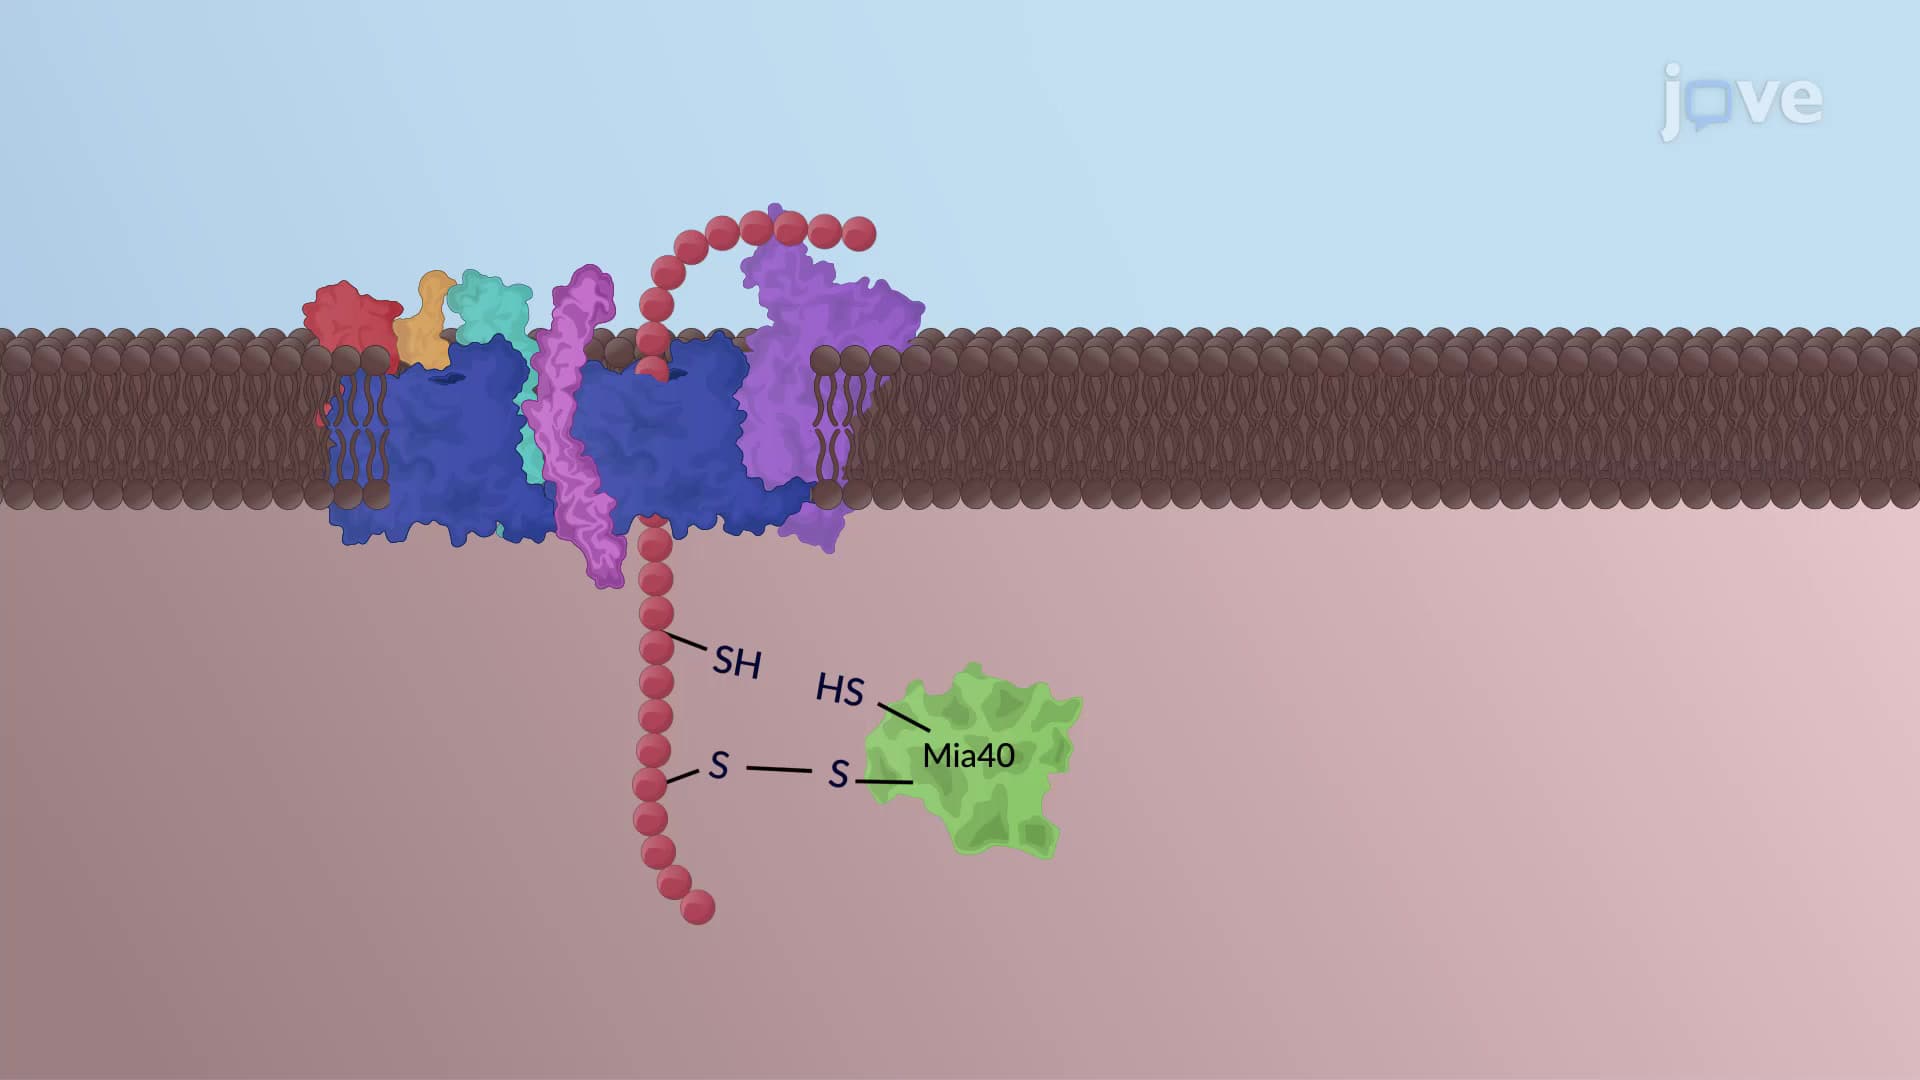
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
3.0K
 02:26
NF-κB-dependent Signaling Pathway
7.2K
The transcription factor NF-κB was discovered in 1986 in the lab of Nobel laureate Professor David Baltimore, for its interaction with the immunoglobulin light chain enhancer in B-cells. After more than three decades of study, it is now evident that NF-κB regulates the expression of over 100 genes. Most of these genes play an essential role in the innate and adaptive immune responses as well as the inflammatory responses of animals.
NF-κB-dependent Signaling Mechanism
The...
NF-κB-dependent Signaling Mechanism
The...
7.2K