
INI1的TARRNA仿真及其对HIV-1整合酶非整合功能的影响
Ganjam V Kalpana1, Emilie Ernst1, Swati Haldar1
1Department of Genetics, Albert Einstein College of Medicine, Bronx, NY 10461, USA.
Viruses
|May 28, 2025

概括
艾滋病毒-1整合酶 (IN) 与宿主因子INI1相互作用,模仿病毒RNA. 这种相互作用对HIV-1粒子的产生和组装至关重要,这表明了新的治疗点.
科学领域:
- 病毒学 病毒学
- 分子生物学分子生物学
- 结构生物学 结构生物学
背景情况:
- 艾滋病毒-1整合酶 (IN) 对于病毒整合至关重要,但也调节了诸如粒子产生等非整合功能.
- 在IN的非集成功能背后的精确机制仍然不完全理解.
- INI1是一种宿主因子,它与IN结合,并影响HIV-1的复制,粒子生成和形态发生.
研究的目的:
- 研究INI1在HIV-1粒子形态发生和组合中的作用.
- 探索INI1和病毒RNA (TARRNA) 在IN结合中的结构模仿.
- 提出INI1在HIV-1核糖核蛋白复合体形成中的功能模型.
主要方法:
- 对INI1结合有缺陷的IN突变的分析.
- 将INI1结合缺陷突变与RNA结合缺陷的IN突变进行比较.
- 结构分析INI1的重复1域及其与IN和TARRNA的相互作用.
主要成果:
- 缺陷INI1结合的IN突变体在粒子形态发生过程中表现出缺陷,类似于缺陷RNA结合的突变体.
- 在结构上,INI1的重复1域模仿TARRNA.
- INI1 和 TAR RNA 在与 HIV-1 整合酶的结合中竞争.
结论:
- INI1可能会作为病毒RNA的替代体,在HIV-1组装过程中促进适当的核糖蛋白复合体形成.
- 针对IN/INI1相互作用可以提供对IN/INI1和IN/RNA相互作用的双重抑制策略,从而抑制HIV-1复制.
更多相关视频
相关概念视频
 02:15
Experimental RNAi
6.3K
RNA interference (RNAi) is a cellular mechanism that inhibits gene expression by suppressing its transcription or activating the RNA degradation process. The mechanism was discovered by Andrew Fire and Craig Mello in 1998 in plants. Today, it is observed in almost all eukaryotes, including protozoa, flies, nematodes, insects, parasites, and mammals. This precise cellular mechanism of gene silencing has been developed into a technique that provides an efficient way to identify and determine the...
6.3K
 02:30
siRNA - Small Interfering RNAs
17.0K
Small interfering RNAs, or siRNAs, are short regulatory RNA molecules that can silence genes post-transcriptionally, as well as the transcriptional level in some cases. siRNAs are important for protecting cells against viral infections and silencing transposable genetic elements.
In the cytoplasm, siRNA is processed from a double-stranded RNA, which comes from either endogenous DNA transcription or exogenous sources like a virus. This double-stranded RNA is then cleaved by the...
In the cytoplasm, siRNA is processed from a double-stranded RNA, which comes from either endogenous DNA transcription or exogenous sources like a virus. This double-stranded RNA is then cleaved by the...
17.0K
 01:23
RNA Interference
26.5K
RNA interference (RNAi) is a process in which a small non-coding RNA molecule blocks the post-transcriptional expression of a gene by binding to its messenger RNA (mRNA) and preventing the protein from being translated.
This process occurs naturally in cells, often through the activity of genomically-encoded microRNAs. Researchers can take advantage of this mechanism by introducing synthetic RNAs to deactivate specific genes for research or therapeutic purposes. For example, RNAi could be used...
This process occurs naturally in cells, often through the activity of genomically-encoded microRNAs. Researchers can take advantage of this mechanism by introducing synthetic RNAs to deactivate specific genes for research or therapeutic purposes. For example, RNAi could be used...
26.5K
 02:57
piRNA - Piwi-interacting RNAs
7.0K
PIWI-interacting RNAs, or piRNAs, are the most abundant short non-coding RNAs. More than 20,000 genes have been found in humans that code for piRNAs while only 2000 genes have been found for miRNAs. piRNAs can act at the transcriptional and post-transcriptional levels and have a vital role in silencing transposable elements present in germ cells. They are also involved in epigenetic silencing and activation. Previously, they were thought to function only in germ cells but new evidence suggests...
7.0K
 01:29
Viruses with RNA Genomes
148
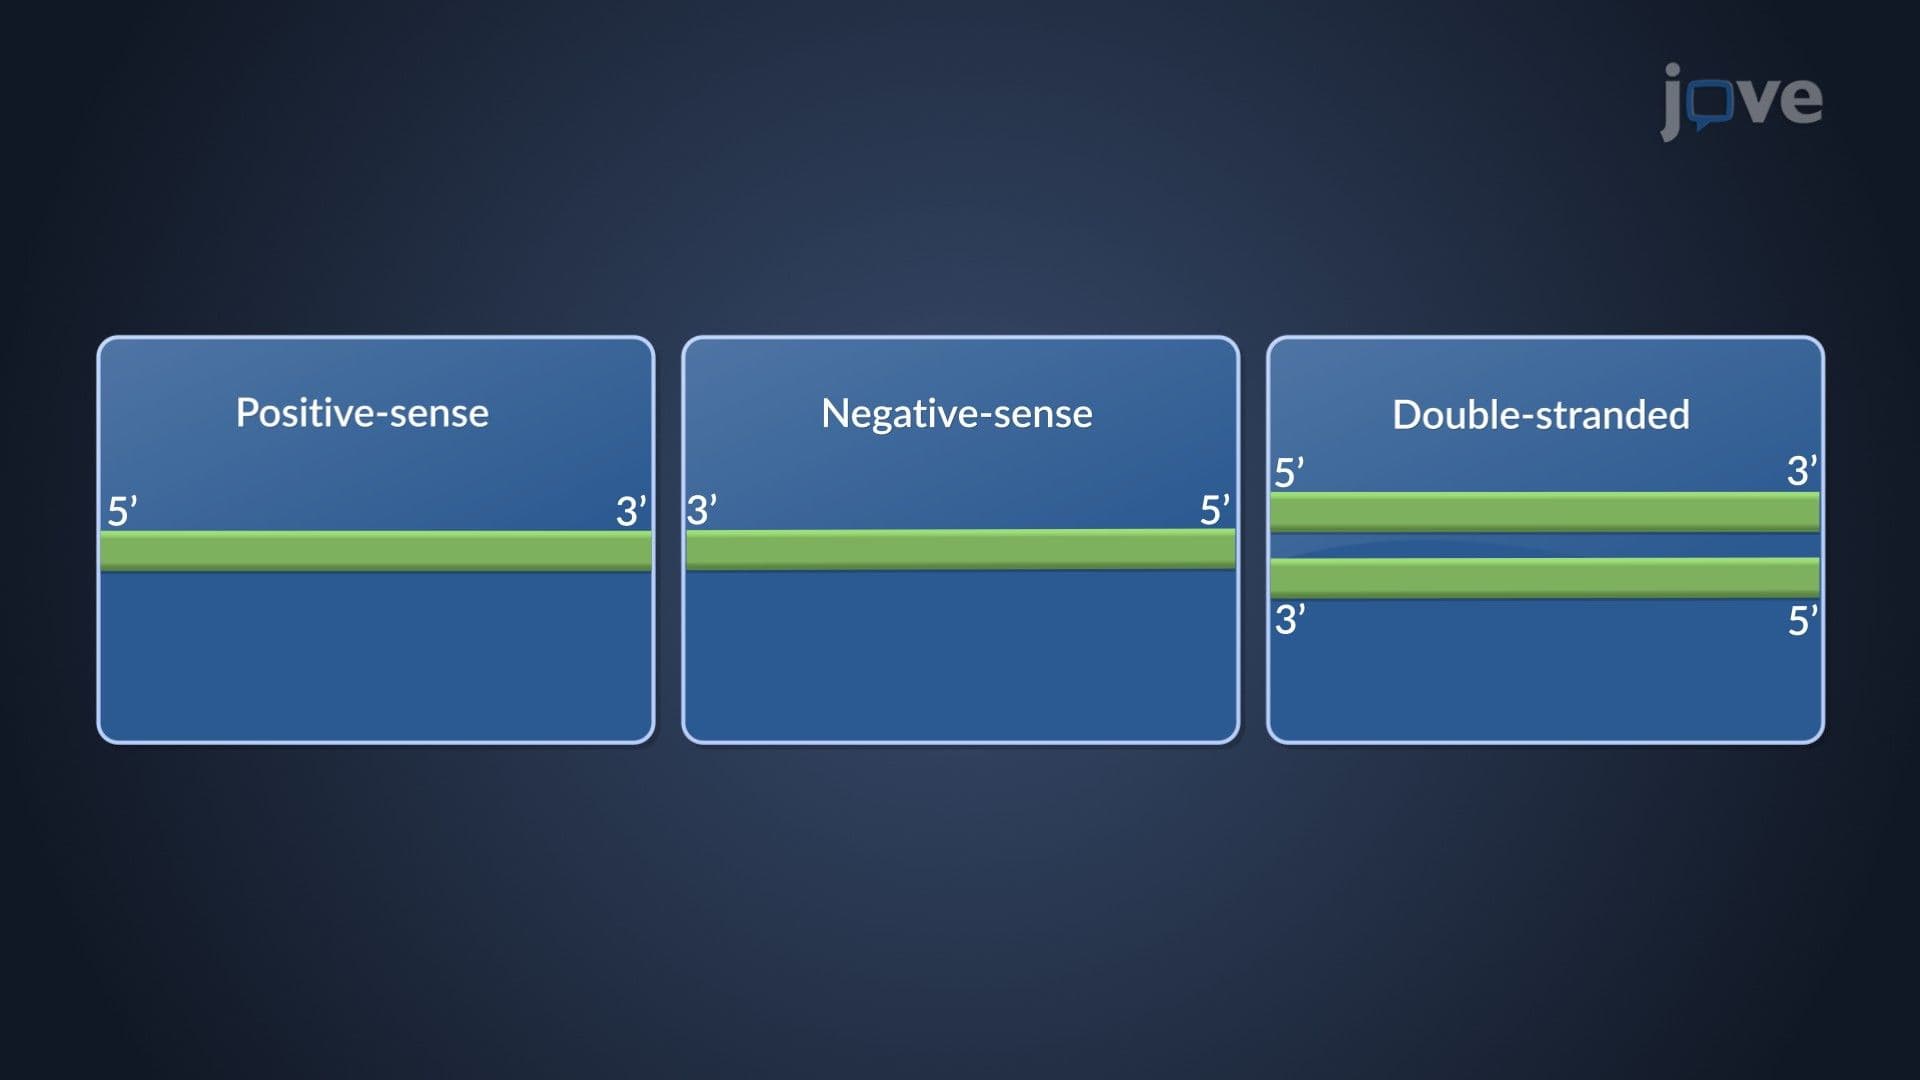
RNA viruses are categorized into positive-strand, negative-strand, or double-stranded groups based on their genomic structure and replication mechanisms. This classification dictates how they exploit host cellular machinery for protein synthesis and replication. Some RNA viruses also utilize reverse transcription as part of their life cycle, further diversifying their replication strategies.Positive-Strand RNA VirusesPositive-strand RNA viruses have genomes that function directly as messenger...
148
 03:08
LTR Retrotransposons
18.0K
LTR retrotransposons are class I transposable elements with long terminal repeats flanking an internal coding region. These elements are less abundant in mammals compared to other class I transposable elements. About 8 percent of human genomic DNA comprises LTR retrotransposons. Some of the common examples of LTR retrotransposons are Ty elements in yeast and Copia elements in Drosophila.
The internal coding region of LTR retrotransposons and their mechanism of transposition closely resembles a...
The internal coding region of LTR retrotransposons and their mechanism of transposition closely resembles a...
18.0K