相关实验视频
Updated: Sep 17, 2025
10:05

Ganglioside Extraction, Purification and Profiling
Published on: March 12, 2021
4.7K
在化物合成中,B4GALNT1的形态动力学和膜插入机制
Jack W J Welland1, Henry G Barrow1, Phillip J Stansfeld2
1Cambridge Institute for Medical Research, Department of Clinical Neuroscience, University of Cambridge, Cambridge, UK.
Nature communications
|July 2, 2025

概括
像B4GALNT1这样的葡萄糖脂酶对于大脑的化物合成至关重要. 了解它们的膜相互作用机制揭示了对神经疾病和癌症的洞察力.
科学领域:
- 生物化学 生化学
- 分子生物学分子生物学
- 结构生物学 结构生物学
背景情况:
- 葡萄糖脂 (GSL) 是细胞功能中涉及的必不可少的膜成分.
- 化物,复杂的GLS,由糖系转移酶合成;代谢失衡导致神经系统疾病.
- B4GALNT1对于合成主要的大脑化物前体至关重要,其功能障碍与遗传性性和癌症有关.
研究的目的:
- 阐明B4GALNT1在脂质基质加工中的功能结构和机制基础.
- 为了研究B4GALNT1与脂质双层相互作用中的活性位点侧环的作用.
- 提出一种由GSL合成酶的基质访问和处理的保存机制.
主要方法:
- 进行X射线晶体学以确定人类同位体B4GALNT1.1.的结构.
- 位点定向突变发生,以评估循环残留物变化对酶活性的影响.
- 分子动力学模拟用于模拟酶-膜相互作用.
主要成果:
- 在催化过程中,晶体结构揭示了B4GALNT1基质结合部位的动态重塑.
- 活动部位旁边的表面环中的疏水性到极性残留物的突变损害了脂质基质加工.
- 分子动力学模拟表明,这些循环可以插入脂质双层,促进基质访问.
结论:
- B4GALNT1通过涉及表面环的动态膜插入机制访问和处理脂质基质.
- 这种动态膜插入的机制很可能在其他结构上不同的GSL合成酶中得到保留.
- 了解这种机制,可以了解与GSL代谢相关的神经疾病和癌症.
相关概念视频
 01:33
Coat Assembly and GTPases
3.6K
Vesicles incorporate different coat protein subunits in different cell locations, which changes the properties of the coat, such as the shape and geometry of the transport vesicles. Thus, vesicle coat proteins also play a significant role in cargo selection.
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
3.6K
 01:32
Pinching-off of Coated Vesicles
3.3K
Vesicle budding is orchestrated by distinct cytosolic proteins such as adaptor proteins, coat proteins, and GTPases. To initiate vesicle budding, membrane-bending proteins containing crescent-shaped BAR domains bind to the lipid heads in the bilayer and distort the membrane to form a protein-coated vesicle bud. Adaptors proteins such as AP2 for clathrin-coated vesicles can nucleate on the deformed membrane. Finally, coat proteins such as clathrin or COPI and COPII assemble into a coat forming...
3.3K
 01:24
Oligosaccharide Assembly
3.0K
Protein glycosylation starts in the ER lumen and continues in the Golgi apparatus. Glycosyltransferases catalyze the addition of sugar molecules or glycosylation of proteins. Usually, these enzymes add sugars to the hydroxyl groups of selected serine or threonine residues to form O-linked glycans or the amino groups of asparagine residues to form N-linked glycans. Different positions on the same polypeptide chain can contain differently linked glycans.
Multiple sugar molecules that may or may...
Multiple sugar molecules that may or may...
3.0K
 01:28
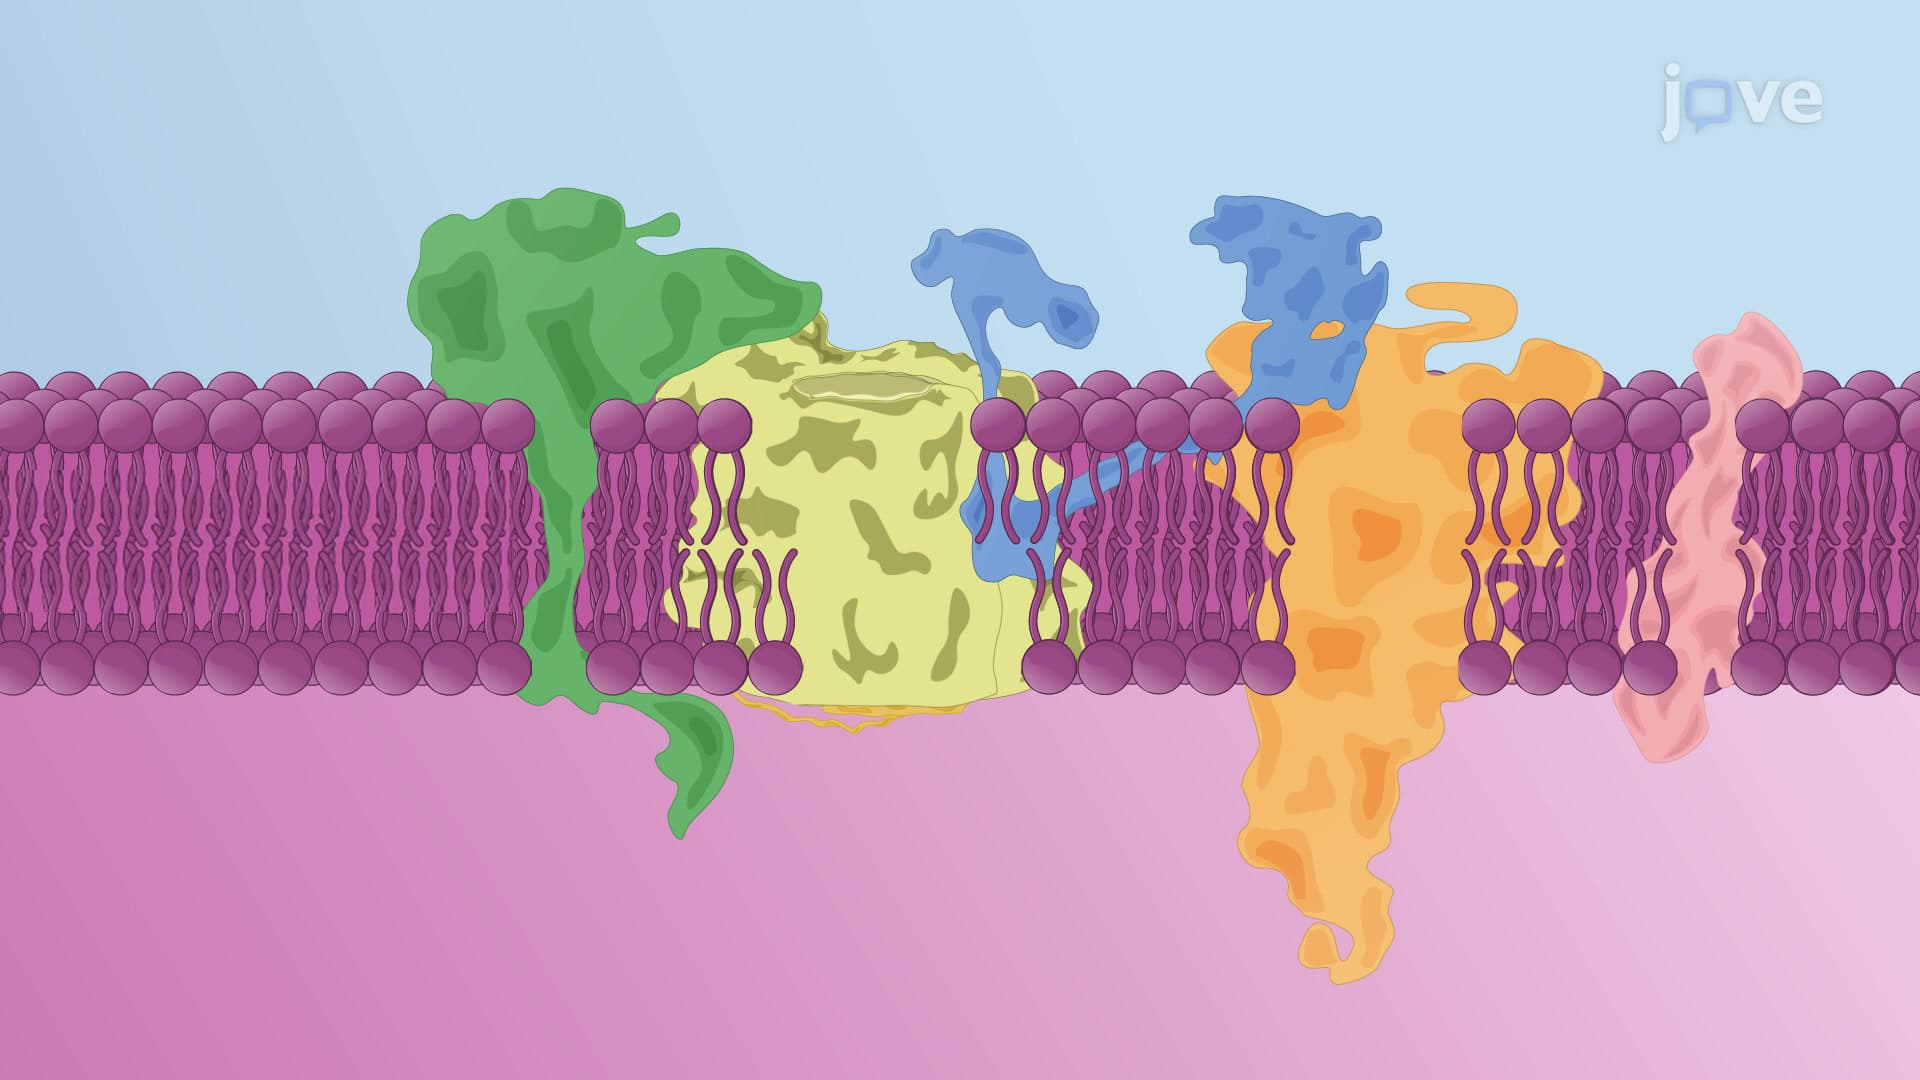
Protein Translocation Machinery on the ER Membrane
5.0K
The translocon complex situated on the ER membrane is the main gateway for the protein secretory pathway. It facilitates the transport of nascent peptides into the ER lumen and their insertion into the ER membrane.
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the...
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the...
5.0K
 01:45
Tail-anchoring of Proteins in the ER Membrane
3.2K
Tail-anchored, or TA, proteins are estimated to make up to 3-5% of membrane proteins found in the eukaryotic cell. Such proteins have a single transmembrane domain located approximately 30 amino acid residues upstream from the C-terminal end. As a result, the signal recognition particle (SRP) cannot guide a TA protein to the ER membrane for cotranslational insertion. Hence, they are integrated into the ER membrane post-translationally using their C-terminal end as the anchor. TA proteins...
3.2K
 01:29
GPI Anchoring of Proteins in the ER Membrane
4.3K
GPI-anchoring is a post-translational, reversible protein modification that is ubiquitous in eukaryotes. Such proteins are primarily present on the exoplasmic leaflet of the plasma membrane.
GPI-anchor structure
A sequence of 11 enzymatic reactions results in the synthesis of the complete GPI anchor consisting of a hydrophobic and a hydrophilic portion. The hydrophobic portion comprises phosphatidylinositol, while the hydrophilic part comprises polar groups like phosphoethanolamine,...
GPI-anchor structure
A sequence of 11 enzymatic reactions results in the synthesis of the complete GPI anchor consisting of a hydrophobic and a hydrophilic portion. The hydrophobic portion comprises phosphatidylinositol, while the hydrophilic part comprises polar groups like phosphoethanolamine,...
4.3K