
来自Mycobacterium tuberculosis的硫脂-1激活了Gαq/11结合的通路,以增加感觉神经元的刺激性
Dhananjay K Naik1, Felipe Espinosa1, Ifunanya M Okolie1
1Department of Neuroscience and Center for Advanced Pain Studies, University of Texas at Dallas, Richardson, TX, USA.
Journal of neurophysiology
|December 15, 2025

概括
结核性脂质,特别是硫-1,通过G蛋白合受体直接激活感官神经元,增加神经元刺激能力,并可能导致咳. 这项研究揭示了一种新的机制,将病原体脂质与结核病中的咳反射联系起来.
科学领域:
- 神经科学是一个神经科学.
- 免疫学 免疫学 免疫学
- 微生物学 微生物学
背景情况:
- 咳是结核病 (TB) 的主要症状,也是疾病传播的关键因素.
- 之前的研究表明,Mycobacterium tuberculosis脂质提取物 (Mtb提取物) 和其成分硫脂-1 (SL-1) 通过作用于感知神经元可以诱导咳.
- 这种相互作用背后的精确细胞机制尚未完全理解.
研究的目的:
- 阐明Mtb提取物和SL-1调节感知神经元的细胞机制.
- 研究G蛋白结合受体 (GPCRs) 和细胞内信号在Mtb提取物诱导的神经元反应中的作用.
- 为了确定Mtb提取物是否会影响感官神经元的刺激性.
主要方法:
- 成像被用来测量来自小鼠结节和人类背根 (hDRG) 的TRPV1+神经元中的细胞内Ca2+信号.
- 评估了YM254890,Gαq/11抑制剂对Ca2+信号传递的影响.
- 在治疗Mtb提取物后,在小鼠节点性感受体中测量了动作潜能 (AP) 生成和兴奋性.
主要成果:
- Mtb提取物和SL-1在老鼠和人类感官神经元中显著增加了细胞内Ca2+信号.
- 这些Ca2+增加被YM254890减弱,这表明GPCR介导的机制涉及Gαq/11向细胞内Ca2+储存器发送信号.
- Mtb提取物增强了小鼠结节神经元中的AP生成和增加了AP半宽,这表明了电压受控离子通道的调制.
- Mtb 提取物对神经元刺激性和AP 半幅度的影响被 YM254890.0 阻止.
结论:
- 结核病原体衍生的脂质,包括SL-1,通过GPCRs直接激活感官神经元.
- 这种激活涉及Gαq/11信号传递,导致细胞内的增加和神经元刺激性的增强.
- 这些发现提供了结核病脂质与感觉神经元活动调节之间的直接联系,为结核病相关咳的机制提供了洞察力.
相关概念视频
 01:11
IP3/DAG Signaling Pathway
14.2K
Membrane lipids such as phosphatidylinositol (PI) are precursors for several membrane-bound and soluble second messengers. Specific kinases phosphorylate PI and produce phosphorylated inositol phospholipids. One such inositol phospholipids are the phosphatidylinositol-4,5 bisphosphate [PI(4,5)P2], present in the inner half of the lipid bilayer. Upon ligand binding, GPCR stimulates Gq proteins to turn on phospholipase Cꞵ. Activated phospholipase Cꞵ cleaves PI(4,5)P2 and...
14.2K
 01:30
Ligand-Gated Ion Channel Receptor: Gating Mechanism
3.7K
Ligand-gated ion channels are transmembrane proteins that play a vital role in intercellular communication and functions of the nervous system. They allow the influx of ions across the membrane once the neurotransmitter binds, allowing the subsequent transmission of electrical excitation across the neurons. Other ligand-gated ion channels, like the γ-aminobutyric acid (GABA) receptor, permit anions like chloride into the cells on the binding of the GABA molecule. Their entry into the cell...
3.7K
 01:22
Activation and Inactivation of G Proteins
10.7K
Heterotrimeric G proteins are guanine nucleotide-binding proteins. As the name suggests, heterotrimeric G proteins are composed of three subunits: alpha, beta, and gamma. They remain GDP-bound or GTP-bound inside the cells and switch between inactive/active states. The Gα subunit possesses the nucleotide-binding pocket that binds guanine nucleotides and switches between GDP or GTP-bound states. In contrast, the Gꞵ and Gγ subunits are always bound together with high...
10.7K
 01:21
G-Protein Gated Ion Channels
5.5K
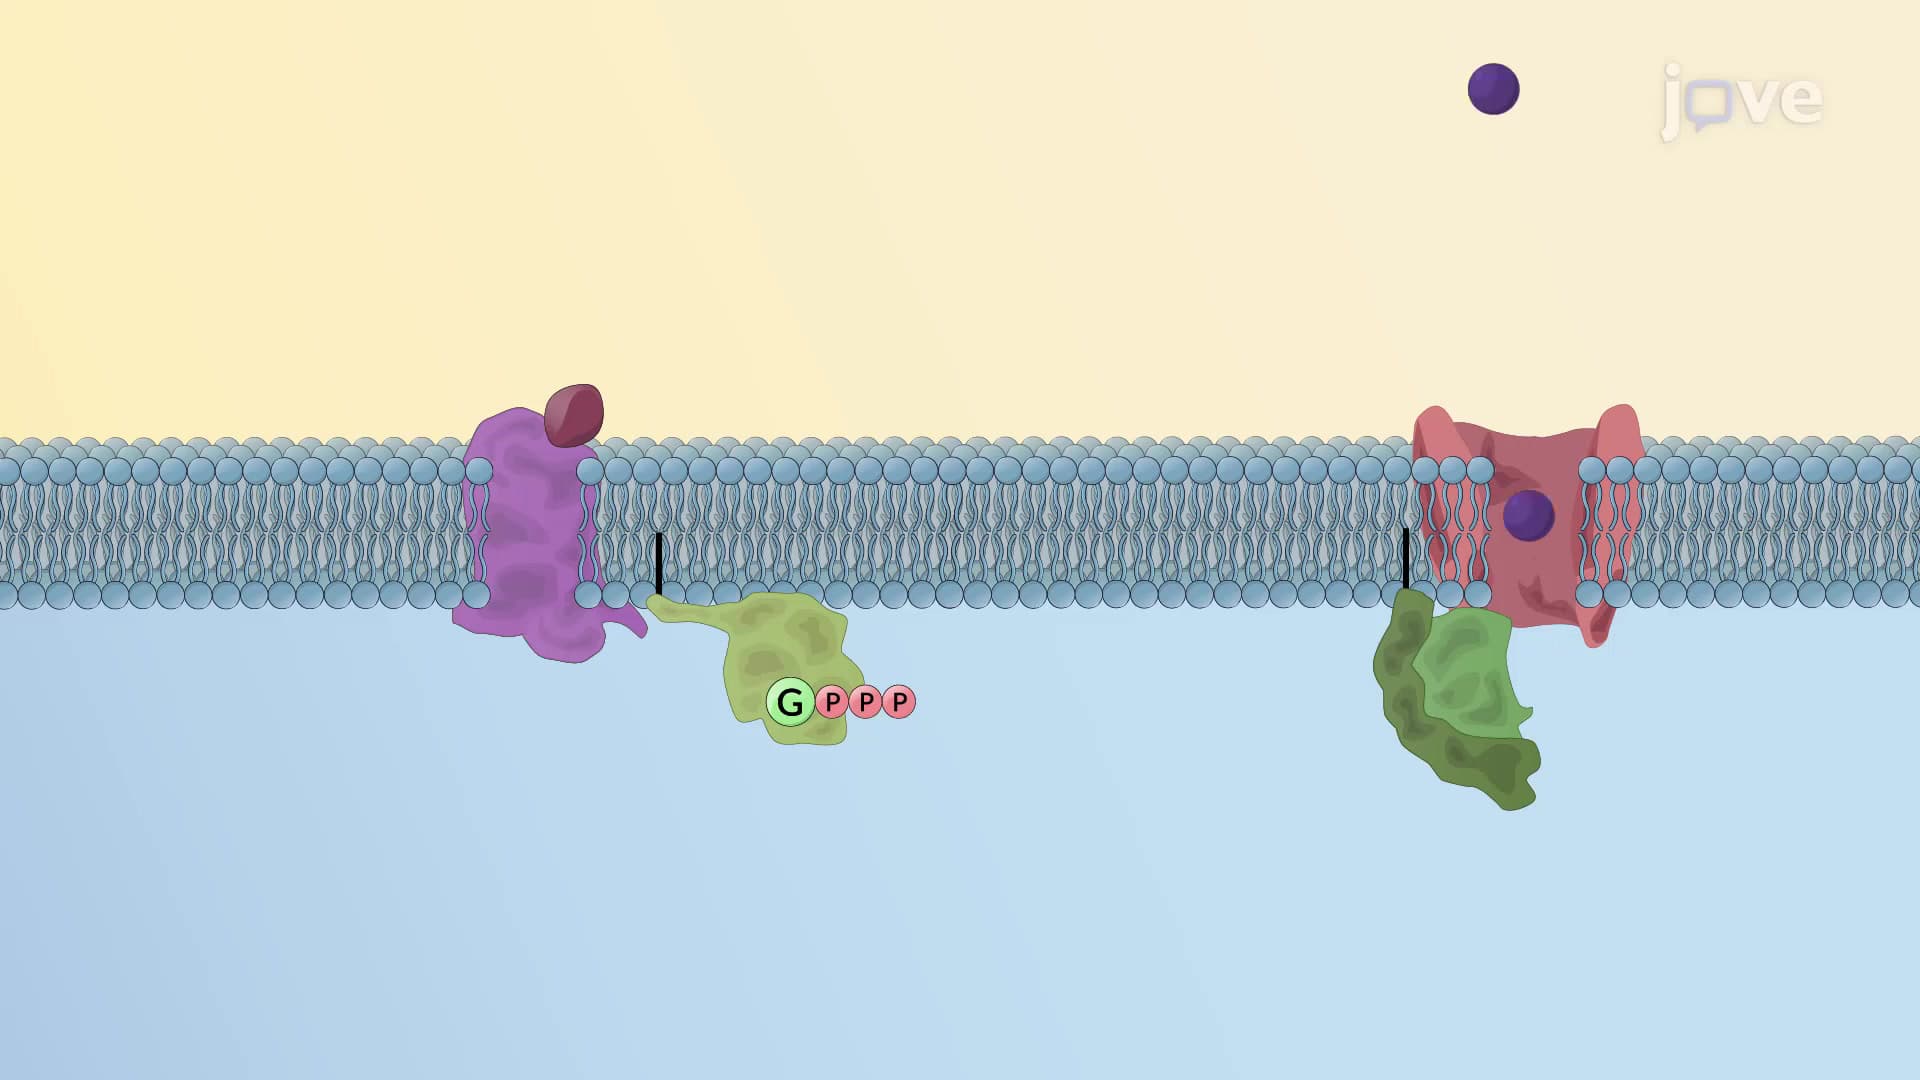
GPCRs are primarily responsible for our sense of smell, taste, and vision. The binding of a sensory stimulus activates GPCR to stimulate effector proteins, many of which are ion channels in the sensory organs. GPCRs modulate the opening and closing of the target ion channels either directly by binding them, or by releasing second messengers that activate these channels. As ions move across the membrane, the membrane potential is altered, which induces an appropriate response.
Sensory...
Sensory...
5.5K
 01:28
Gene Regulation in Microbial Communities: Quorum Sensing
463
Quorum sensing is a mechanism of bacterial communication that enables coordinated gene expression in response to changes in population density. This facilitates collective behaviors that enhance survival, resource acquisition, and ecological adaptation. This process relies on small signaling molecules called autoinducers that accumulate as bacterial populations grow. When a critical threshold concentration of autoinducers is reached, bacterial cells collectively modify gene expression,...
463
 01:09
GPCRs Regulate Adenylyl Cylase Activity
7.2K
Some GPCRs transmit signals through adenylyl cyclase (AC), a transmembrane enzyme. AC helps synthesize second messenger cyclic adenosine monophosphate (cAMP). AC catalyzes cyclization reaction and converts ATP to cAMP by releasing a pyrophosphate. The pyrophosphate is further hydrolyzed to phosphate by the enzyme pyrophosphatase, which drives cAMP synthesis to completion. However, cAMP is rapidly degraded to 5′ AMP by the enzymes phosphodiesterase (PDE), preventing overstimulation of...
7.2K