
通过细胞透Pep-1的曲率诱导的膜重塑
Yasith Indigahawela Gamage1, Jianjun Pan1
1Department of Physics, University of South Florida, Tampa, FL 33620, USA.
Membranes
|December 24, 2025

概括
细胞透Pep-1根据其组成不同地重塑脂质膜. 它会导致一些膜的解体,以及在其他膜的重组或曲率产生,影响转位.
科学领域:
- 生物物理学的生物物理.
- 膜生物学 膜生物学
- 生物化学 生物化学
背景情况:
- 像Pep-1这样的细胞透 (CPP) 对于药物输送至关重要.
- 了解CPP如何与脂质膜相互作用和重塑是优化其功能的关键.
- 佩普-1的膜扰动的精确结构机制在很大程度上仍未被描述.
研究的目的:
- 为了研究Pep-1的膜重塑活动的结构细节.
- 检查Pep-1扰动如何支持具有不同组成和几何形状的脂质双层.
- 阐明 - 膜相互作用的组成依赖的途径.
主要方法:
- 使用原子力显微镜 (AFM) 可视化Pep-1对脂质双层的影响.
- 研究了由不同脂质 (POPC,POPS) 和胆固醇组成的支持性脂质双层.
- 分析的重点是膜形态变化,包括边缘效应,破坏和重组.
主要成果:
- 在POPC双层中,Pep-1引起了边缘侵蚀和分解.
- 阴性POPS脂质增强了Pep-1结合,导致局部破坏和聚合物形成.
- 含胆固醇的双层显示了表面重组,具有状特征,表明脂质再分配和曲率生成.
- 在连续的POPC/POPS双层中,Pep-1形成了类似花朵的突出,这些突出网络成厚厚的域.
结论:
- -1的膜重塑高度依赖于脂质组成和双层几何.
- 该可以根据其机械和静电性质来破坏稳定,重组或曲线膜.
- 这些发现为细胞透转位机制提供了关键的见解.
相关概念视频
 01:15
Mechanisms of Membrane-bending
3.2K
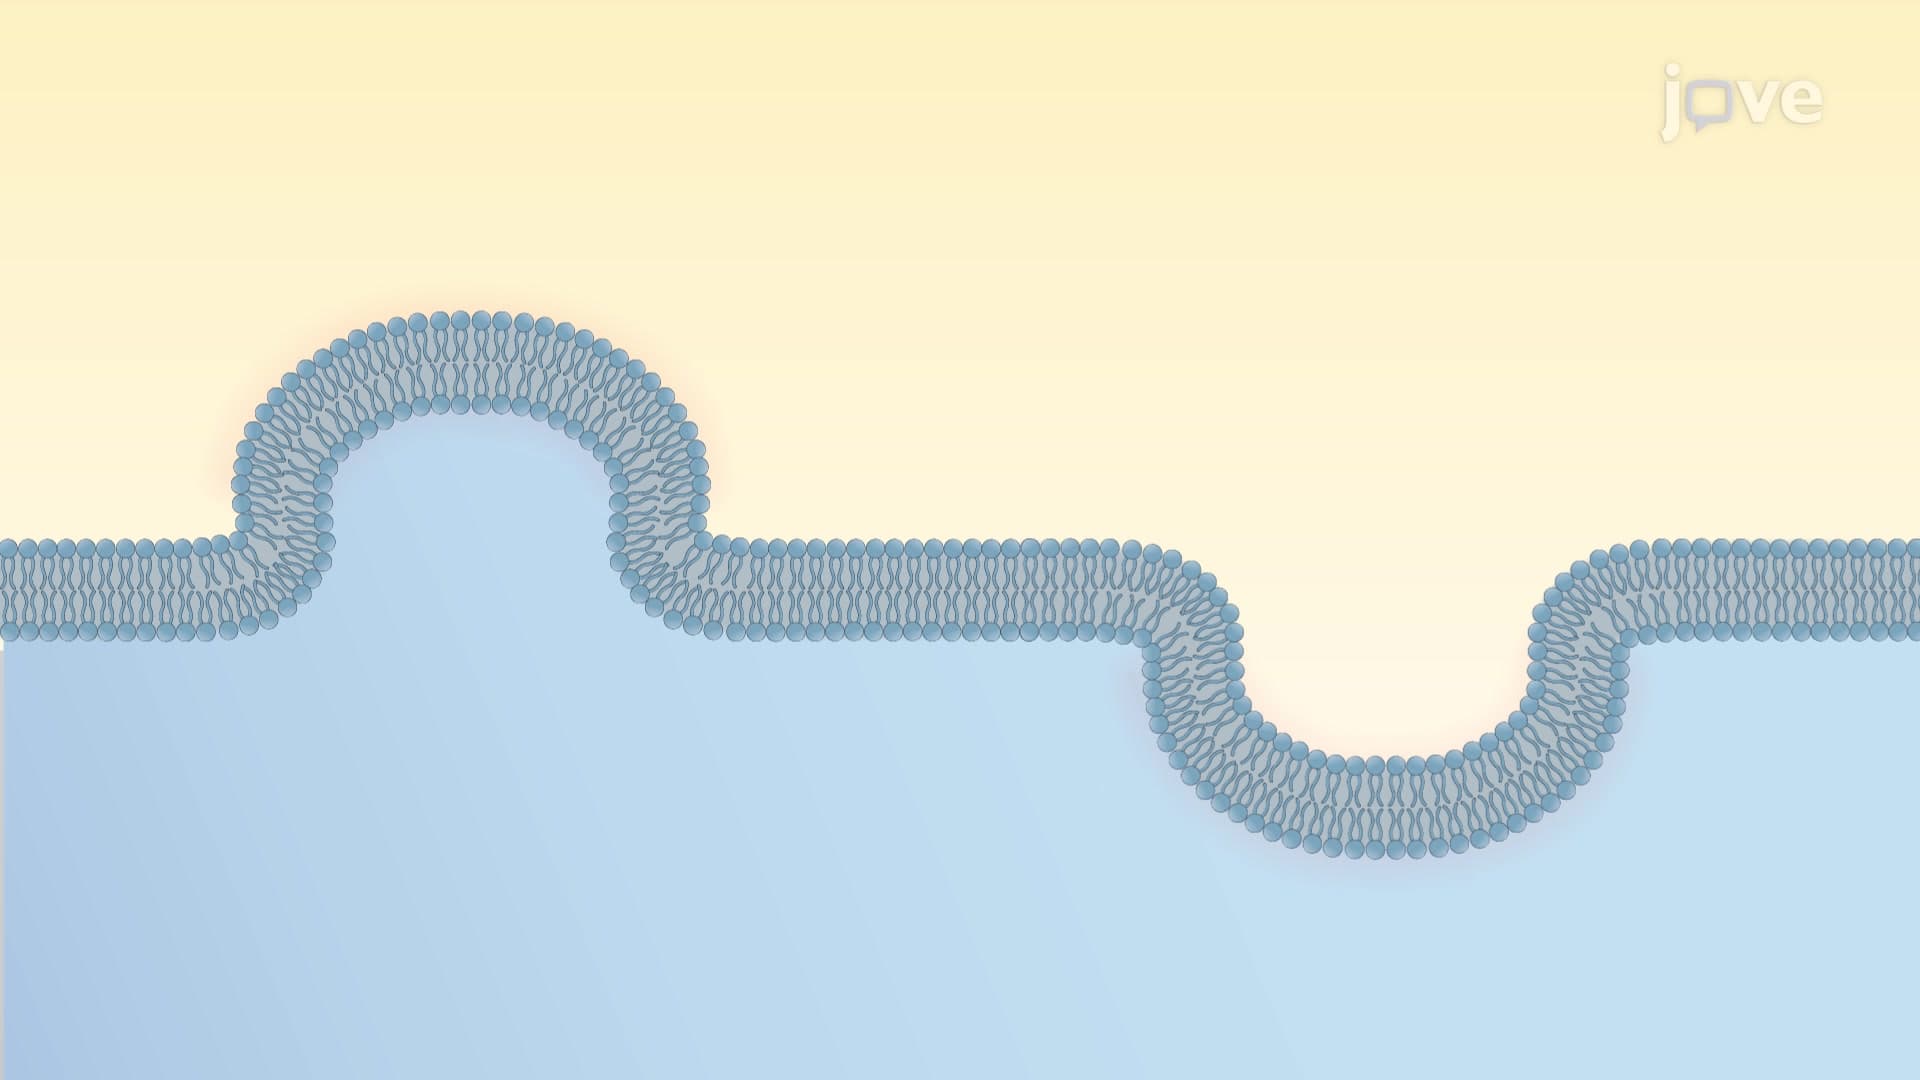
The living membranes are flexible due to their fluid mosaic nature; however, their bending into different shapes is an active process regulated by specific lipids and proteins. The membrane bending can be transient as seen in vesicles or stable for a long time as in microvilli. Cells regulate the size, location, and duration of the membrane curvature.
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
3.2K
 01:16
Cell Motility through Blebbing
2.4K
Blebs are a type of membrane protrusion formed by the internal hydrostatic pressure of the cytoplasm. Blebs are observed in several cell types, including fibroblasts, immune cells, and single-celled organisms like the amoeba. The primary function of blebs is cell locomotion and apoptosis, but they are also found during necrosis and cell division. The life cycle of a bleb comprises an initiation phase followed by the expansion and retraction phases.
Blebbing Through the Matrix
In multicellular...
Blebbing Through the Matrix
In multicellular...
2.4K
 01:28
Types of Membrane Protrusions
3.5K
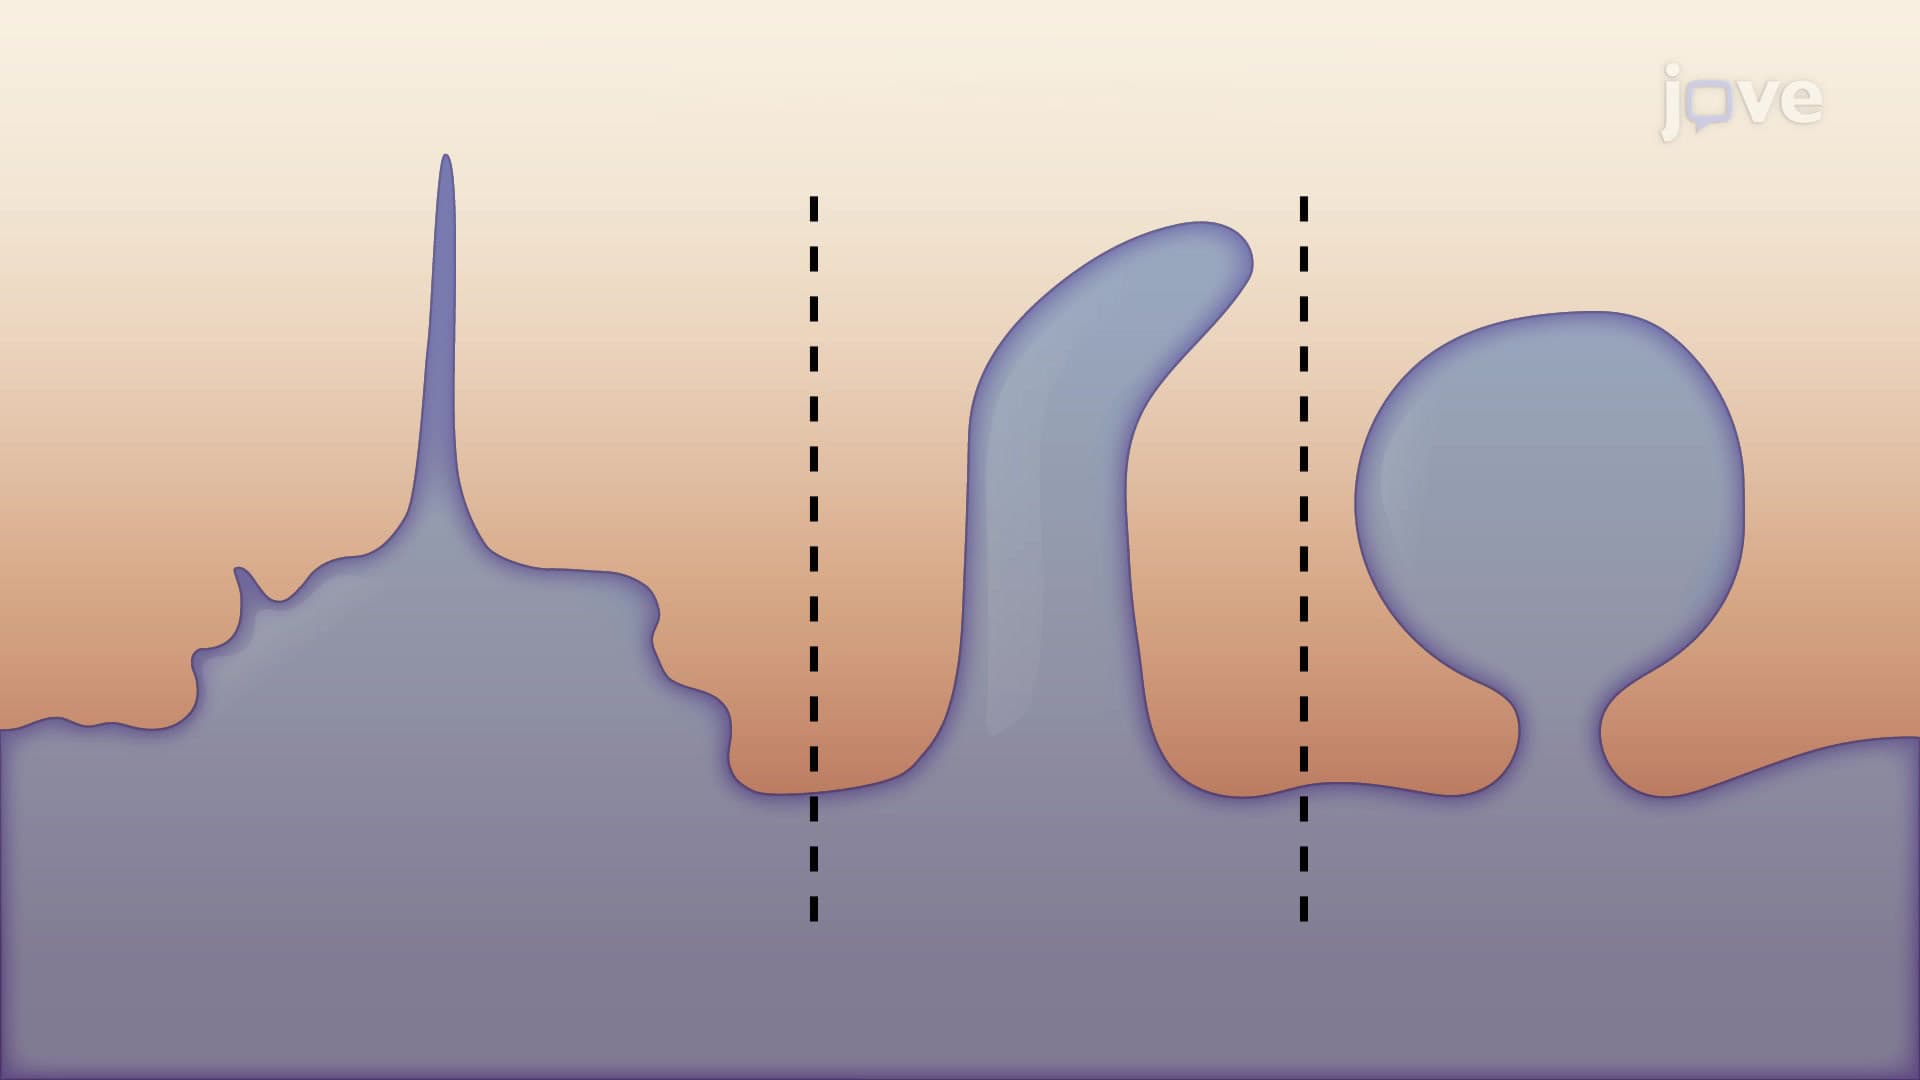
The protrusion of the cell surface is an initial step for several cellular processes, including cell migration, phagocytosis, and neurite outgrowth. These membrane protrusions are a result of cytoskeletal rearrangement. The most widely observed cell protrusions include lamellipodia, pseudopodia, filopodia, microvilli, invadopodia, and podosomes. These protrusions can be of two types — static or dynamic.
The microvilli, an example of stable protrusions, are finger-like projections...
The microvilli, an example of stable protrusions, are finger-like projections...
3.5K
 01:22
Enlargement of the Plasma Membrane
2.2K
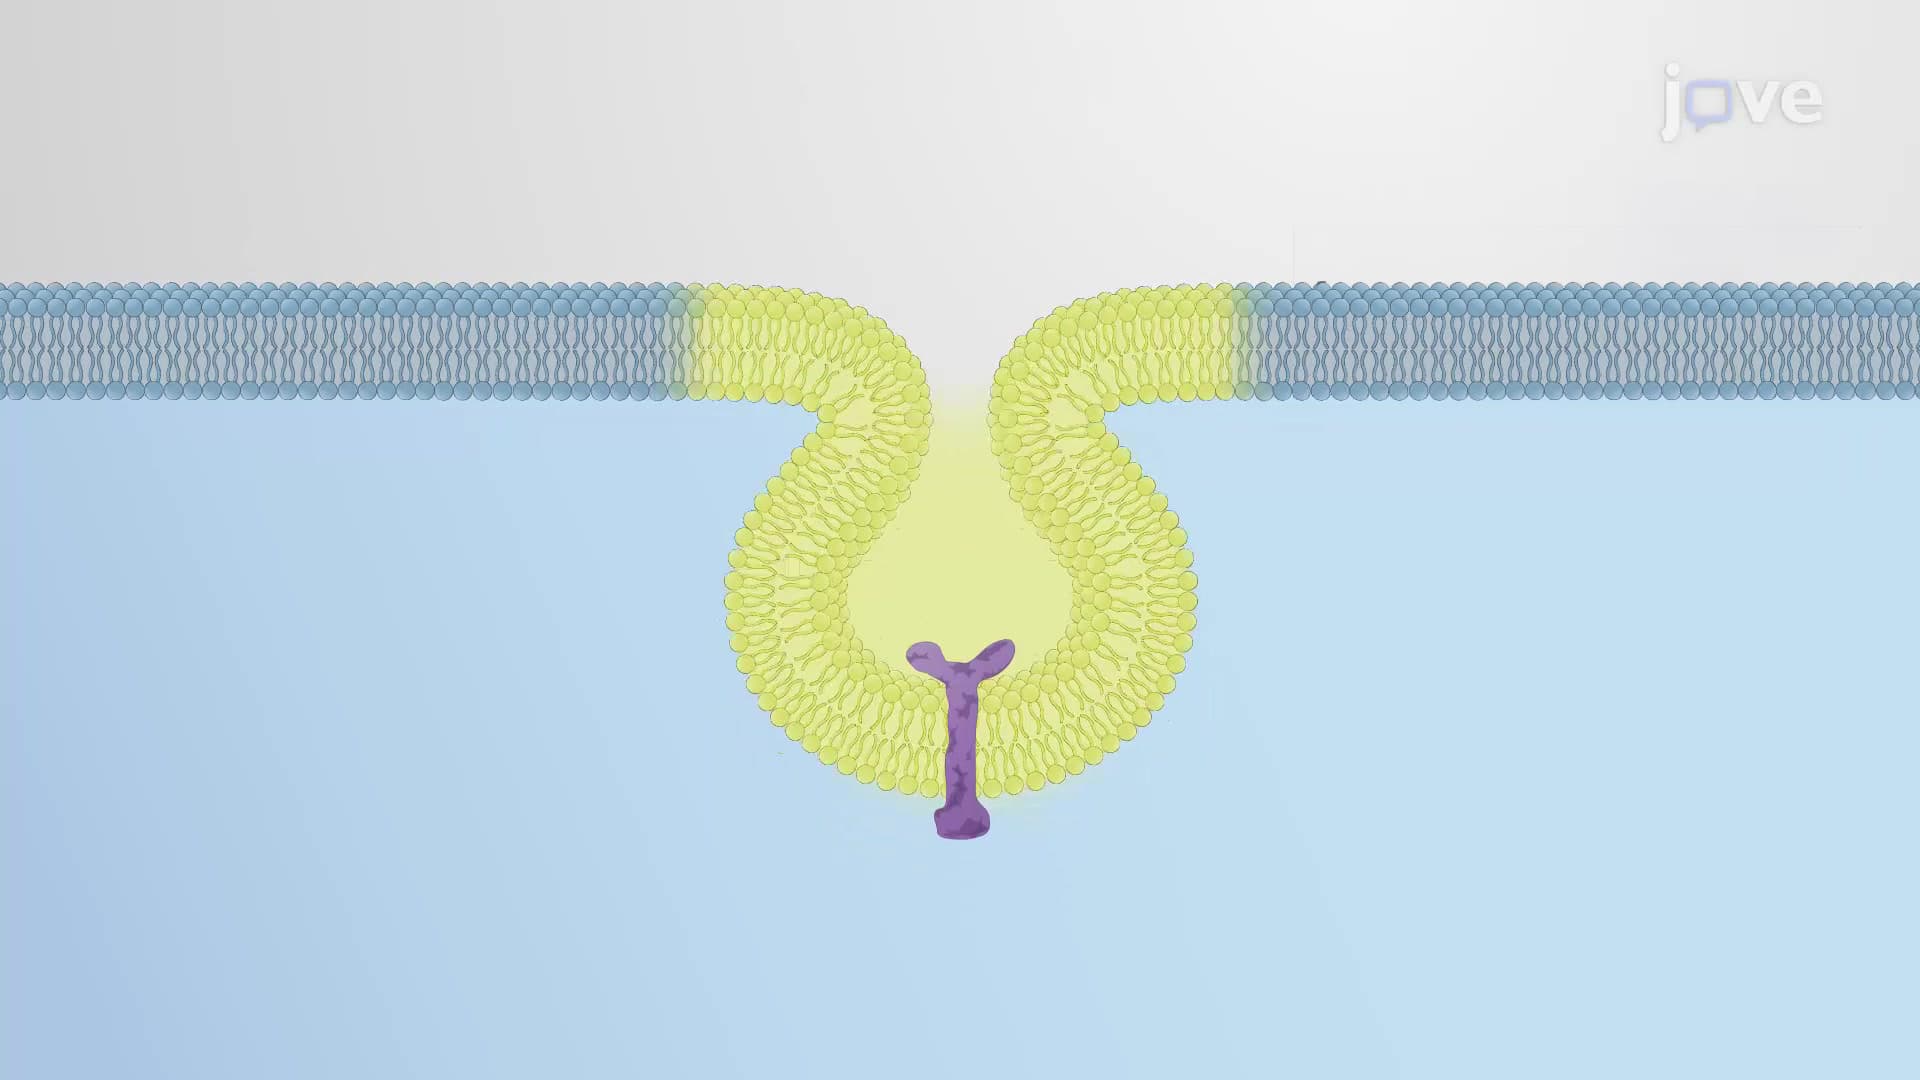
Cell division and enlargement are processes that require precise control. The control ensures that cell division cannot proceed unless the cell has grown to a specific size. A spherical, dividing cell requires an approximately 1.6X increase in its surface area to double its volume. The secretory pathway also has a significant role in cell membrane enlargement. Secretory vesicles that bud off from the Golgi apparatus and later fuse with the plasma membrane during exocytosis are a major source of...
2.2K
 01:31
Mechanism of Lamellipodia Formation
3.5K
Cells migrating in response to external stimuli form lamellipodia, which are thin membrane protrusions supported by a mesh of linked, branched, or unbranched actin filaments. These actin filaments interact with myosin motor proteins, creating the dynamic actomyosin complex within the cytoskeleton. Contractility, or the ability to generate contractile stress, is inherent to the actomyosin complex. It helps cells detect the stiffness of the surrounding ECM and exert contractile force for...
3.5K
 01:45
Tail-anchoring of Proteins in the ER Membrane
3.6K
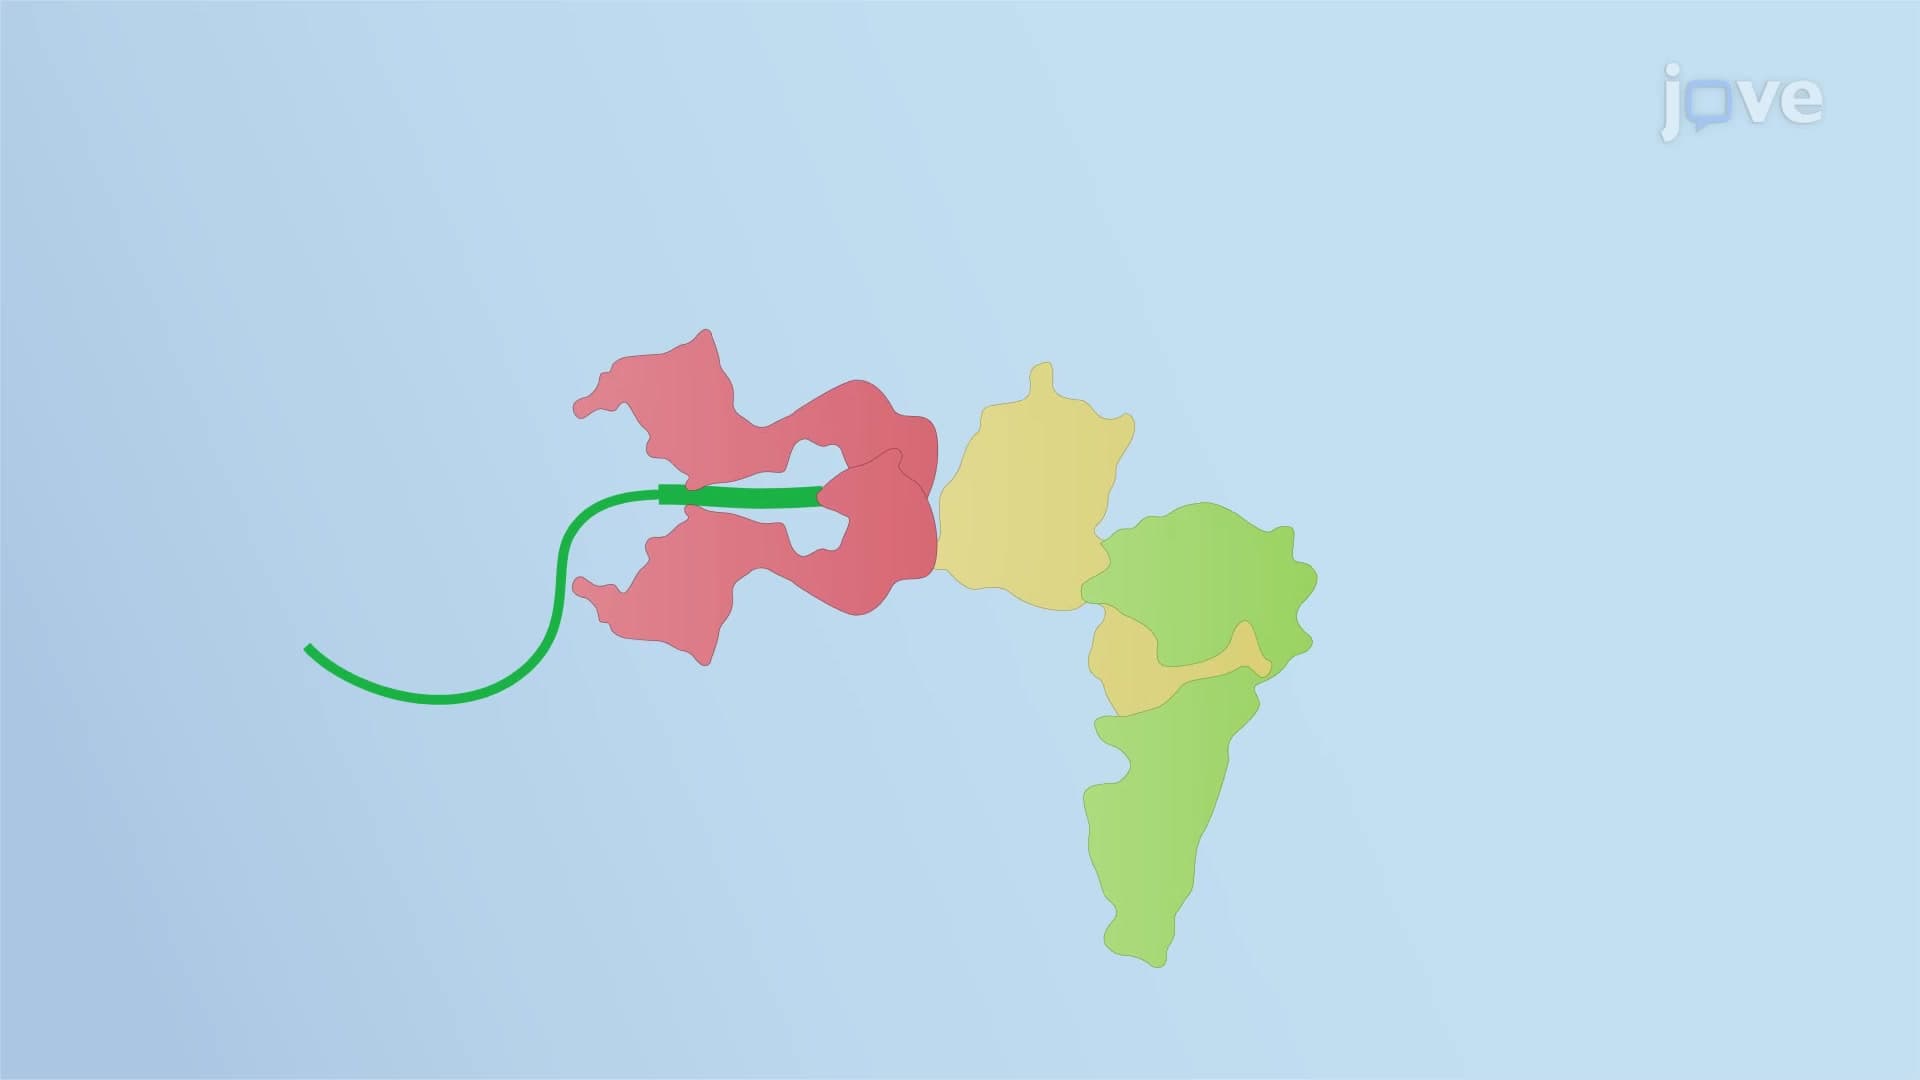
Tail-anchored, or TA, proteins are estimated to make up to 3-5% of membrane proteins found in the eukaryotic cell. Such proteins have a single transmembrane domain located approximately 30 amino acid residues upstream from the C-terminal end. As a result, the signal recognition particle (SRP) cannot guide a TA protein to the ER membrane for cotranslational insertion. Hence, they are integrated into the ER membrane post-translationally using their C-terminal end as the anchor. TA proteins...
3.6K