
膀性乙胆载体的突变增加了管乙化,影响了突触膀的运输
Cheng-Shan Kuo1, Vignesh Mahendran Ruckmani1, Meng-Chieh Wang1
1Department of Life Science, Institute of Molecular and Cellular Biology, National Tsing Hua University, Hsinchu, Taiwan, ROC.
Journal of neurochemistry
|December 26, 2025

概括
在Kinesin-3UNC-104的遗传缺陷导致神经系统疾病. 提升的氨酸乙化损害了UNC-104的运动功能和突触囊泡运输,揭示了一个新的调节机制.
科学领域:
- 神经科学和分子生物学
- 细胞运输机制的细胞运输机制.
- 神经系统疾病的遗传学
背景情况:
- 素-3 UNC-104 (KIF1A) 对于突触囊泡的前级轴突运输至关重要.
- UNC-104中的缺陷与KIF1A相关的神经疾病 (KAND) 有关,包括CMT和HSP.
- 素的翻译后修饰,如乙化,可以影响轴突运输.
研究的目的:
- 为了研究神经传递缺陷,氨酸乙化和UNC-104功能之间的关系.
- 为了确定影响素乙化的基因及其对C. elegans.中轴突运输的影响.
- 阐明UNC-104运输规则背后的分子机制.
主要方法:
- 在C. elegans中进行候选基因查,寻找影响神经传递和蛋白修饰的基因.
- 在ALM神经元中跟踪UNC-104和RAB-3运动,使用免疫染.
- 对MEC-17 (α-tubulin乙转移酶) 和UNC-17 (膀性乙胆载体) 的基因操纵 (敲除/过度表达).
- 使用双分子光补充 (BiFC) 和共免疫沉 (Co-IP) 验证蛋白质与蛋白质相互作用.
主要成果:
- 在体内,unc-17(e245) 的等位基因显著增加了素乙化.
- 在unc-17(e245) 菌株中提升的氨酸乙化会损害UNC-104的机动和货物 (RAB-3) 运动.
- 在MEC-17突变体中,MEC-17 Knockdown提高了UNC-104的运动性,而在野生动物中,MEC-17的过度表达会损害其.
- UNC-104,UNC-17和MEC-17形成一个三元复合体;UNC-17的变化影响MEC-17的局部化和氨酸乙烯化.
- 由于中断了UNC-17功能而增加的氨酸乙化抑制了UNC-104的过程性和运输效率.
结论:
- 囊泡性乙胆载体UNC-17在调节氨酸乙化中起作用.
- 素乙化增加,可能由MEC-17介导,损害了依赖于Kinesin-3 UNC-104的轴突运输.
- 这项研究揭示了一种涉及UNC-104,UNC-17和MEC-17的神经元功能的新型调节途径,影响神经元功能和潜在的KAND病原体.
相关概念视频
 01:45
Vesicular Tubular Clusters
3.0K
After budding out from the ER membrane, some COPII vesicles lose their coat and fuse with one another to form larger vesicles and interconnected tubules called vesicular tubular clusters or VTCs. These clusters constitute a compartment at the ER-Golgi interface known as ERGIC (Endoplasmic Reticulum Golgi Intermediate Compartment). The ERGIC is a mobile membrane-bound cargo transport system that sorts proteins secreted from ER and delivers them to the Golgi.
With the help of motor proteins such...
With the help of motor proteins such...
3.0K
 01:33
Overview of Secretory Vesicles
9.3K
Secretory vesicles, also known as dense core vesicles (DCVs), are membrane-bound vesicles that transport secretory proteins, such as hormones or neurotransmitters. Regulated secretory vesicles transport proteins from the trans-Golgi network to the exterior of the cell. Proteins present in regulated secretory vesicles are required to be rapidly exocytosed in large amounts upon a specific stimulus.
Various proteins regulate the aggregation of molecules inside the secretory vesicles. Chromogranins...
Various proteins regulate the aggregation of molecules inside the secretory vesicles. Chromogranins...
9.3K
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
16.5K
Proteins and neurotransmitters in secretory vesicles can be released from a cell upon vesicle docking, priming, and fusion with the plasma membrane. Vesicles are docked and primed in preparation for the quick exocytosis of their contents in response to a stimulus. The fusion process is mainly carried out by a SNAP Receptor or SNARE complex, consisting of synaptobrevin, syntaxin-1, and SNAP-25.
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
16.5K
 01:23
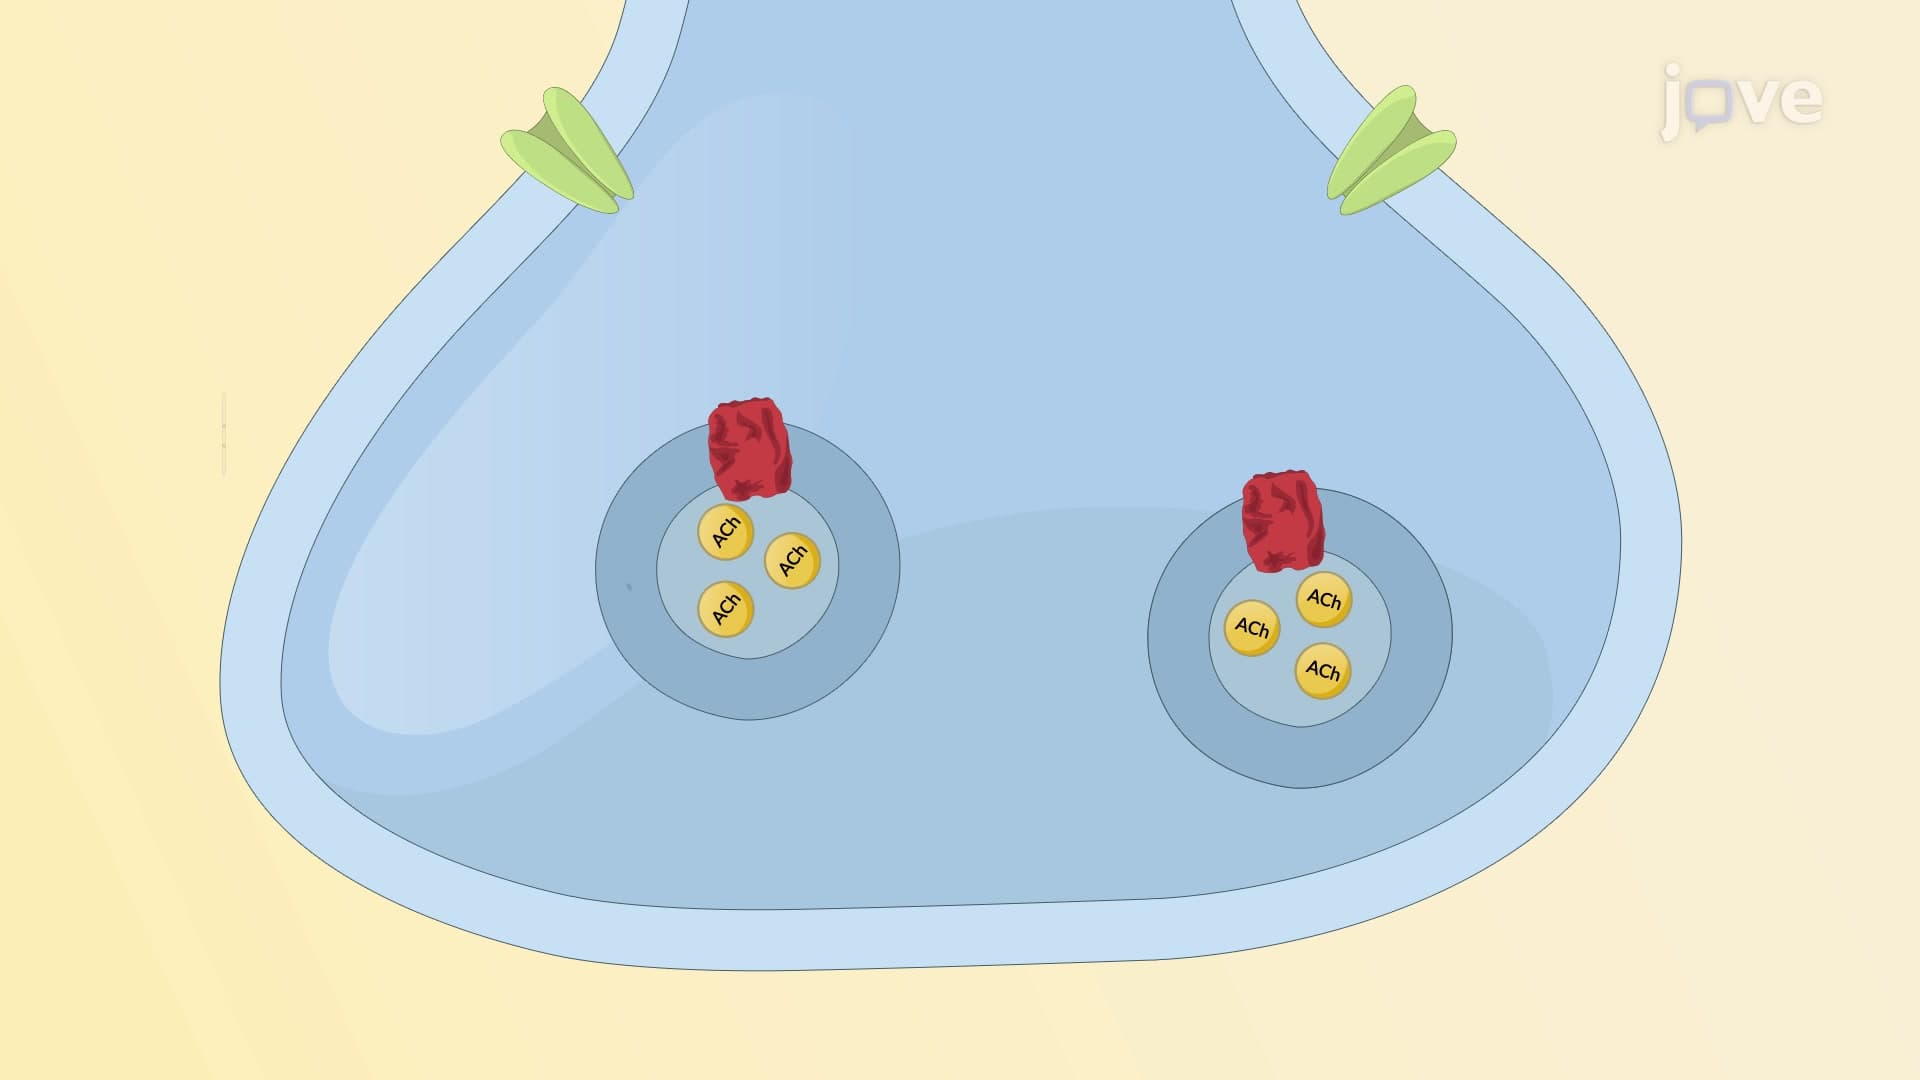
Cholinergic Neurons: Neurotransmission
4.9K
Cholinergic neurotransmission involves the synthesis and the release of acetylcholine (ACh) in order to transmit nerve impulses across the synapse. The process begins with the synthesis of acetyl CoA, a precursor for ACh, from ATP, acetate, and coenzyme A in the mitochondria. Choline, another vital precursor, is transported inside the neuron through choline transporters, including high-affinity choline transporter CHT1, low-affinity choline transporter CTL1, and lower-affinity choline...
4.9K
 01:38
Intralumenal Vesicles and Multivesicular Bodies
4.6K
Intraluminal vesicles (ILVs) are small vesicles 50-80 nm in diameter formed during the maturation of early endosomes. A specialized endosome containing numerous ILVs is called a multivesicular body (MVB). ILVs contain internalized molecules such as antigens, nucleic acids, proteins, and metabolites. Some of these molecules are released from the MVBs inside exosomes and are transported to other cells. Other MVBs contain molecules that are retained in the ILVs and are later degraded within the...
4.6K
 01:45
Destabilization of Microtubules
3.4K
The destabilization of microtubules can occur during different stages of the microtubule lifecycle, such as nucleation or elongation. It can take place at either end of the microtubule or in the microtubule lattices as a whole. The lifespan of individual microtubules within a cell varies according to the cell type and stage of the cell cycle. During interphase, the lifespan of the microtubule is about 30 minutes, while during cell division, it is about 15 minutes. In axonal microtubules of...
3.4K