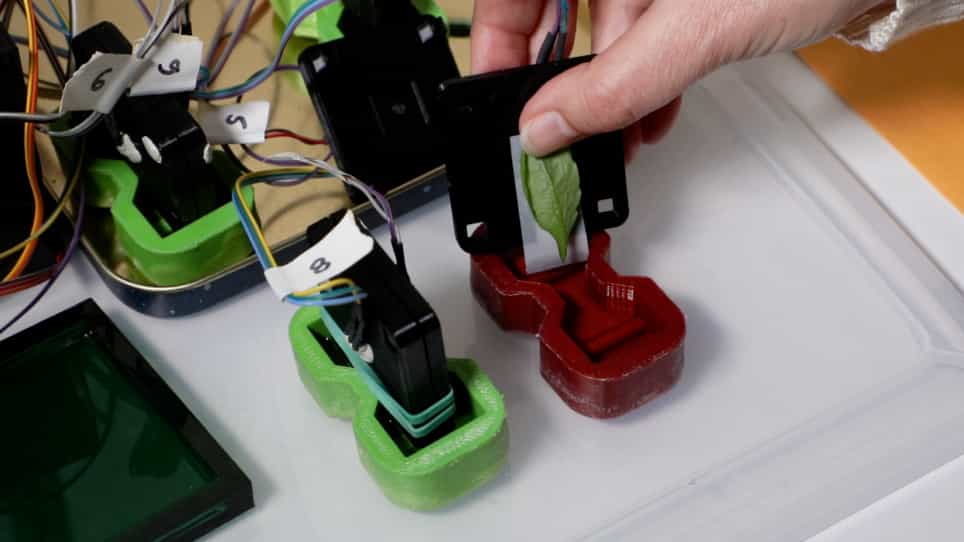
光热素监测的是实际温度,而不是温度差异,通过Marchantia多态生物中的 cis-trans自化模式切换来调节温度依赖的叶绿体运动
Minoru Noguchi1, Tatsushi Fukushima1,2, Saki Wakasugi1,2
1Center for Bioscience Research and Education, Utsunomiya University, Tochigi, 321-8505, Japan.
Planta
|January 17, 2026

概括
肝中的光热素 (图) 作为直接温度传感器,而不是感知温度差异. 它切换自化模式来控制叶绿体的运动,使植物能够避免寒冷损伤.
科学领域:
- 植物生物学 植物生物学
- 摄影生物学 摄影生物学
- 蜂信号传输是如何进行的
背景情况:
- 植物中蓝光 (BL) 诱导的叶绿体运动表现出温度依赖的反应.
- 在高温下,叶绿体在BL (积累反应) 中积累;在低温下,它们移动 (避冷反应),以防止光损伤.
- 光热素 (图) 是一个BL受体和热传感器,通过温度和BL依赖的自酸化来调节这个开关.
研究的目的:
- 为了研究光热素是否感知实际温度或温度差异,以调节叶绿体的运动.
- 阐明光热素的自酸化模式在温度传感中的作用.
主要方法:
- 在受控的温度变化下,分析肝草Marchantia polymorpha中光热素介导的叶绿体运动.
- 监测光热素的 cis-和 trans-自化状态,以应对温度变化.
主要成果:
- 发现叶绿体的运动是对实际环境温度的反应,而不仅仅是温度波动.
- 光热素被确认为实际温度的植物内传感器.
- 光热素的自酸化活性随着温度的降低而增加.
- 叶绿体积累和避免反应之间的转变与光热素自酸化从cis-到trans-的转变相关.
结论:
- 光热素作为植物实际温度的直接传感器.
- 温度传感机制涉及光热素的自酸化模式 (cis-到 trans-) 的切换.
- 这种机制调节了叶绿体的运动,允许植物适应不同温度,避免细胞损伤.
相关概念视频
 02:00
Photoreceptors and Plant Responses to Light
28.3K
Light plays a significant role in regulating the growth and development of plants. In addition to providing energy for photosynthesis, light provides other important cues to regulate a range of developmental and physiological responses in plants.
28.3K
 01:24
Protein Transport to the Stroma
2.2K
Chloroplasts are triple membrane structures with an outer membrane, an inner membrane, and a thylakoid membrane, each containing distinct metabolite transporters, membrane translocons, and enzymes. Appropriate sorting and translocating these proteins to their correct membrane systems is essential for chloroplast function.
Protein complexes called the translocon of the outer chloroplast membrane or TOC complex, and the translocon of the inner chloroplast membrane or TIC complex mediate the...
Protein complexes called the translocon of the outer chloroplast membrane or TOC complex, and the translocon of the inner chloroplast membrane or TIC complex mediate the...
2.2K
 01:18
Protein Transport to the Inner Chloroplast Membrane
2.4K
Proteins targeted to the inner chloroplast membrane, or plastid proteins, are transported by two general pathways: the stop-transfer and the re-insertion or post-import pathways. Most plastid proteins carry N-terminal transit sequences and internal import sequences targeting it to the specific chloroplast subcompartment. Proteins targeted by the stop-transfer pathway have internal hydrophobic sequences that inhibit their translocation into the stroma. As a result, these precursors are arrested...
2.4K
 02:45
Biological Clocks and Seasonal Responses
41.5K
The circadian—or biological—clock is an intrinsic, timekeeping, molecular mechanism that allows plants to coordinate physiological activities over 24-hour cycles called circadian rhythms. Photoperiodism is a collective term for the biological responses of plants to variations in the relative lengths of dark and light periods. The period of light-exposure is called the photoperiod.
41.5K
 01:11
Channel Rhodopsins
3.1K
Most organisms use photoreceptors to sense and respond to light. Examples of photoreceptors include bacteriorhodopsins and bacteriophytochromes in some bacteria, phytochromes in plants, and rhodopsins in the photoreceptor cells of the vertebral retina. The light-sensitive property of these receptors is because of the bound chromophores, such as bilin in the phytochromes and retinal in the rhodopsins.
Rhodopsins belong to the family of cell surface proteins called G-protein coupled receptors,...
Rhodopsins belong to the family of cell surface proteins called G-protein coupled receptors,...
3.1K
 01:11
Protein Transport to the Outer Chloroplast Membrane
2.3K
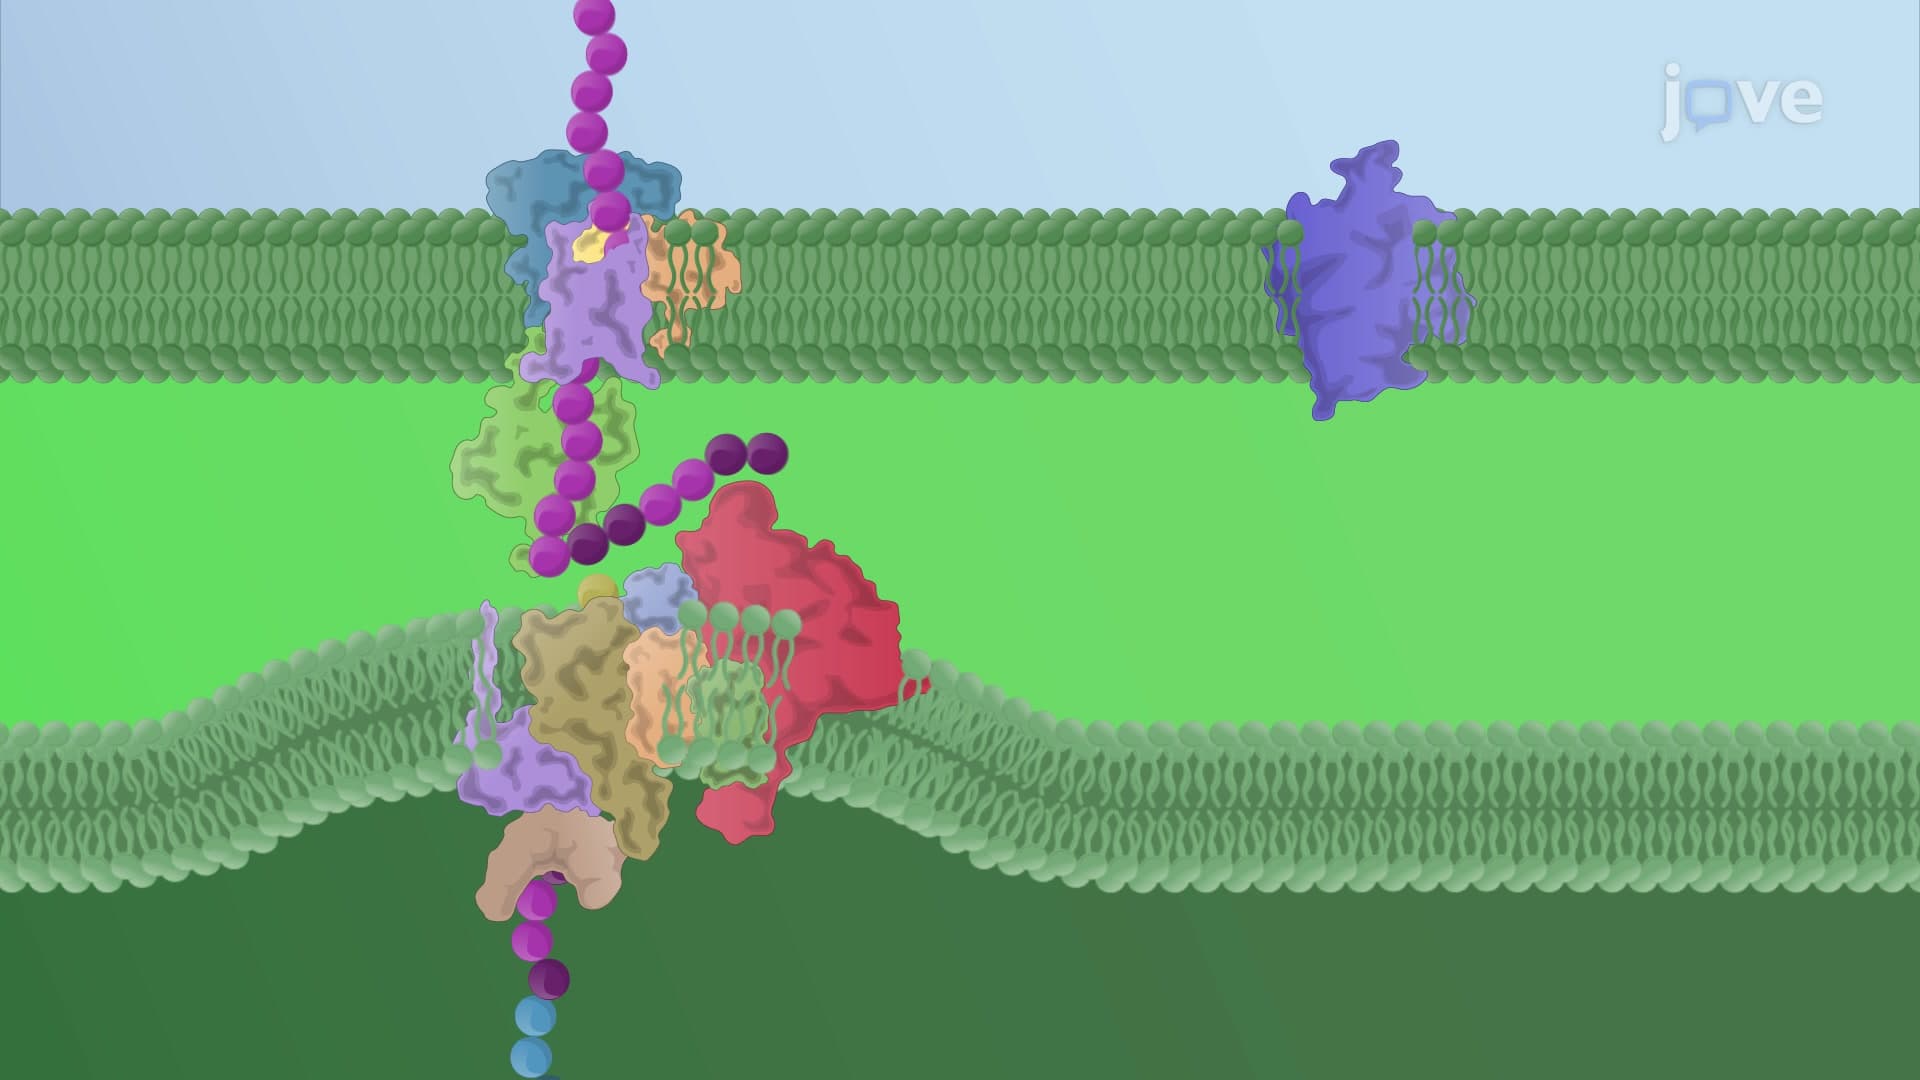
Chloroplast outer membrane proteins encoded by the nucleus are synthesized in the cytosol. Soon after synthesis, they bind cytosolic factors such as 14-3-3 protein and the Hsp70 chaperones that keep these precursors in an unfolded state until their translocation.
Two models describe the mechanism of precursor recognition and entry across the outer membrane through the TOC complex. Model 1 suggests the newly synthesized precursor binds to the TOC receptor 159 and forms a complex.
Two models describe the mechanism of precursor recognition and entry across the outer membrane through the TOC complex. Model 1 suggests the newly synthesized precursor binds to the TOC receptor 159 and forms a complex.
2.3K