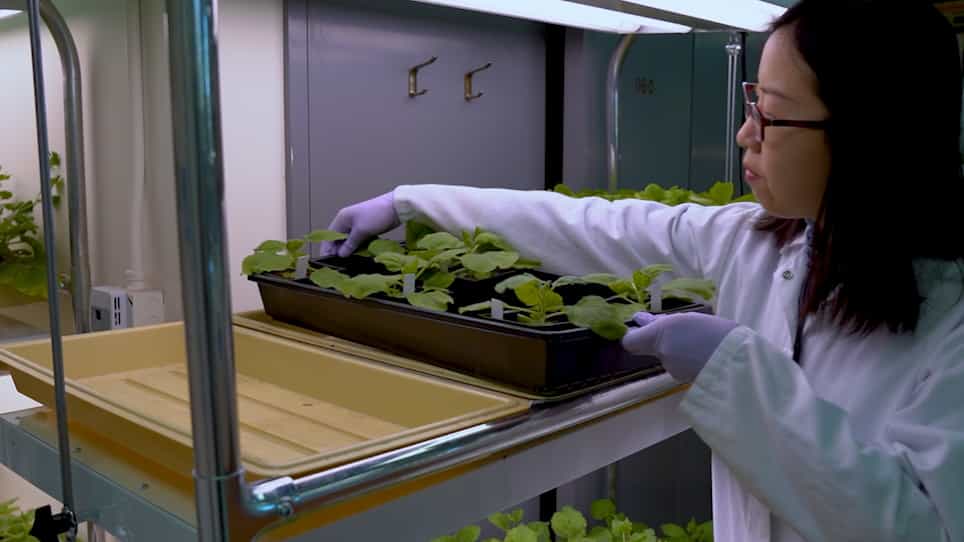

在高光下,使用基于TurboID的近距离标记来识别Arabidopsis thaliana的叶片质体中的PsbS结合蛋白
Yuwei Jiao1,2, Yanhui Dou1,2, Lihua Wang1
1Center for Excellence in Molecular Plant Sciences, Chinese Academy of Sciences, Shanghai, China.
Frontiers in plant science
|February 5, 2026

概括
光系统II子单元S (PsbS) 调节植物的光保护. 这项研究使用近距离标记来识别PsbS相互作用蛋白质,揭示新的合作伙伴,并建议PsbS通过构造变化而不是迁移来发挥作用.
科学领域:
- 植物生物学 植物生物学
- 光合作用研究研究 光合作用研究
- 分子植物生理学分子植物生理学
背景情况:
- 光系统II子单元S (PsbS) 对于非光化学火 (NPQ) 非常重要,这是植物中的光保护机制.
- 了解PsbS蛋白相互作用对于阐明NPQ调节和防止光损伤至关重要.
- 基于PsbS介导的NPQ的分子机制尚不完全理解.
研究的目的:
- 在使用近距离标记的NPQ条件下,在活的阿拉比多普西斯细胞中识别PsbS相互作用蛋白.
- 为了研究光线如何影响PsbS蛋白质-蛋白质相互作用.
- 揭示NPQ的调节和与光抑制修复的潜在协调的新见解.
主要方法:
- 在稳定的Arabidopsis系中,使用TurboID与PsbS融合的靠近依赖生物化.
- 通过液体染色体质谱法 (LC-MS) 对生物化蛋白质进行定量蛋白质组分析.
- 在黑暗和高光条件下对PsbS互动体的比较分析.
主要成果:
- 确定已知的PsbS相互作用体 (Lhcb1.3,Lhcb3,Lhcb4.2) 和许多新的结合伙伴.
- 大多数PsbS相互作用是光独立的,这表明通过形状变化进行调节.
- 像TLP18.3和ZEP这样的特定蛋白质显示出光依赖调制,暗示NPQ和修复协调.
结论:
- PsbS与多样化的蛋白质网络相互作用,扩大了我们对NPQ调节的理解.
- PsbS很可能通过在甲状腺膜内的结构调整来调节NPQ.
- 光调节的相互作用表明光保护和光抑制后修复过程之间的协调反应.
相关概念视频
 02:16
Comparing Mitochondrial, Chloroplast, and Prokaryotic Genomes
16.3K
The present-day mitochondrial and chloroplast genomes have retained some of the characteristics of their ancestral prokaryotes and also have acquired new attributes during their evolution within eukaryotic cells. Like prokaryotic genomes, mitochondrial and chloroplast genomes neither bind with histone-like proteins nor show complex packaging into chromosome-like structures, as observed in eukaryotes. Unlike mitotic cell divisions observed in eukaryotic cells, mitochondria and chloroplasts...
16.3K
 01:07
Anatomy of Chloroplasts
119.4K
Green algae and plants, including green stems and unripe fruit, harbor chloroplasts—the vital organelles where photosynthesis takes place. In plants, the highest density of chloroplasts is found in the mesophyll cells of leaves.
119.4K
 02:19
Export of Mitochondrial and Chloroplast Genes
4.2K
A eukaryotic cell can have up to three different types of genetic systems: nuclear, mitochondrial, and chloroplast. During evolution, organelles have exported many genes to the nucleus; this transfer is still ongoing in some plant species. Approximately 18% of the Arabidopsis thaliana nuclear genome is thought to be derived from the chloroplast’s cyanobacterial ancestor, and around 75% of the yeast genome derived from the mitochondria’s bacterial ancestor. This export has occurred...
4.2K
 01:18
Protein Transport to the Inner Chloroplast Membrane
2.5K
Proteins targeted to the inner chloroplast membrane, or plastid proteins, are transported by two general pathways: the stop-transfer and the re-insertion or post-import pathways. Most plastid proteins carry N-terminal transit sequences and internal import sequences targeting it to the specific chloroplast subcompartment. Proteins targeted by the stop-transfer pathway have internal hydrophobic sequences that inhibit their translocation into the stroma. As a result, these precursors are arrested...
2.5K
 02:16
Light Acquisition
9.6K
In order to produce glucose, plants need to capture sufficient light energy. Many modern plants have evolved leaves specialized for light acquisition. Leaves can be only millimeters in width or tens of meters wide, depending on the environment. Due to competition for sunlight, evolution has driven the evolution of increasingly larger leaves and taller plants, to avoid shading by their neighbors with contaminant elaboration of root architecture and mechanisms to transport water and nutrients.
9.6K
 01:11
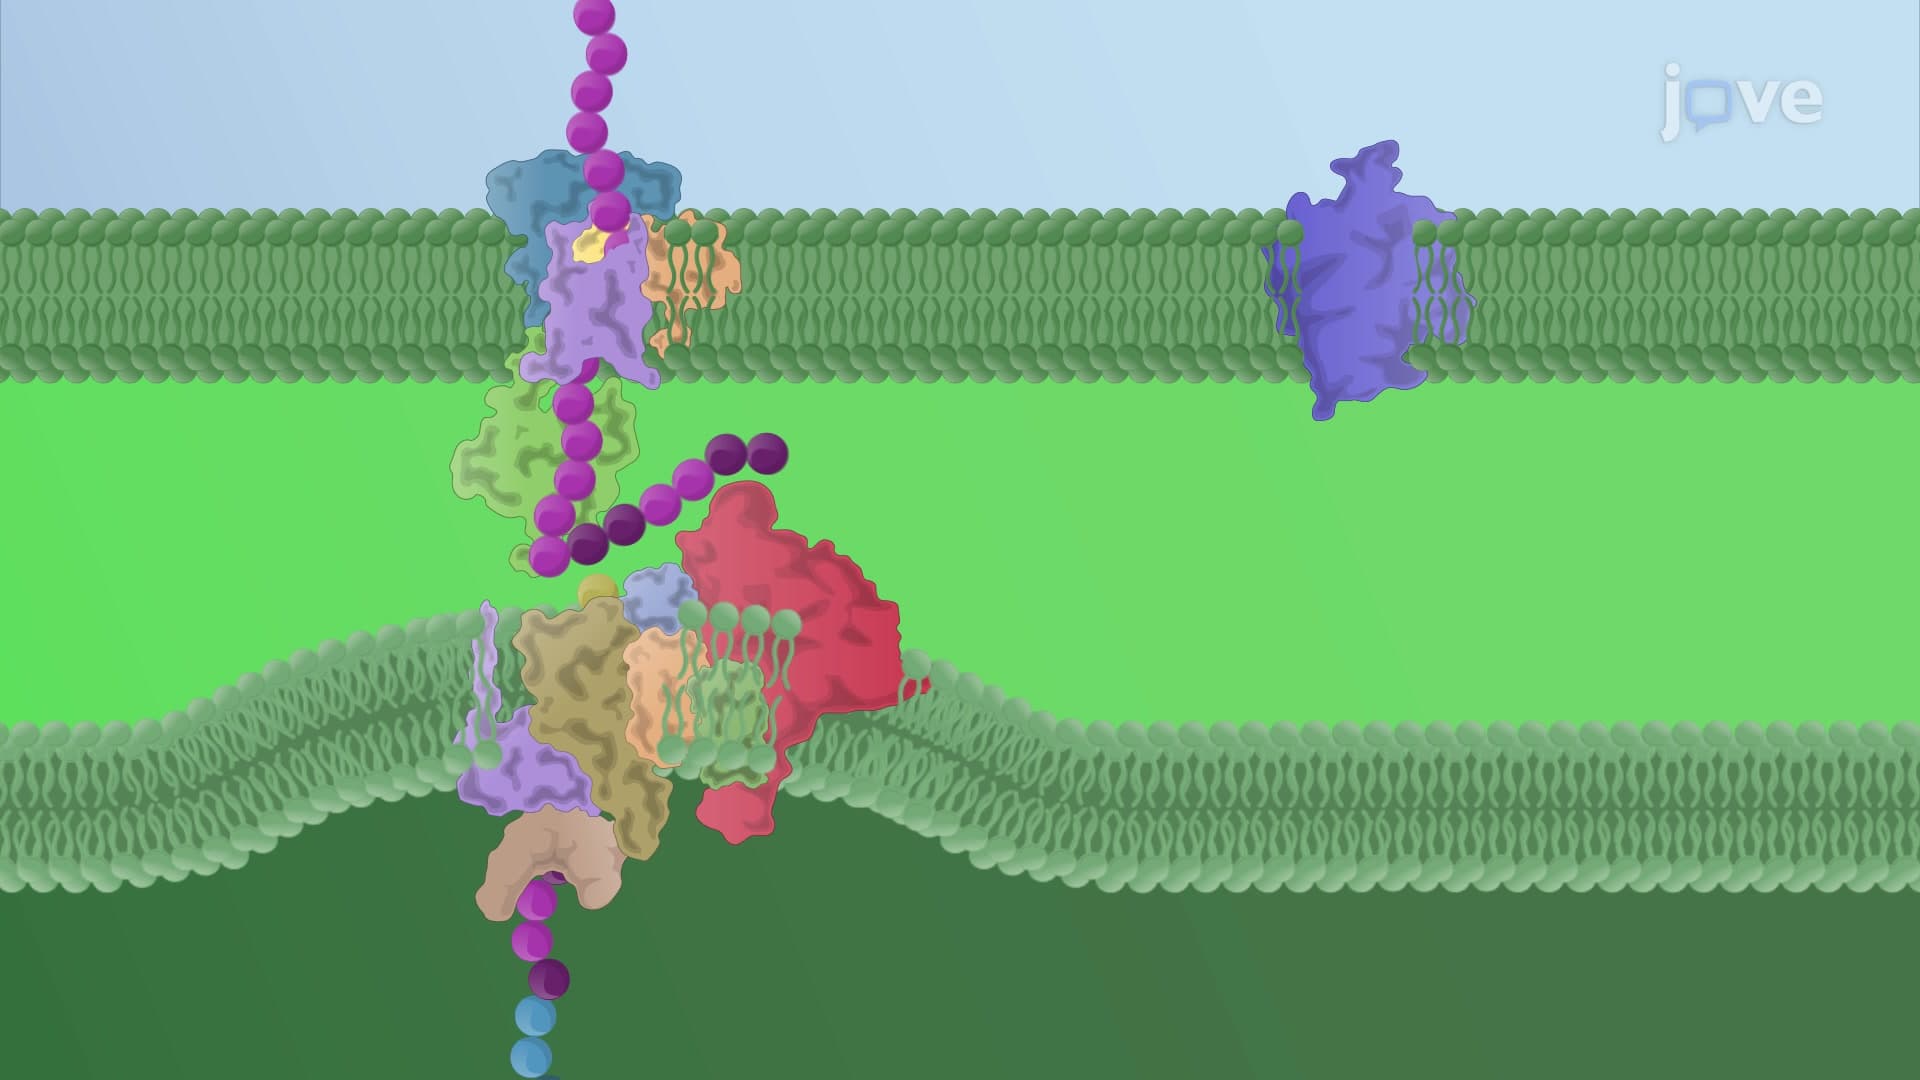
Protein Transport to the Outer Chloroplast Membrane
2.4K
Chloroplast outer membrane proteins encoded by the nucleus are synthesized in the cytosol. Soon after synthesis, they bind cytosolic factors such as 14-3-3 protein and the Hsp70 chaperones that keep these precursors in an unfolded state until their translocation.
Two models describe the mechanism of precursor recognition and entry across the outer membrane through the TOC complex. Model 1 suggests the newly synthesized precursor binds to the TOC receptor 159 and forms a complex.
Two models describe the mechanism of precursor recognition and entry across the outer membrane through the TOC complex. Model 1 suggests the newly synthesized precursor binds to the TOC receptor 159 and forms a complex.
2.4K