
综合体I在人类巨细胞被分泌能力强的细菌感染时保持了线粒体两极分化
Francisco-Javier Garcia-Rodriguez1, Paula Martinez-Oca1, Carmen Buchrieser1
1Institut Pasteur, Université Paris Cité, Biologie des Bactéries Intracellulaires, Département de Microbiologie, Paris, France.
Infection and immunity
|February 27, 2026

概括
细胞内细菌,如莱吉欧内拉肺炎菌和沙门氏菌Typhimurium破坏巨细胞呼吸,但保持线粒体膜潜力 (Δψm). 综合体I对于这种Δψm维护至关重要,作为区分毒性细菌的检查点.
科学领域:
- * 细胞和分子生物学
- * 免疫学 免疫学
- * 微生物学 微生物学
背景情况:
- * 细胞内细菌重新编程宿主细胞的能量代谢.
- *线粒体膜潜力 (Δψm) 对于细胞功能至关重要,并且在感染期间受到调节.
- * 电子输送链 (ETC) 组件在巨细胞感染期间维持 Δψm 的精确作用尚未完全理解.
研究的目的:
- * 调查电子输送链 (ETC) 组件如何在感染Legionella pneumophila* (*Lp*) 和Salmonella enterica* 血清Typhimurium (*S*.Tm) 期间维持人类巨细胞中的线粒体膜潜力 (Δψm).
- * 阐明病原体特定的策略,在早期感染阶段维持Dψm.
主要方法:
- * 结合细胞外流量分析与单细胞实时成像.
- *研究了原发性人类单细胞衍生的巨细胞,感染了Lp或S*TM.
- *利用ETC复合物 (I,II,III,IV) 和分泌系统突变的系统性抑制.
主要成果:
- * 无论是*Lp*还是*S*.Tm感染,都降低了氧气消耗率,但保留了Δψm.
- *复合I是唯一需要在感染毒性细菌期间维护Δψm的,与分泌不足的菌株不同.
- *复合II在维持Dψm方面发挥了感染驱动的作用,而复合III和IV在所有条件下都是必不可少的.
结论:
- *I复合体作为一个关键的生物能检查点,通过维持Δψm来区分毒性细菌和缺乏分泌的细胞内细菌.
- * *Lp*和*S*.Tm采用不同的机制,在早期感染期间保持巨细胞线粒体两极分化.
- * 了解这些病原体特异性策略,可以了解宿主-病原体相互作用和宿主防御机制.
相关概念视频
 01:28
The Inner Mitochondrial Membrane
4.8K
The inner mitochondrial membrane is the primary site of ATP synthesis. The inner membrane domain that forms a smooth layer adjacent to the outer membrane is called the inner boundary membrane. This domain contains membrane transporters that drive metabolites in and out of the mitochondria. In contrast, the inner membrane network that invaginates into the matrix space is called the cristae membrane. This domain accounts for principle mitochondrial function as it accommodates the protein...
4.8K
 01:45
Mitochondrial Membranes
17.5K
A single mitochondrion is a bean-shaped organelle enclosed by a double-membrane system. The outer membrane of mitochondria is smooth and contains many porins - the integral membrane transporters. Porins enable free diffusion of ions and small uncharged molecules through the outer mitochondrial membrane but limit the transport of molecules larger than 5000 Daltons. Further, the outer mitochondrial membrane forms a unique structure called membrane contact sites with other subcellular organelles,...
17.5K
 01:19
Translocation of Proteins into the Mitochondria
13.5K
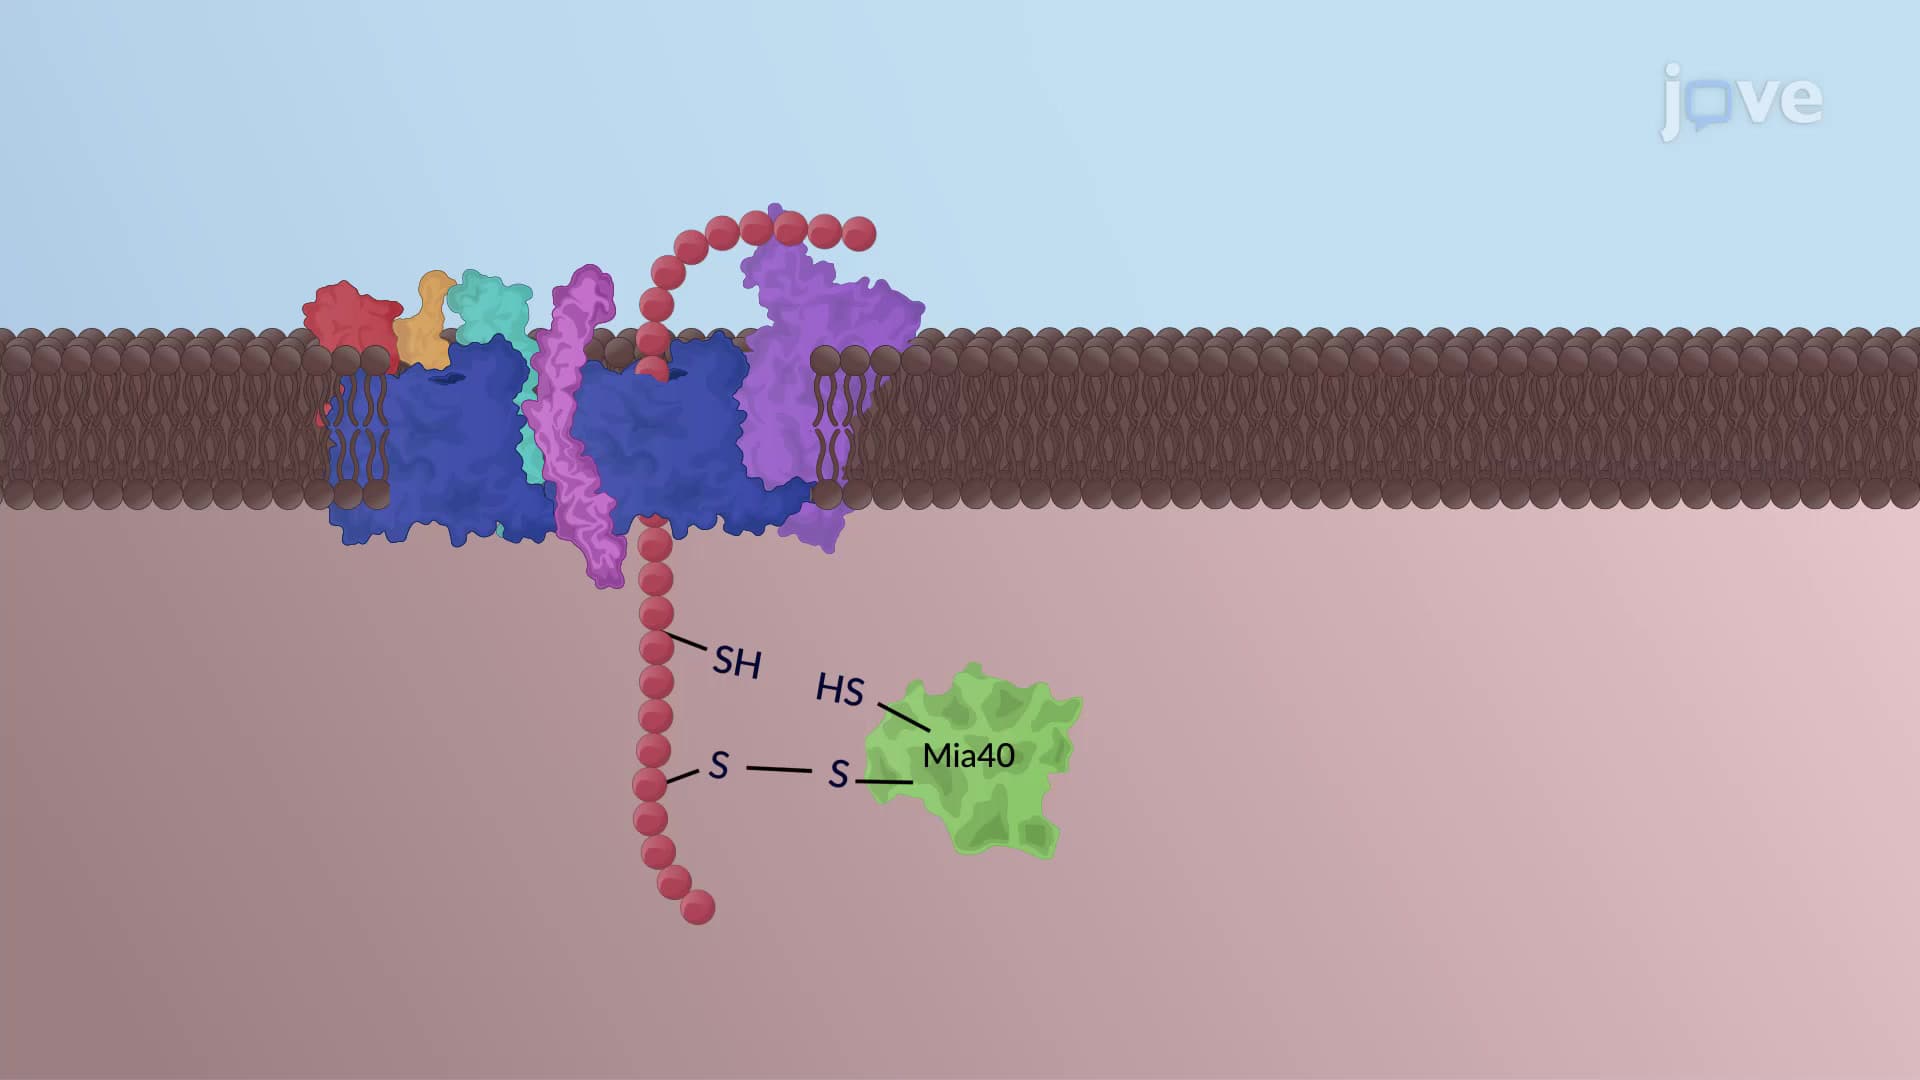
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
13.5K
 01:12
Porin Insertion in the Outer Mitochondrial Membrane
5.0K
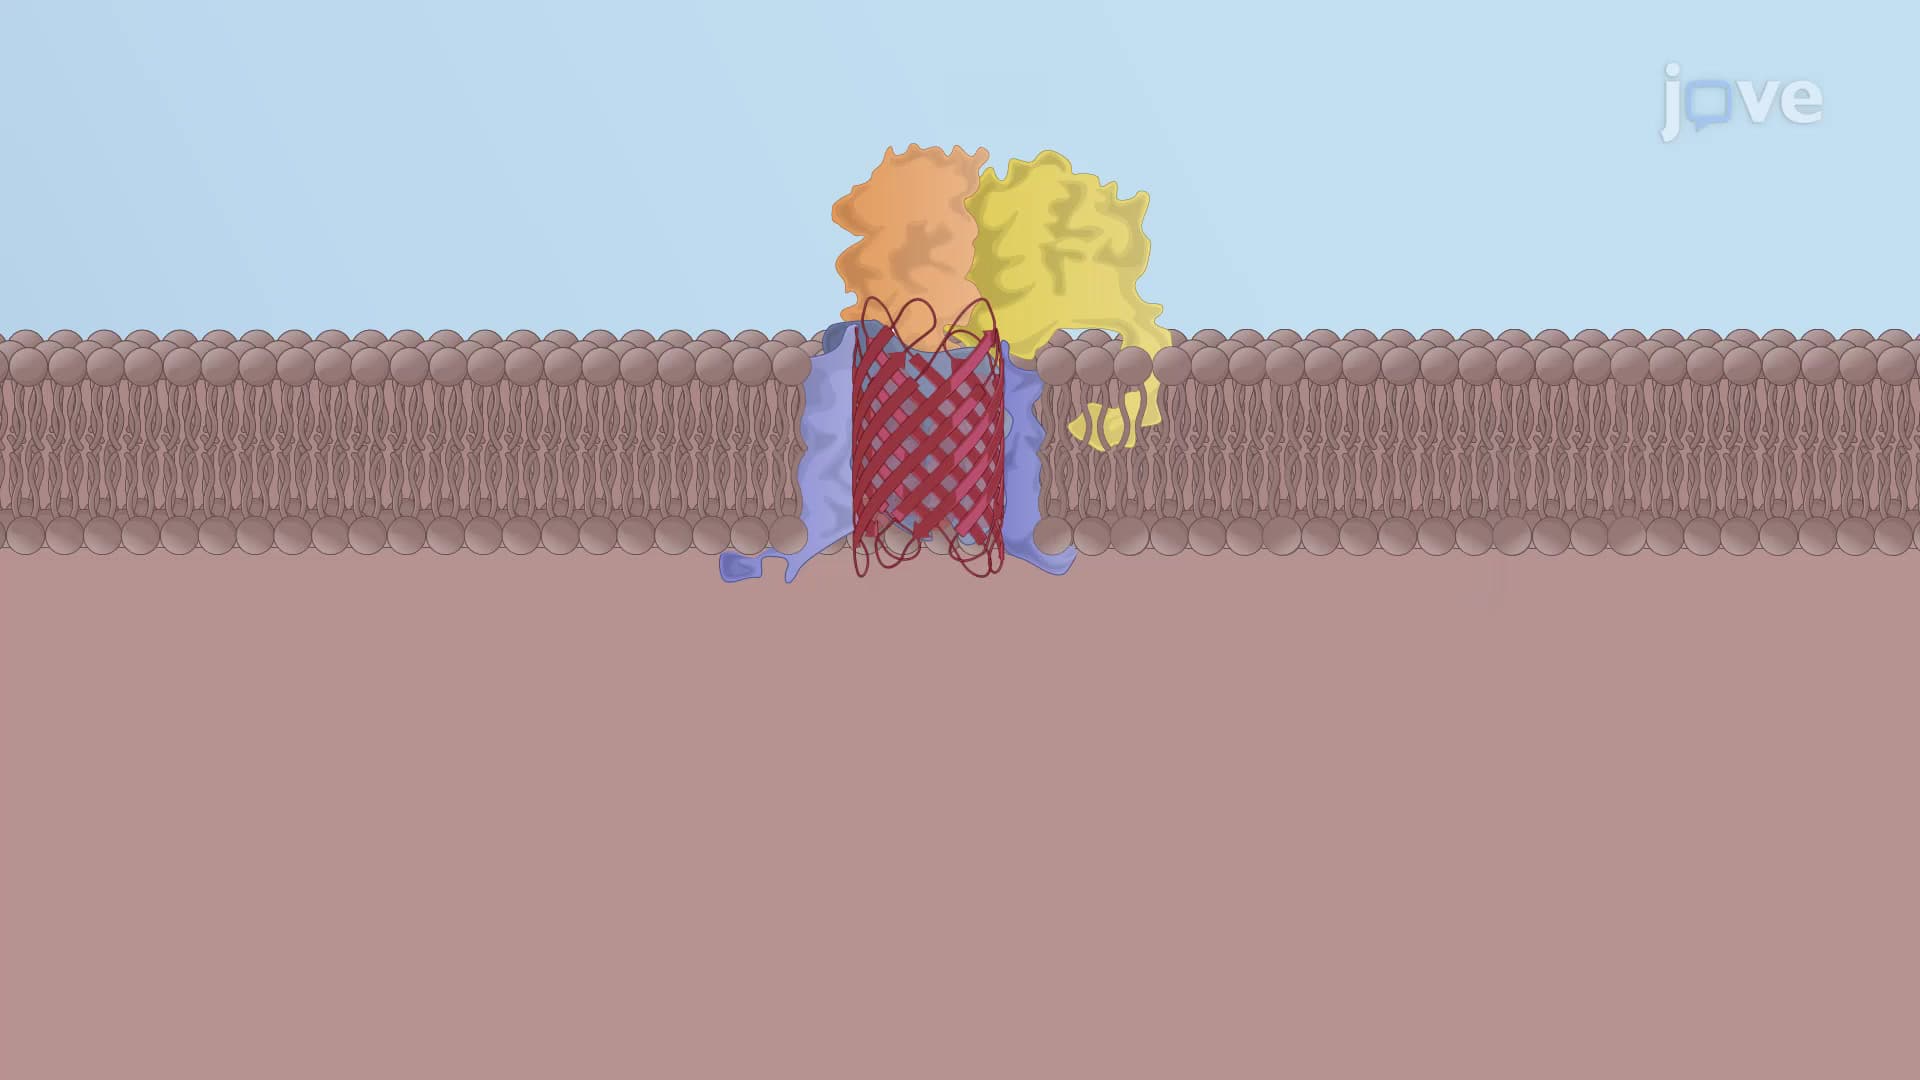
Porins are beta-barrel proteins translocated to the mitochondrial outer membrane through the TOM complex into the intermembrane space. Porin precursors bind TIM chaperones within the intermembrane space and are guided to the Sorting and Assembly Machinery complex or SAM complex on the outer mitochondrial membrane.
Three models describe the assembly of porins by the SAM complex and their insertion into the outer membrane. Model 1 suggests that porins are assembled outside the SAM channel as the...
Three models describe the assembly of porins by the SAM complex and their insertion into the outer membrane. Model 1 suggests that porins are assembled outside the SAM channel as the...
5.0K