相关实验视频
Updated: Jun 30, 2026
09:42
Using SecM Arrest Sequence as a Tool to Isolate Ribosome Bound Polypeptides
Published on: June 19, 2012
翻转SecG的膜拓与SecA依赖的前蛋白转位相结合
K Nishiyama1, T Suzuki, H Tokuda
1Institute of Molecular and Cellular Biosciences, University of Tokyo, Japan.
Cell
|April 5, 1996

概括
对于大肠杆菌前蛋白转位酶的效率来说,SecG蛋白质拓逆转是至关重要的. 这个过程与SecA循环相结合,对于蛋白质跨膜转移至关重要.
科学领域:
- 分子生物学分子生物学
- 细胞生物学 细胞生物学
- 生物化学 生物化学
背景情况:
- 大肠杆菌前蛋白转位酶由Seca和SecY/E/G复合体组成,促进蛋白质穿过内膜的运输.
- SecA利用ATP驱动的膜插入和脱入周期,将前蛋白传递到SecY/E通道.
- SecG显著提高了这种转位酶系统的效率.
研究的目的:
- 研究SecG在前蛋白转位中的作用.
- 阐明SecG在转位过程中的动态行为和拓.
- 了解SecG,SecA和转位酶机制之间的功能合.
主要方法:
- 利用对SecG的C端区域的抗体来检测其可访问性.
- 采用了来自大肠杆菌的长膜囊泡.
- 操纵ATP水解以阻止和观察转位中间体.
主要成果:
- 针对SecG的C端的抗体抑制了转位,表明其参与.
- SecG的C终端区域在启动后的转位阻塞后,从内部暴露到外部暴露状态转移.
- 一个独特的SecG区域表现出拓反转,紧密结合转位和SecA的插入-卸载周期.
结论:
- 在前蛋白转位过程中,SecG经历了拓反转.
- 这种SecG的动态构造变化对于转位酶的效率至关重要.
- SecG的功能循环与SeCA的ATP依赖活性密切相关.
相关概念视频
 01:20
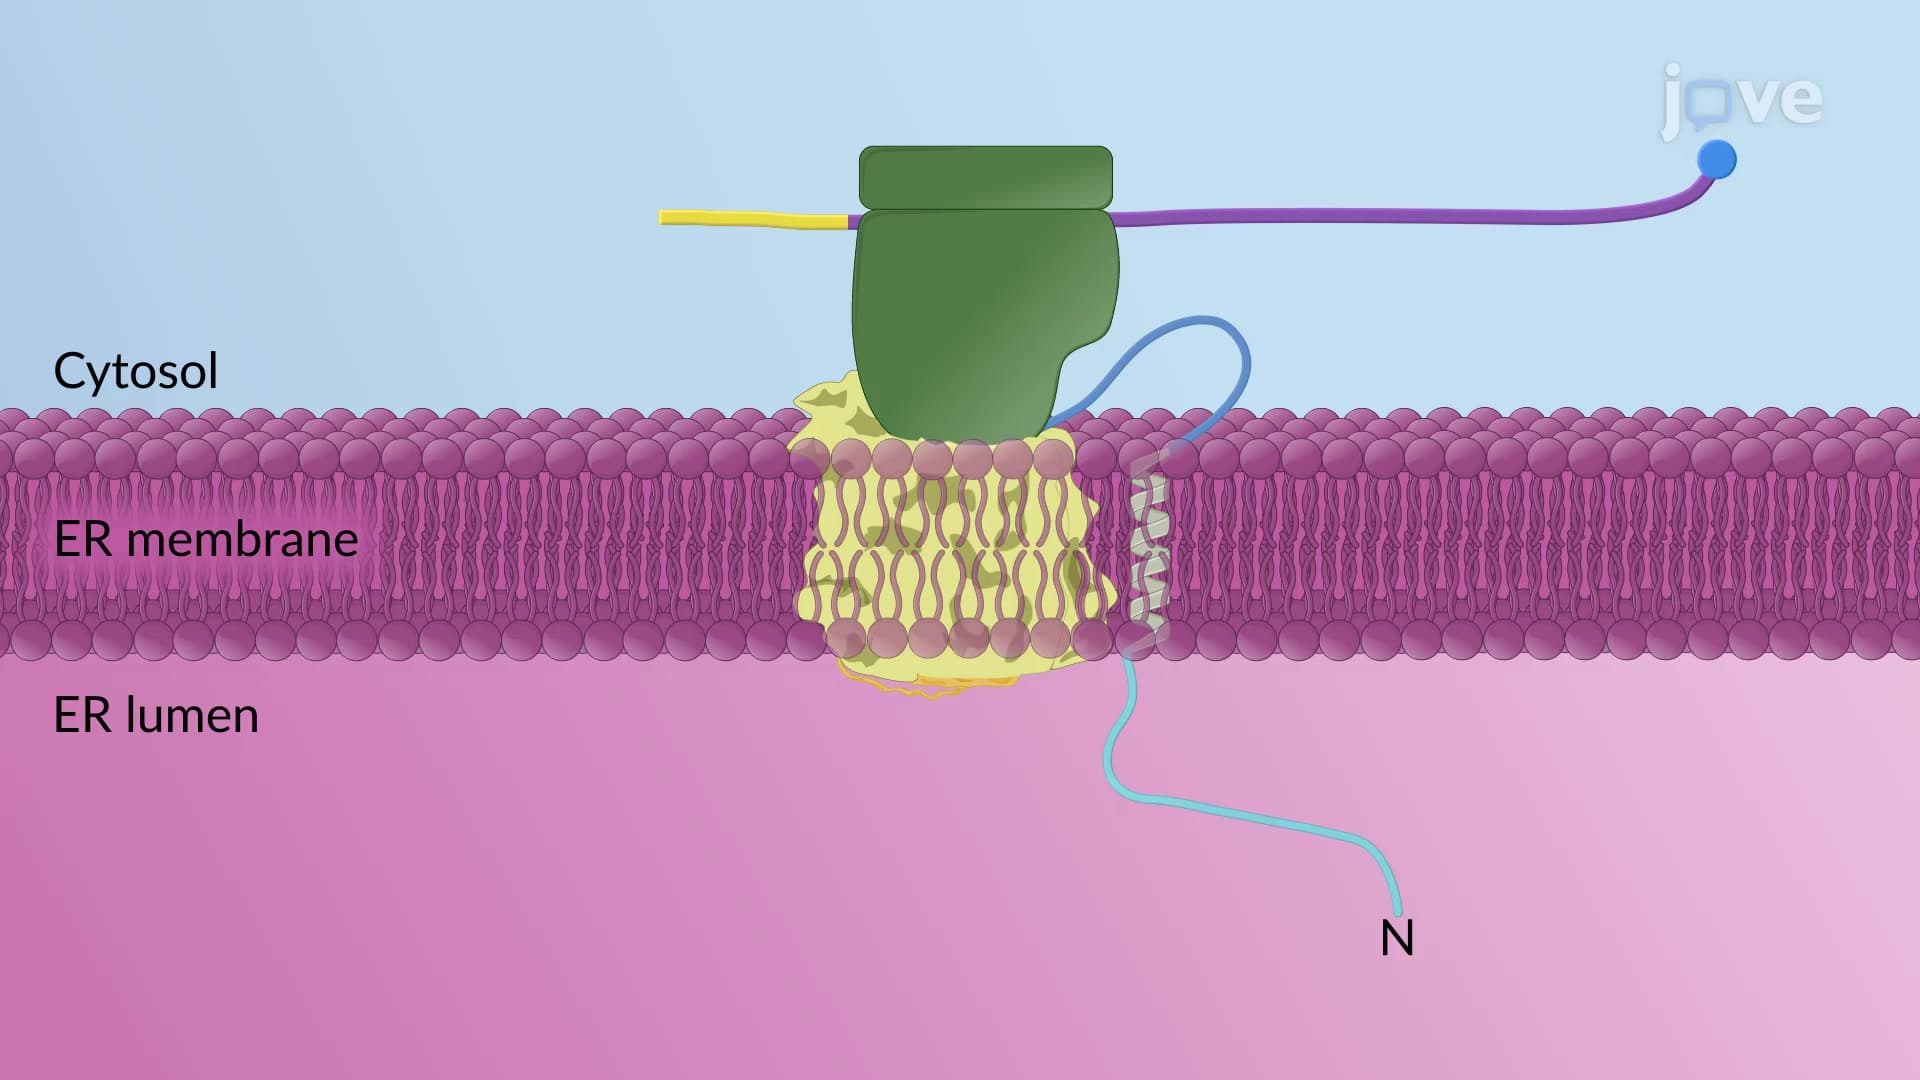
Cotranslational Protein Translocation
Translocation of proteins across membranes is an ancient process that occurs even in bacteria and archaebacteria. In fact, the components of the translocation machinery are still conserved between prokaryotes and eukaryotes.
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:26
Insertion of Single-pass Transmembrane Proteins in the RER
Integral membrane proteins are proteins adhered to the lipid bilayer of a cell organelle or membrane. They can be of two types: transmembrane integral proteins that span the lipid bilayer and monotopic proteins that are attached to either side of the membrane but do not pass through it.
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
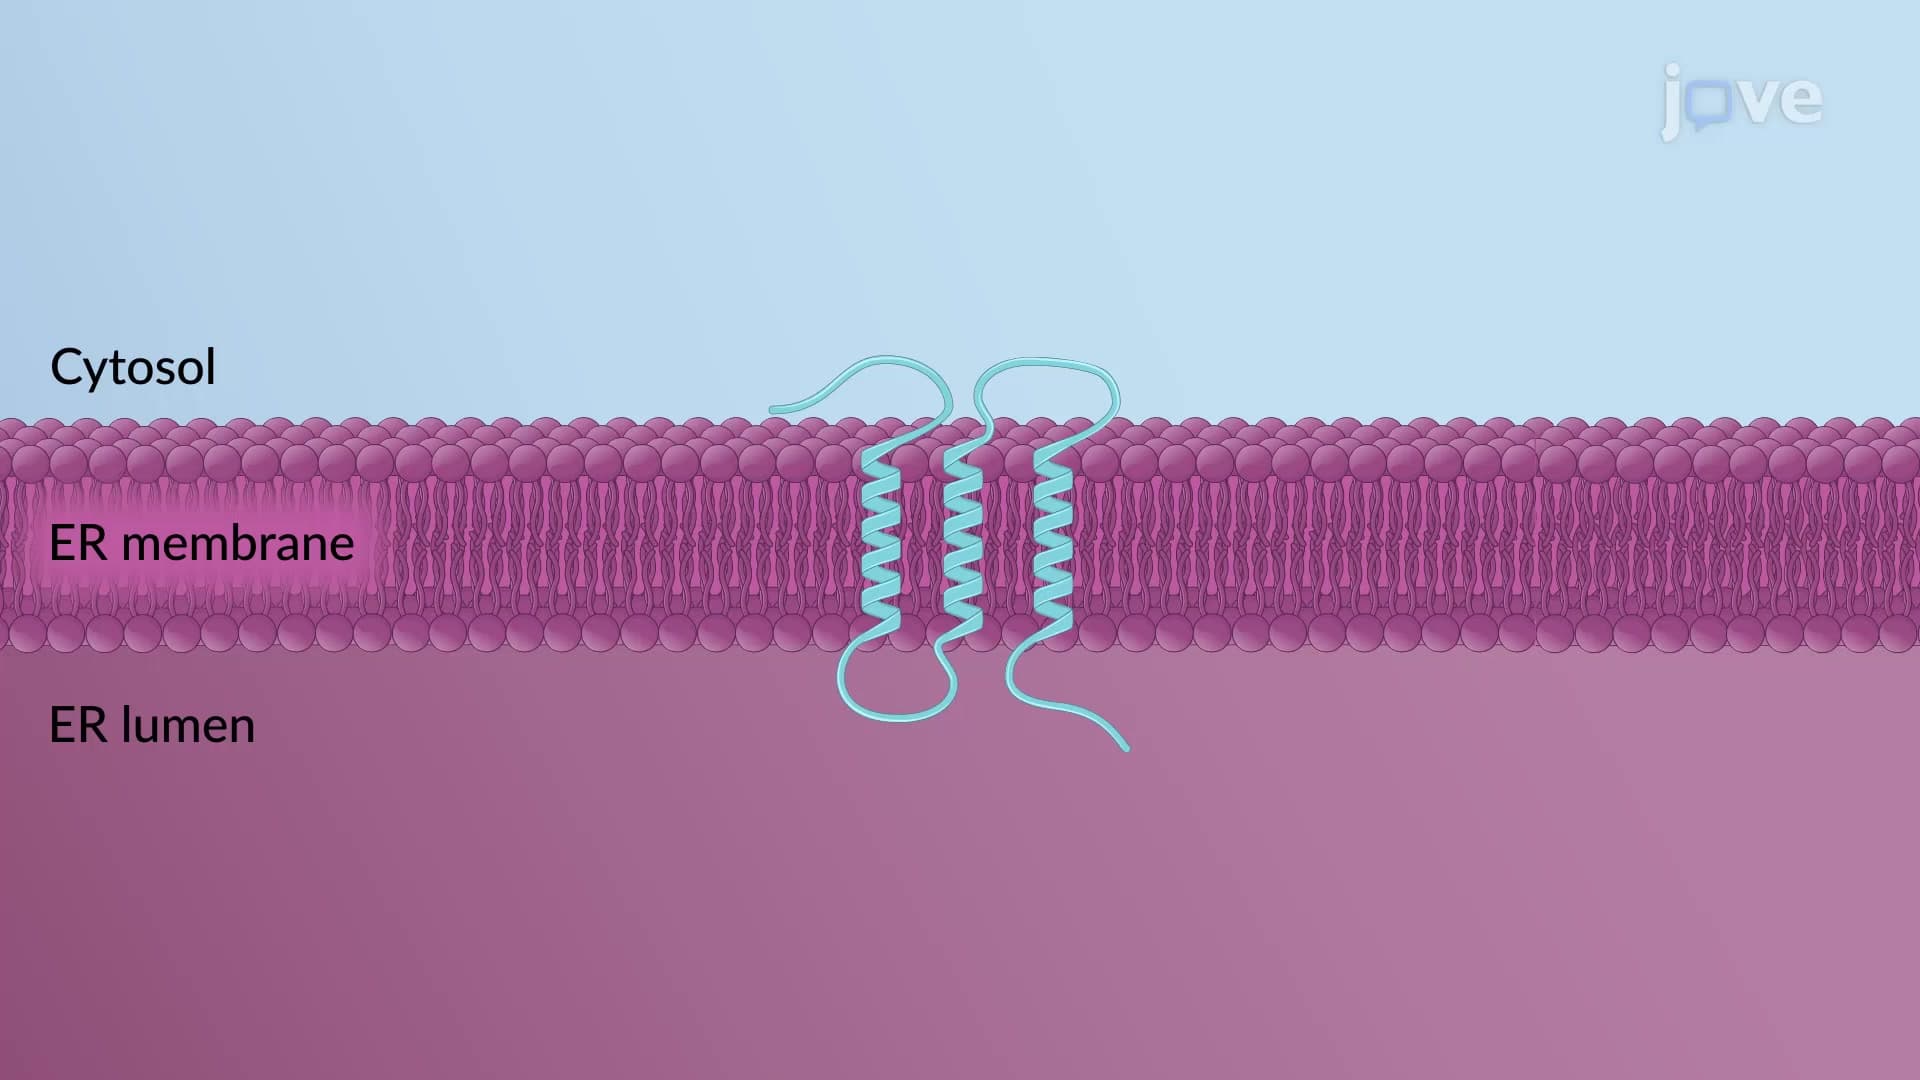 01:29
Insertion of Multi-pass Transmembrane Proteins in the RER
The rough ER membrane synthesizes, assembles, and embeds transmembrane proteins in diverse topologies. These proteins function as transporters or channels and can remain in the ER membrane or are sent to the Golgi complex, lysosome, and cell membrane.
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
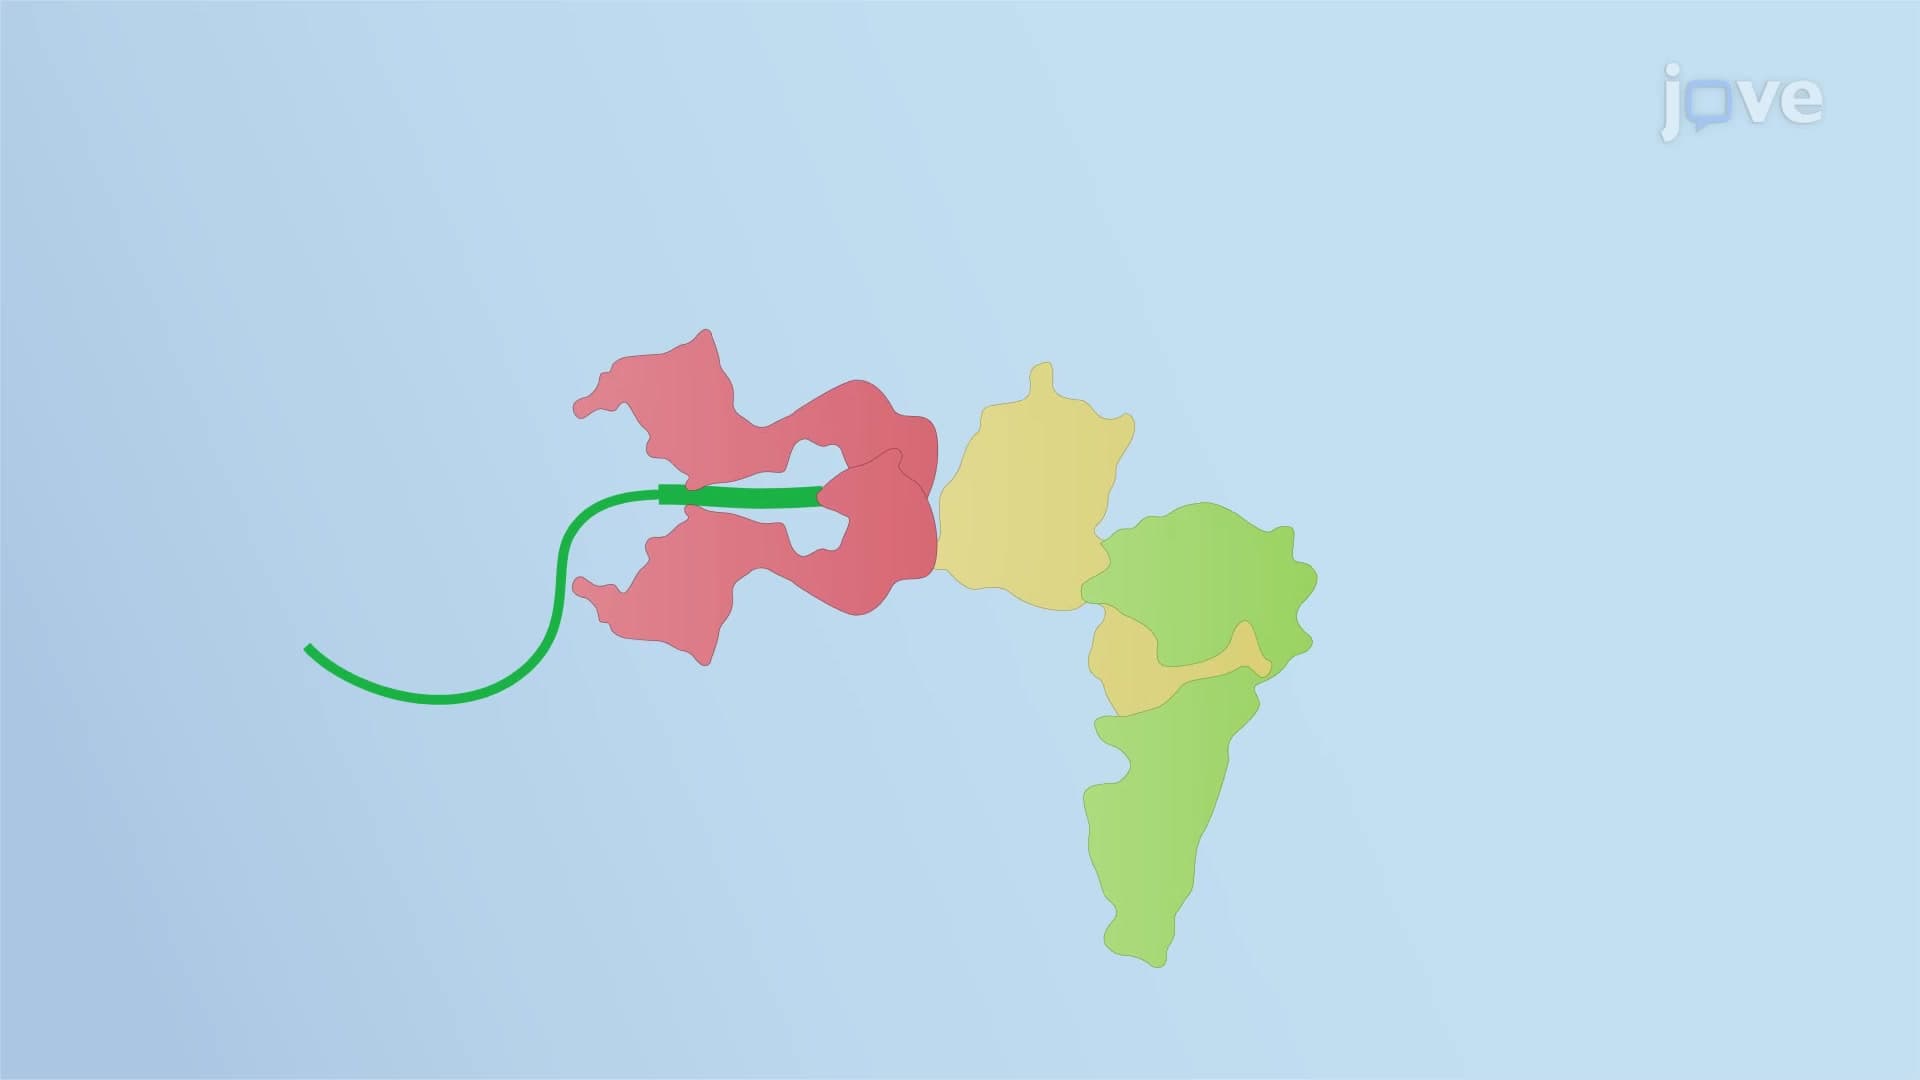 01:45
Tail-anchoring of Proteins in the ER Membrane
Tail-anchored, or TA, proteins are estimated to make up to 3-5% of membrane proteins found in the eukaryotic cell. Such proteins have a single transmembrane domain located approximately 30 amino acid residues upstream from the C-terminal end. As a result, the signal recognition particle (SRP) cannot guide a TA protein to the ER membrane for cotranslational insertion. Hence, they are integrated into the ER membrane post-translationally using their C-terminal end as the anchor. TA proteins...
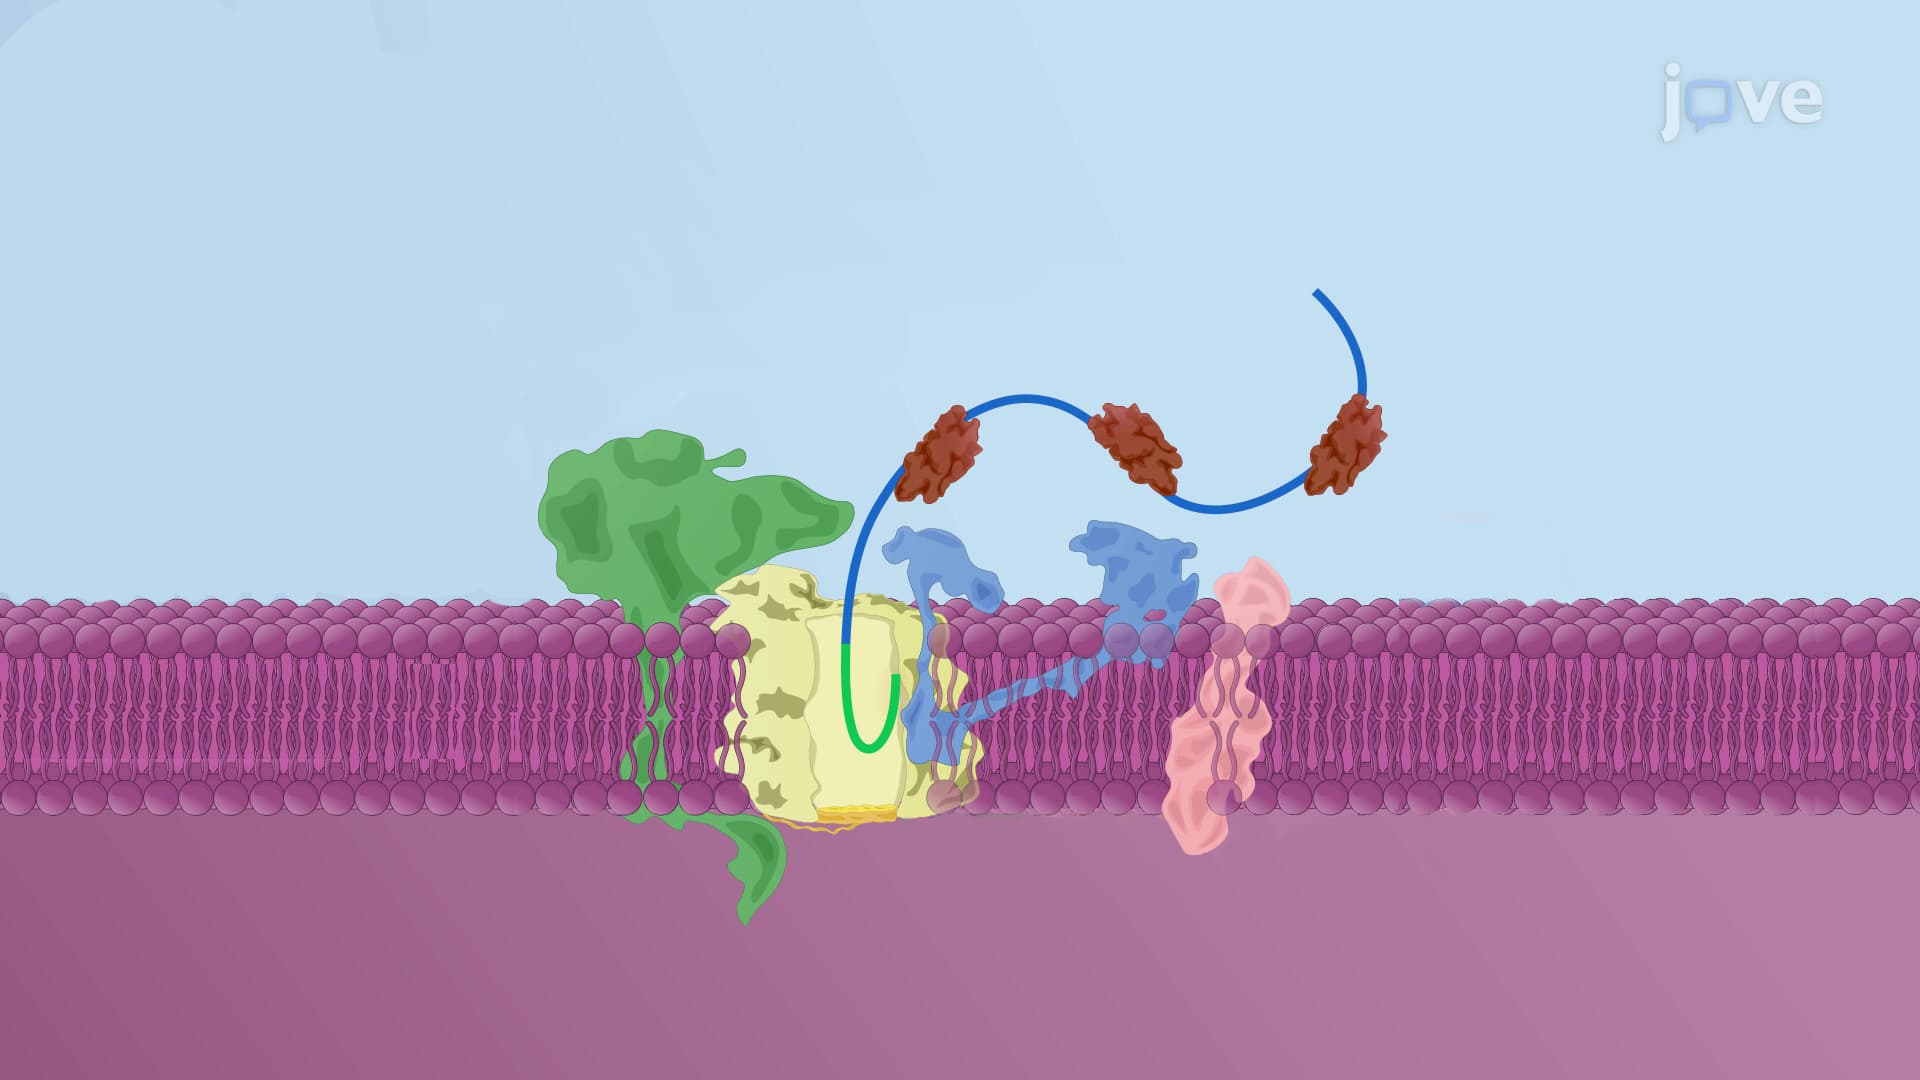 01:27
Post-translational Translocation of Proteins to the RER
A sizable fraction of proteins destined for ER are first synthesized in the cell cytosol and then transported across the ER membrane–a process called post-translational translocation. Similar to cotranslationally translocated proteins, these proteins also use the Sec translocon complex to enter the ER lumen.
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
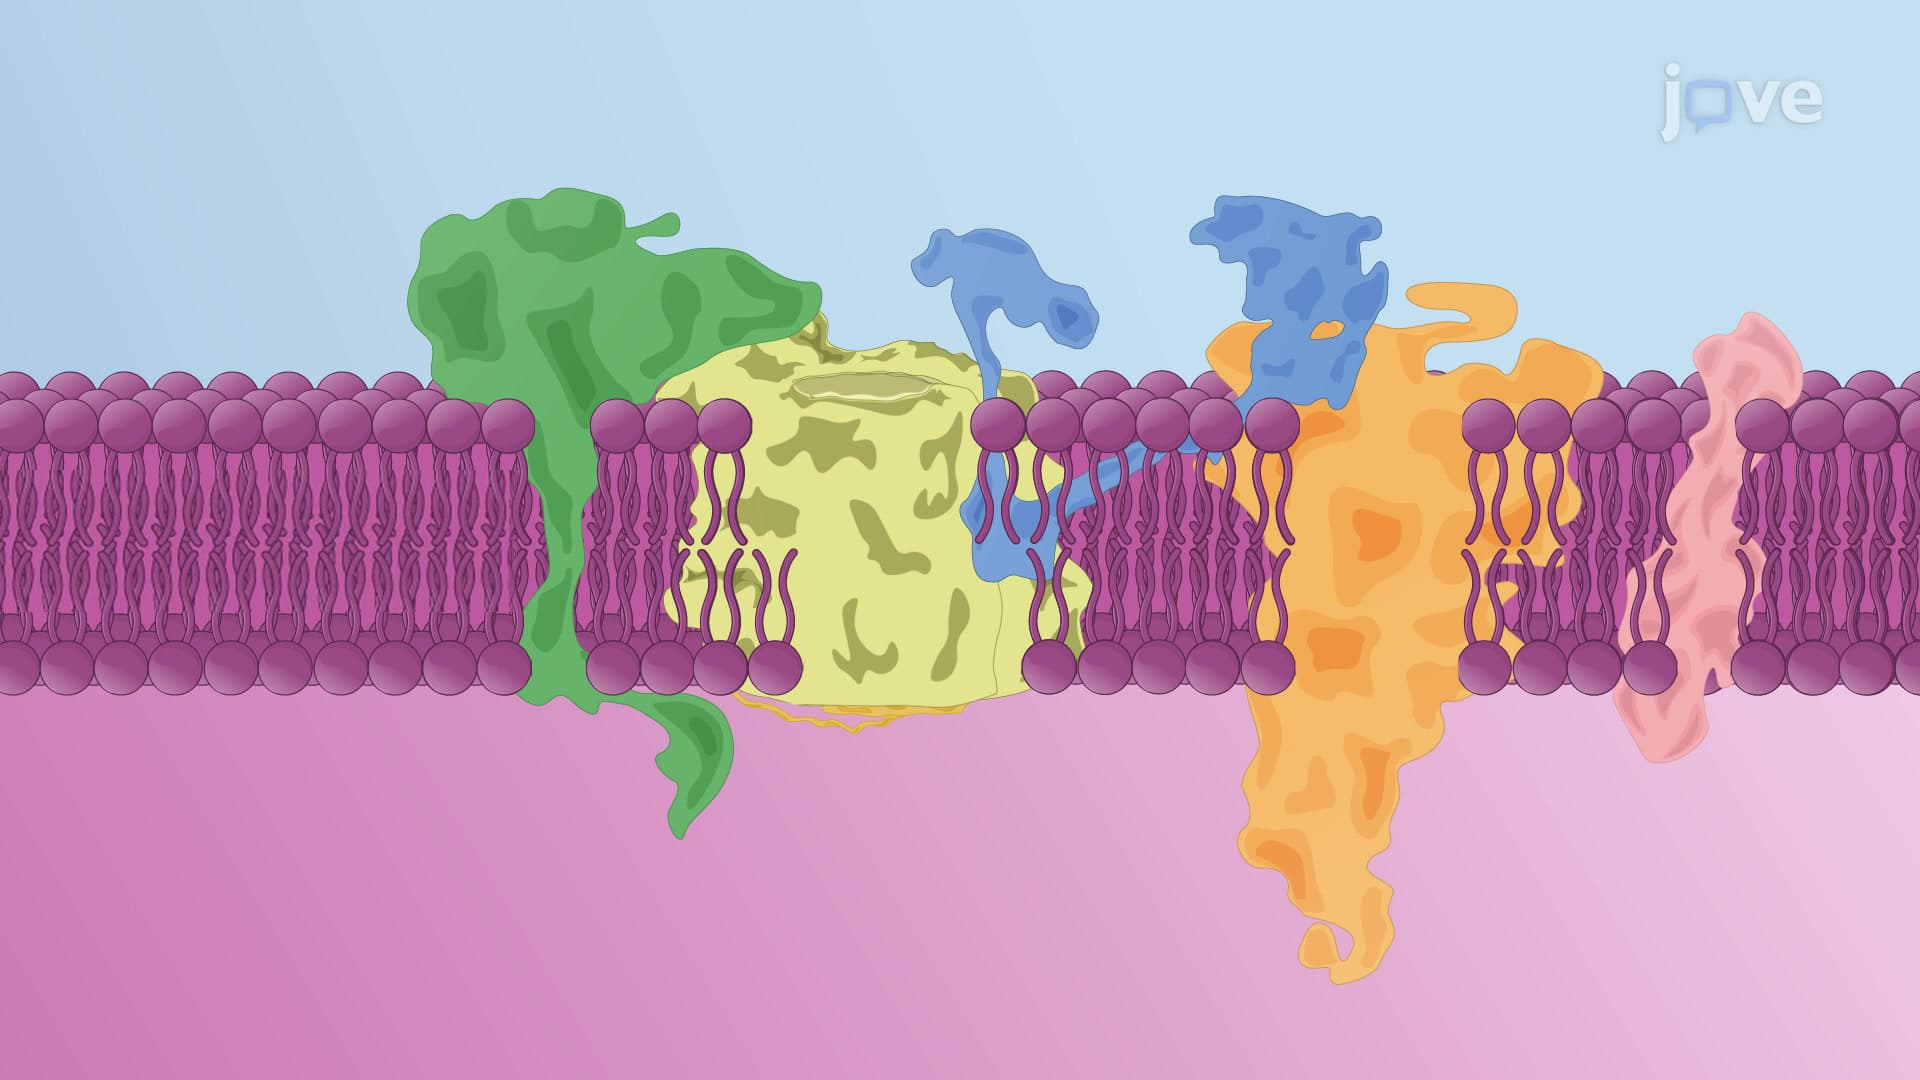 01:28
Protein Translocation Machinery on the ER Membrane
The translocon complex situated on the ER membrane is the main gateway for the protein secretory pathway. It facilitates the transport of nascent peptides into the ER lumen and their insertion into the ER membrane.
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.