
概括
类细胞通过占用受体的绝对数量来感知形态原度,而不是它们的比例. 这一发现揭示了细胞在早期发育过程中如何解释形态变异梯度.
科学领域:
- 发育生物学是发展生物学.
- 细胞信号传递 细胞信号传递
- 分子遗传学 分子遗传学
背景情况:
- 活动素在Xenopus发育过程中起到形态原的作用,触发明显的中皮基因表达.
- 了解细胞如何解释形态原度对于破译发育过程至关重要.
研究的目的:
- 调查Xenopus芽细胞识别和响应不同度的形态原活性蛋白的机制.
- 为了确定细胞是否使用受体占用数或比率来感知连接体度.
主要方法:
- 自然标记的活性素与Xenopus细胞的结合.
- 量化每个细胞中绑定活性素分子的绝对数量.
- 与特定基因激活模式 (Xbra和Xgsc) 相关的受体占用率.
主要成果:
- 细胞根据激素度以剂量依赖的方式激活不同的中皮基因.
- 一个单个受体类型的占用水平决定了基因表达切换.
- 细胞通过占用受体的绝对数量 (例如100-300个分子) 来感知连接体度,而不是占用与未占用受体的比例.
- 长时间的受体占用时间解释了观察到的拉切特效应.
结论:
- 细胞对形态基因梯度的解释依赖于占用受体的绝对数量.
- 这种机制为了解早期胚胎发育中的形态基因梯度形成和解释提供了一个新的框架.
- 这些发现特别适用于早期发展的快速和精确的模式需求.
相关概念视频
 02:32
Position-effect Variegation
5.6K
In 1928, a German botanist Emil Heitz observed the moss nuclei with a DNA binding dye. He observed that while some chromatin regions decondense and spread out in the interphase nucleus, others do not. He termed them euchromatin and heterochromatin, respectively. He proposed that the heterochromatin regions reflect a functionally inactive state of the genome. It was later confirmed that heterochromatin is transcriptionally repressed, and euchromatin is transcriptionally active chromatin.
5.6K
 02:35
Chromatin Position Affects Gene Expression
22.5K
Chromatin is the massive complex of DNA and proteins packaged inside the nucleus. The complexity of chromatin folding and how it is packaged inside the nucleus greatly influences access to genetic information. Generally, the nucleus' periphery is considered transcriptionally repressive, while the cell's interior is considered a transcriptionally active area.
Topologically Associated Domains (TADs)
The 3-dimensional positioning of chromatin in the nucleus influences the...
Topologically Associated Domains (TADs)
The 3-dimensional positioning of chromatin in the nucleus influences the...
22.5K
 03:14
Notch Signaling Pathway
4.6K
The Notch signaling pathway is a major intracellular signaling pathway that is highly conserved over a broad spectrum of metazoan species. It stands unique from other intracellular signaling mechanisms in animals because notch protein itself acts as the receptor as well as the primary signaling molecule.
The Notch gene came into the limelight in 1914 after the discovery that its mutation in Drosophila melanogaster leads to a serrated (or "notched") wing margin phenotype. It was not...
The Notch gene came into the limelight in 1914 after the discovery that its mutation in Drosophila melanogaster leads to a serrated (or "notched") wing margin phenotype. It was not...
4.6K
 01:21
Cell Polarization by Rho Proteins
3.2K
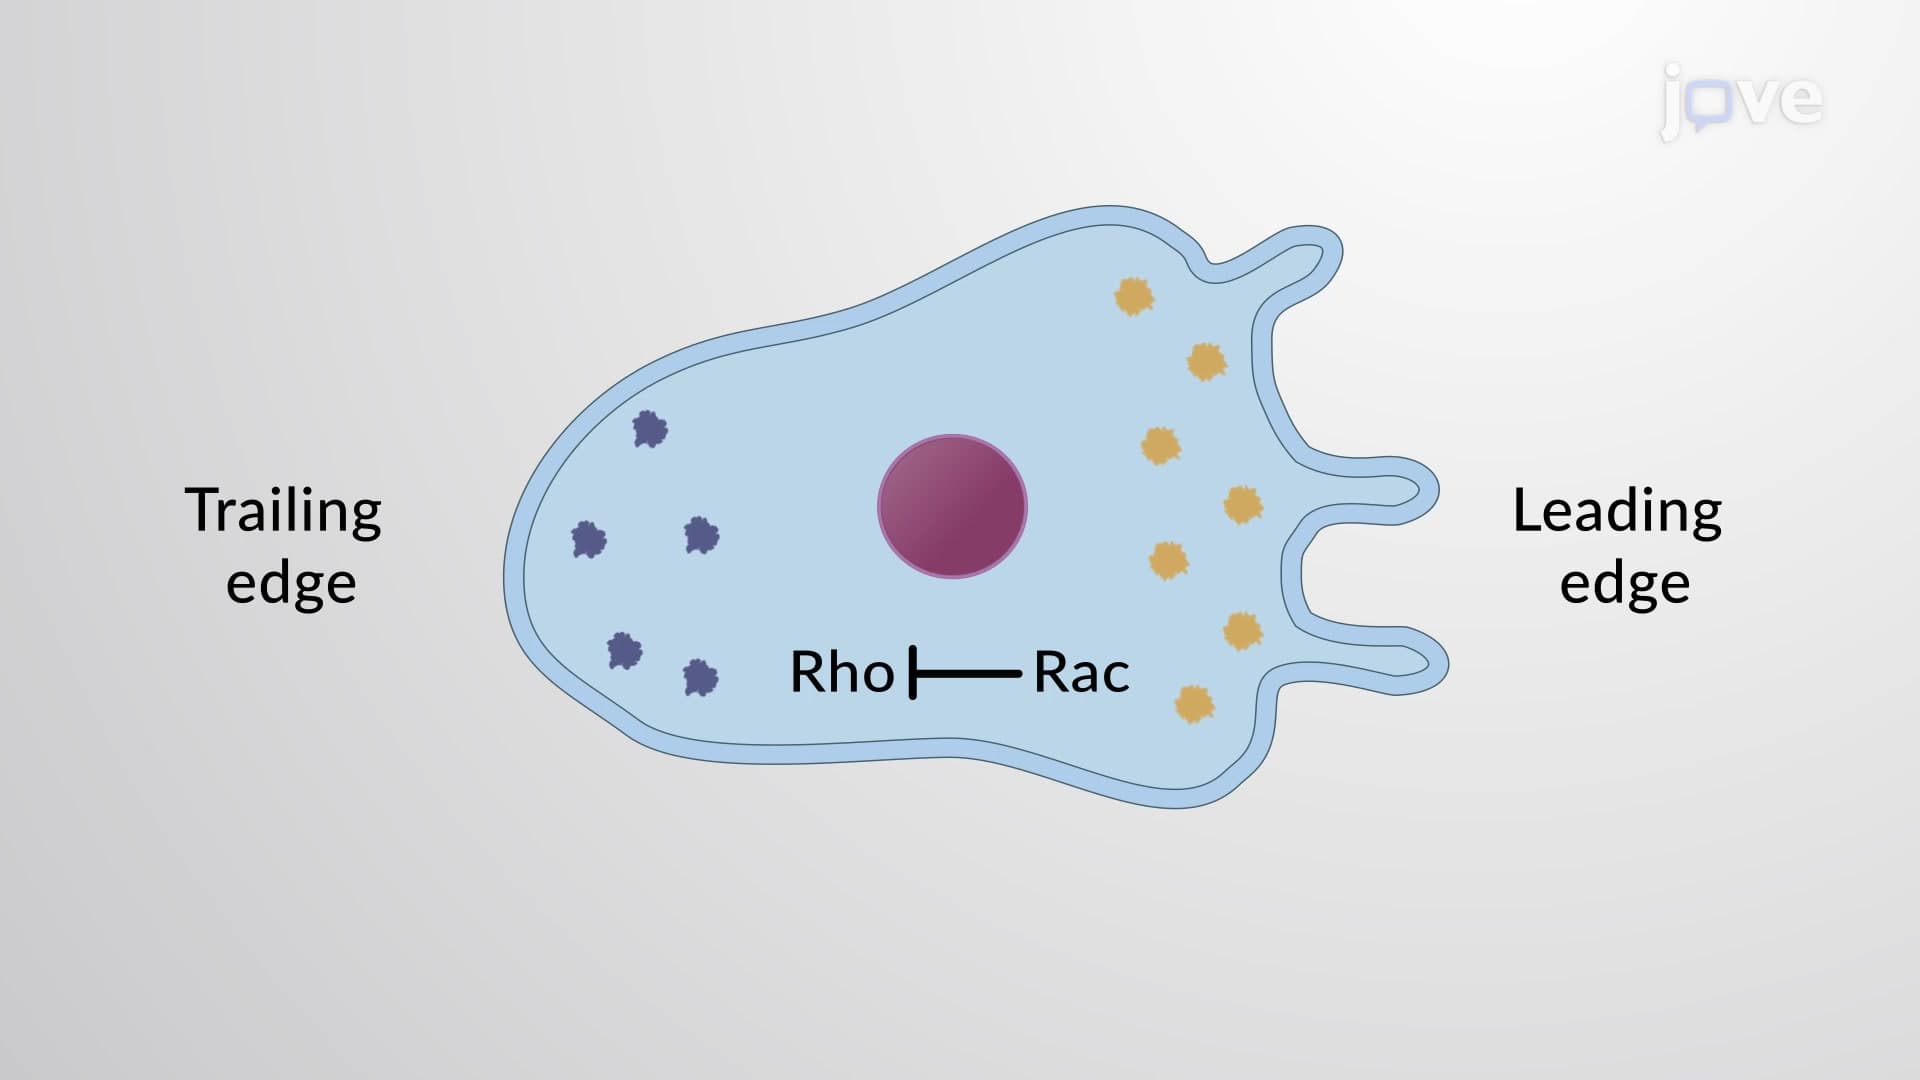
Cell polarity is the asymmetric distribution of cellular and membrane components, making one side of the cell different from the other. This polarity is essential to many processes such as embryogenesis, axon migration, glucose transport across epithelial cells, and directional cell migration. A migrating cell responds to intracellular or extracellular signals via molecular cascades that reorganize the actin cytoskeleton to establish this polarity. In these cells, the Rho family proteins Cdc42,...
3.2K
 01:16
TGF - β Signaling Pathway
7.2K
The TGF-β signaling pathway regulates cell growth, differentiation, adhesion, motility, and development. TGF-β ligands that induce TGF-β signaling are synthesized in their latent form. Several proteases or cell surface receptors such as integrins act upon the latent form, releasing the active ligand. There are three types of mammalian TGF-βs: (TGF-β1, TGF-β2, and TGF-β3) that bind as homodimers or heterodimers to TGF-β receptors. The TGF-β receptors...
7.2K
 01:15
Activation of Integrins
4.4K
Integrins bind ligands and transmit information from outside the cell to inside or vice-versa through an "outside-in signaling" or "inside-out signaling."
In "outside-in signaling," external factors in the extracellular space bind to exposed ligand binding sites on integrins. This causes the inactive protein to undergo a conformational change to become active. Integrins are often clustered on the cell membrane. Repetitive and regularly spaced ligand binding...
In "outside-in signaling," external factors in the extracellular space bind to exposed ligand binding sites on integrins. This causes the inactive protein to undergo a conformational change to become active. Integrins are often clustered on the cell membrane. Repetitive and regularly spaced ligand binding...
4.4K