Related Experiment Video
Updated: Aug 3, 2026

Transmembrane Domain Oligomerization Propensity determined by ToxR Assay
Published on: May 26, 2011
Roles of multimerization and membrane association in the proteolytic functions of FtsH (HflB)
1Institute for Virus Research, Kyoto University, Kyoto 606-8507, Japan yakiyama@virus.kyoto-u.ac.jp.

Abstract:
FtsH (HflB) is an Escherichia coli ATP-dependent protease that degrades some integral membrane and cytoplasmic proteins. While anchored to the cytoplasmic membrane by the two transmembrane (TM) segments near the N-terminus, it has a large cytoplasmic domain. The N-terminal region also has a role in homo-oligomerization of this protein. To study the significance of the membrane integration and oligomer formation, we constructed FtsH derivatives in which the N-terminal region had been deleted or replaced with either the leucine zipper sequence from Saccharomyces cerevisiae GCN4 protein or TM regions from other membrane proteins. The cytoplasmic domain, which was monomeric and virtually inactive, was converted, by the attachment of the leucine zipper, to an oligomer with proteolytic function against a soluble, but not a membrane-bound substrate. In contrast, chimeric TM-FtsH proteins were active against both substrate classes. We suggest that the cytoplasmic domain has intrinsic but weak self-interaction ability, which becomes effective with the aid of the leucine zipper or membrane tethering, and that membrane association is essential for FtsH to degrade integral membrane proteins.
Related Concept Videos
 02:41
Protein Complex Assembly
Many viruses self-assemble into a fully functional unit using the infected host cell to...
 01:57
Protein Complexes with Interchangeable Parts
The SCF ubiquitin ligase is a protein complex of five individual proteins. This complex attaches ubiquitin to other target proteins to mark them for degradation. In order to...
 01:19
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:29
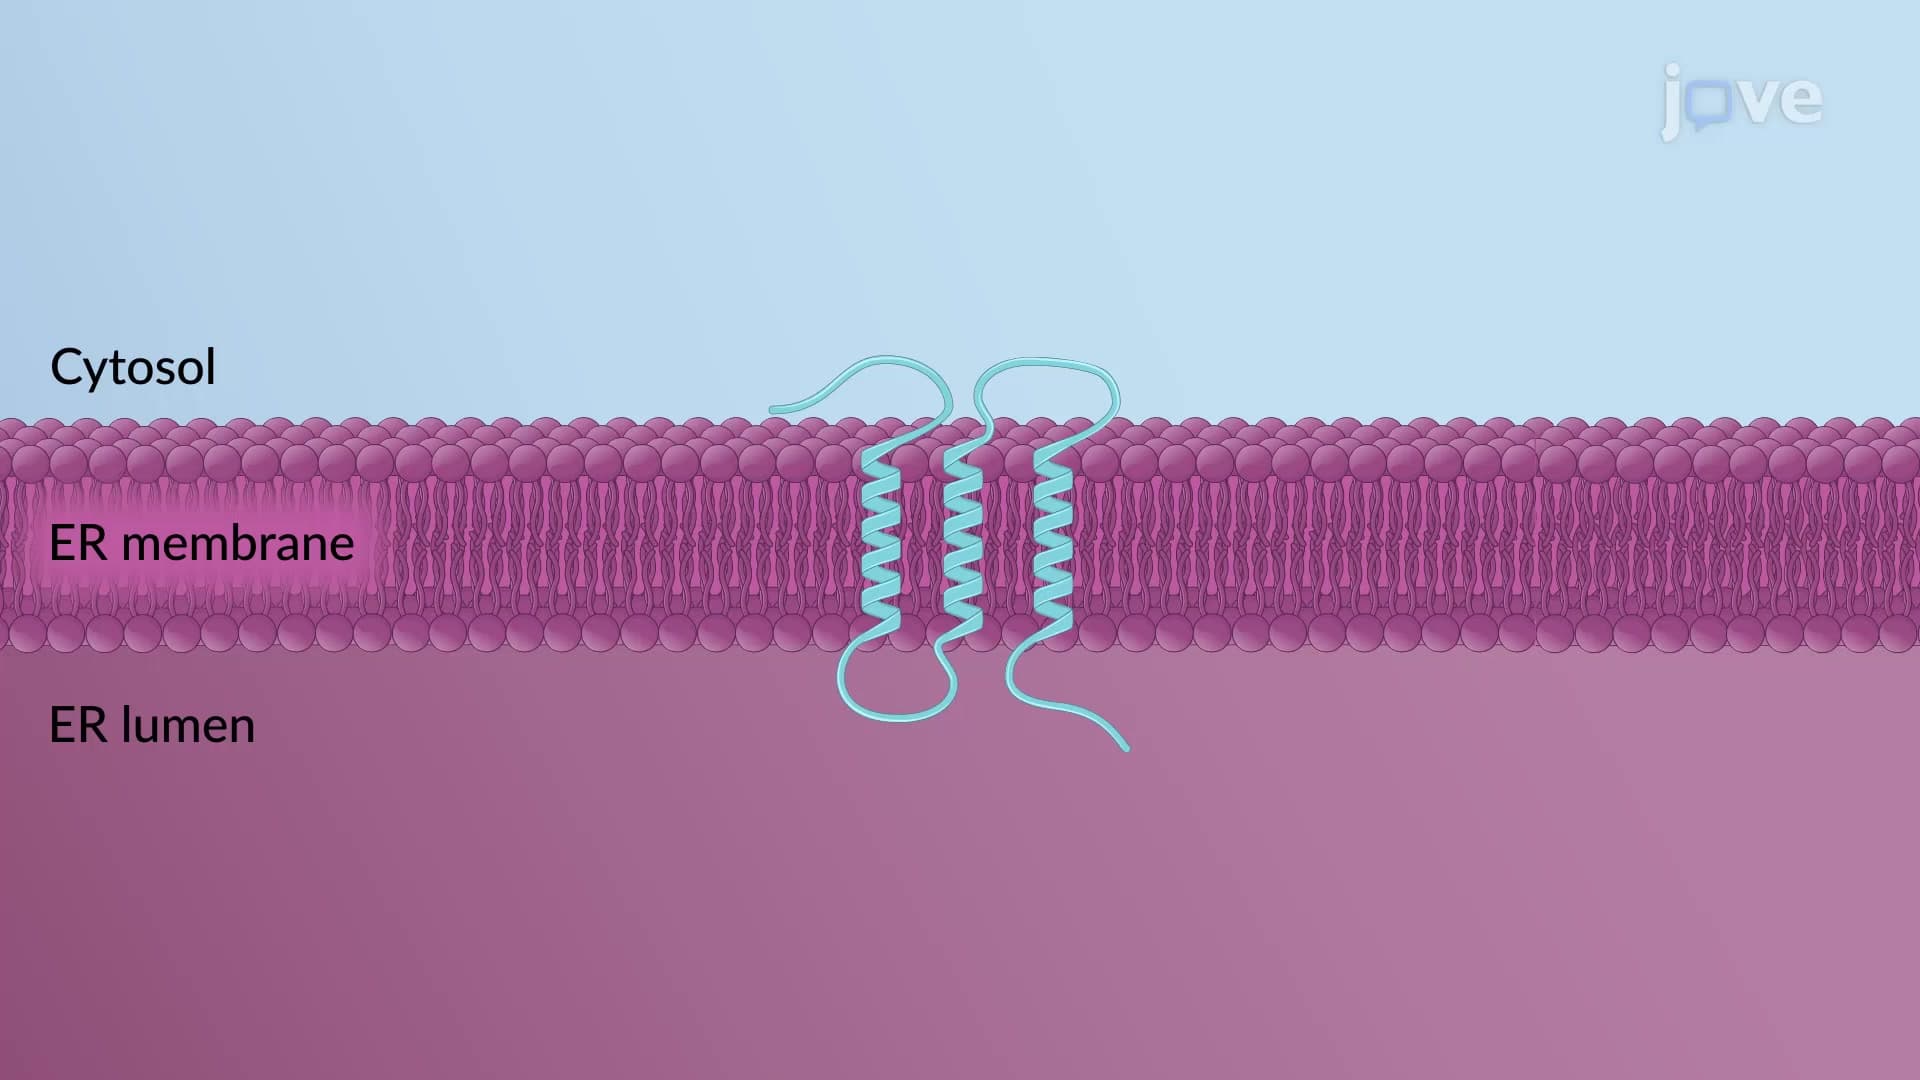
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
 01:19
Membrane Asymmetry Regulating Transporters
Flippase
Eukaryotic flippases are type-IV P-type ATPases or P4-ATPases belonging to P-type ATPase family proteins that are membrane-bound pumps involved in the ATP-mediated transport of ions and molecules across the membrane. Flippases flip specific phospholipids from the outer to the inner leaflet of a membrane. All P4-ATPases have one...