Related Experiment Video
Updated: Jul 6, 2026
A Direct Force Probe for Measuring Mechanical Integration Between the Nucleus and the Cytoskeleton
Published on: July 29, 2018
Synaptotagmin modulation of fusion pore kinetics in regulated exocytosis of dense-core vesicles
C T Wang1, R Grishanin, C A Earles
1Department of Physiology, University of Wisconsin Medical School, University of Wisconsin, Madison, WI 53706, USA.

Abstract:
In the exocytosis of neurotransmitter, fusion pore opening represents the first instant of fluid contact between the vesicle lumen and extracellular space. The existence of the fusion pore has been established by electrical measurements, but its molecular composition is unknown. The possibility that synaptotagmin regulates fusion pores was investigated with amperometry to monitor exocytosis of single dense-core vesicles. Overexpression of synaptotagmin I prolonged the time from fusion pore opening to dilation, whereas synaptotagmin IV shortened this time. Both synaptotagmin isoforms reduced norepinephrine flux through open fusion pores. Thus, synaptotagmin interacts with fusion pores, possibly by associating with a core complex of membrane proteins and/or lipid.
Related Concept Videos
 01:15
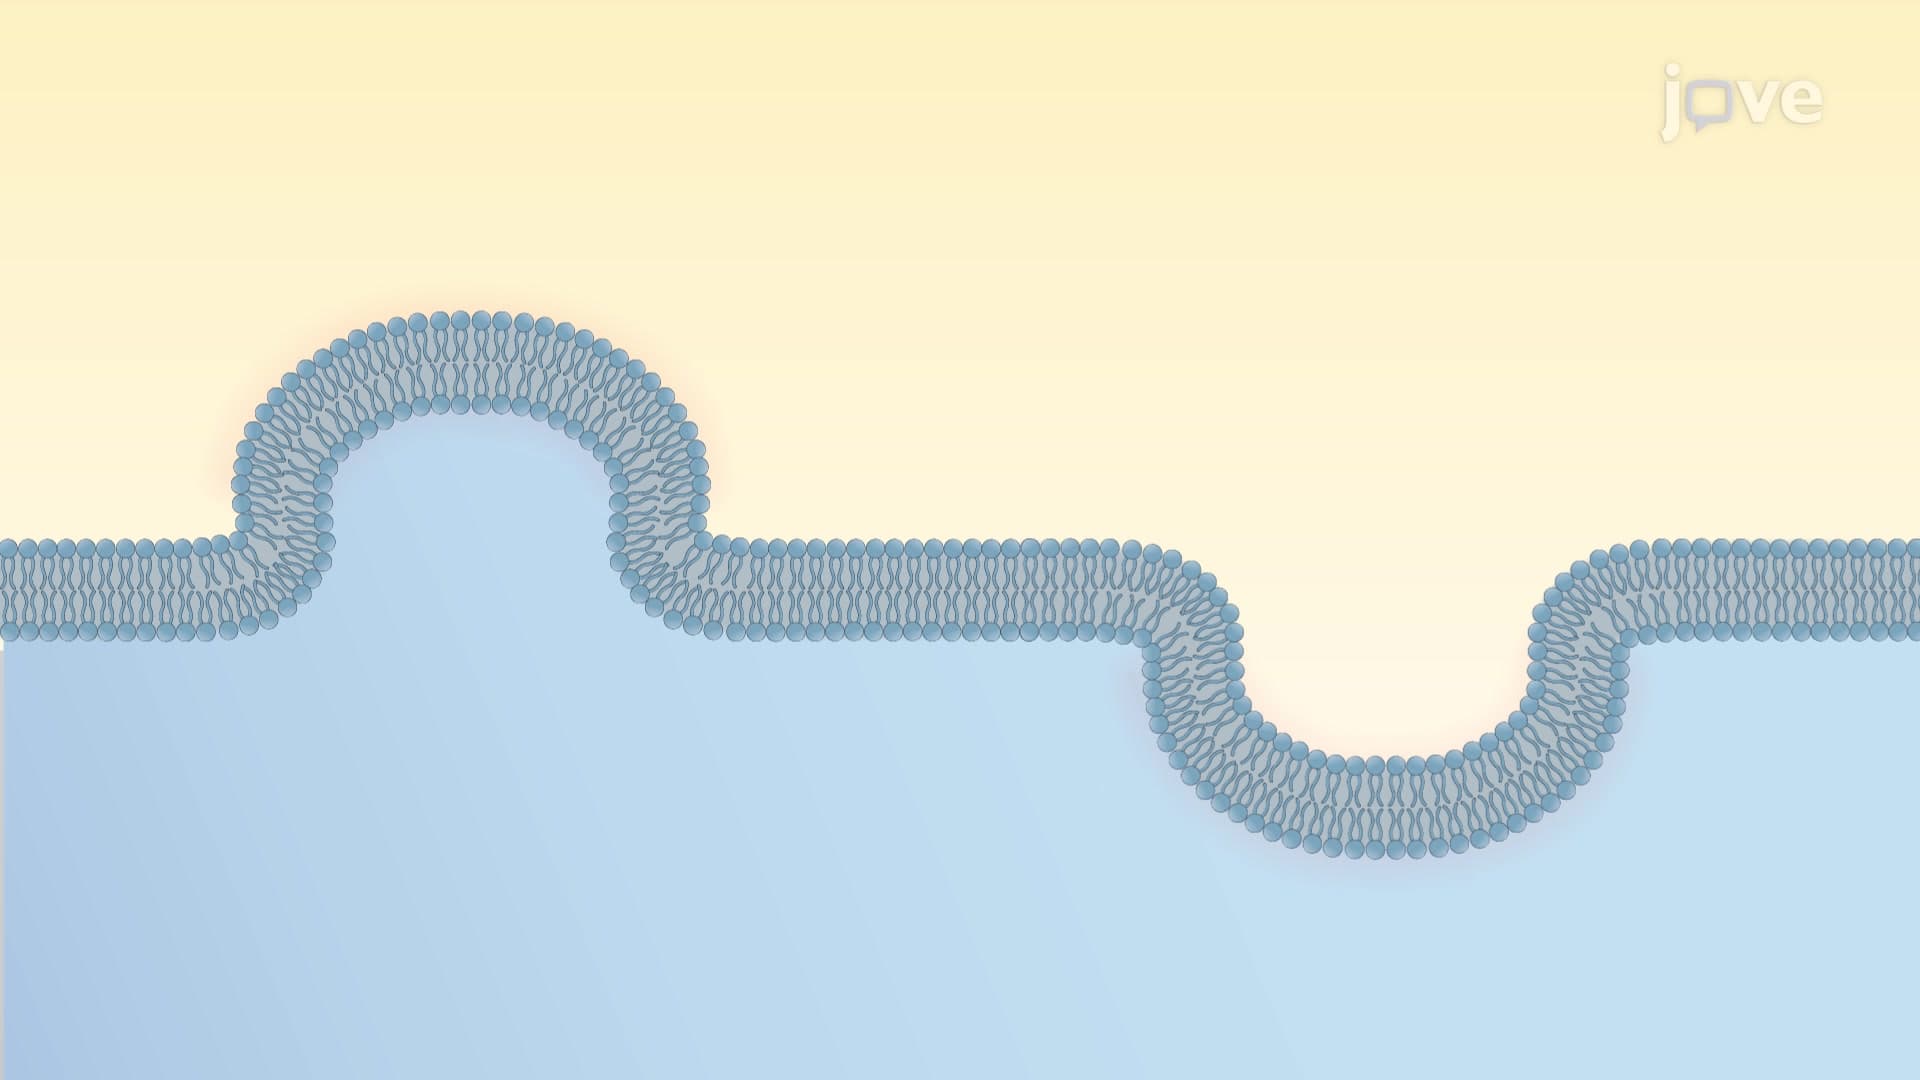
Mechanisms of Membrane-bending
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
 01:12
Adaptability of Cytoskeletal Filaments
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 02:17
Microtubule Instability
 01:13
Cell-matrix's Response to Mechanical Forces
Anchoring junctions mechanically attach a cell to the...