A brain-specific isoform of small glutamine-rich tetratricopeptide repeat-containing protein binds to Hsc70 and the
Sönke Tobaben1, Frederique Varoqueaux, Nils Brose
1Max Planck Institute for Experimental Medicine, Department of Molecular Neurobiology and Deutsche Forschungsgemeinschaft Center for Molecular Physiology of the Brain, Hermann-Rein-Strasse 3, D-37075 Göttingen, Germany.

Abstract:
Small glutamine-rich tetratricopeptide repeat-containing protein (SGT) is a ubiquitously expressed cochaperone of heat shock cognate protein of 70 kDa (Hsc70). SGT binds to the C terminus of Hsc70, a site used by several tetratricopeptide repeat-containing binding partners to recruit Hsc70 into complexes of diverse function. We describe here an isoform of SGT with 60% amino acid sequence identity that we name betaSGT. In contrast to the previously published alphaSGT, betaSGT is almost exclusively expressed in brain. Both isoforms of SGT possess similar binding properties toward Hsc70 and cysteine string protein, a synaptic vesicle-associated J-domain-containing protein. In addition, SGTs oligomerize without preferences among isoforms. The distribution of protein binding motifs on SGTs reveals a modular structure. The N-terminal domains mediate oligomerization. Binding to Hsc70 is impaired by mutations of basic residues within the central tetratricopeptide repeat domain of betaSGT, indicating a two-carboxylate clamp as the binding mode. The tetratricopeptide repeats are also necessary for binding to the cysteine string protein. However, this binding mode is distinct from the two-carboxylate clamp that is involved in Hsc70 binding. The C-terminal regions of SGTs might constitute independent protein interaction domains. We conclude that betaSGT is likely to cooperate with alphaSGT as co-chaperone of Hsc70 in the brain. The modular structure of SGTs allows them to recruit client proteins to Hsc70 and to direct the resulting complex toward downstream proteins that take over the respective client proteins.
Related Concept Videos
 02:41
Protein Complex Assembly
Many viruses self-assemble into a fully functional unit using the infected host cell to...
 01:45
Regulation of Nuclear Protein Sorting
 01:19
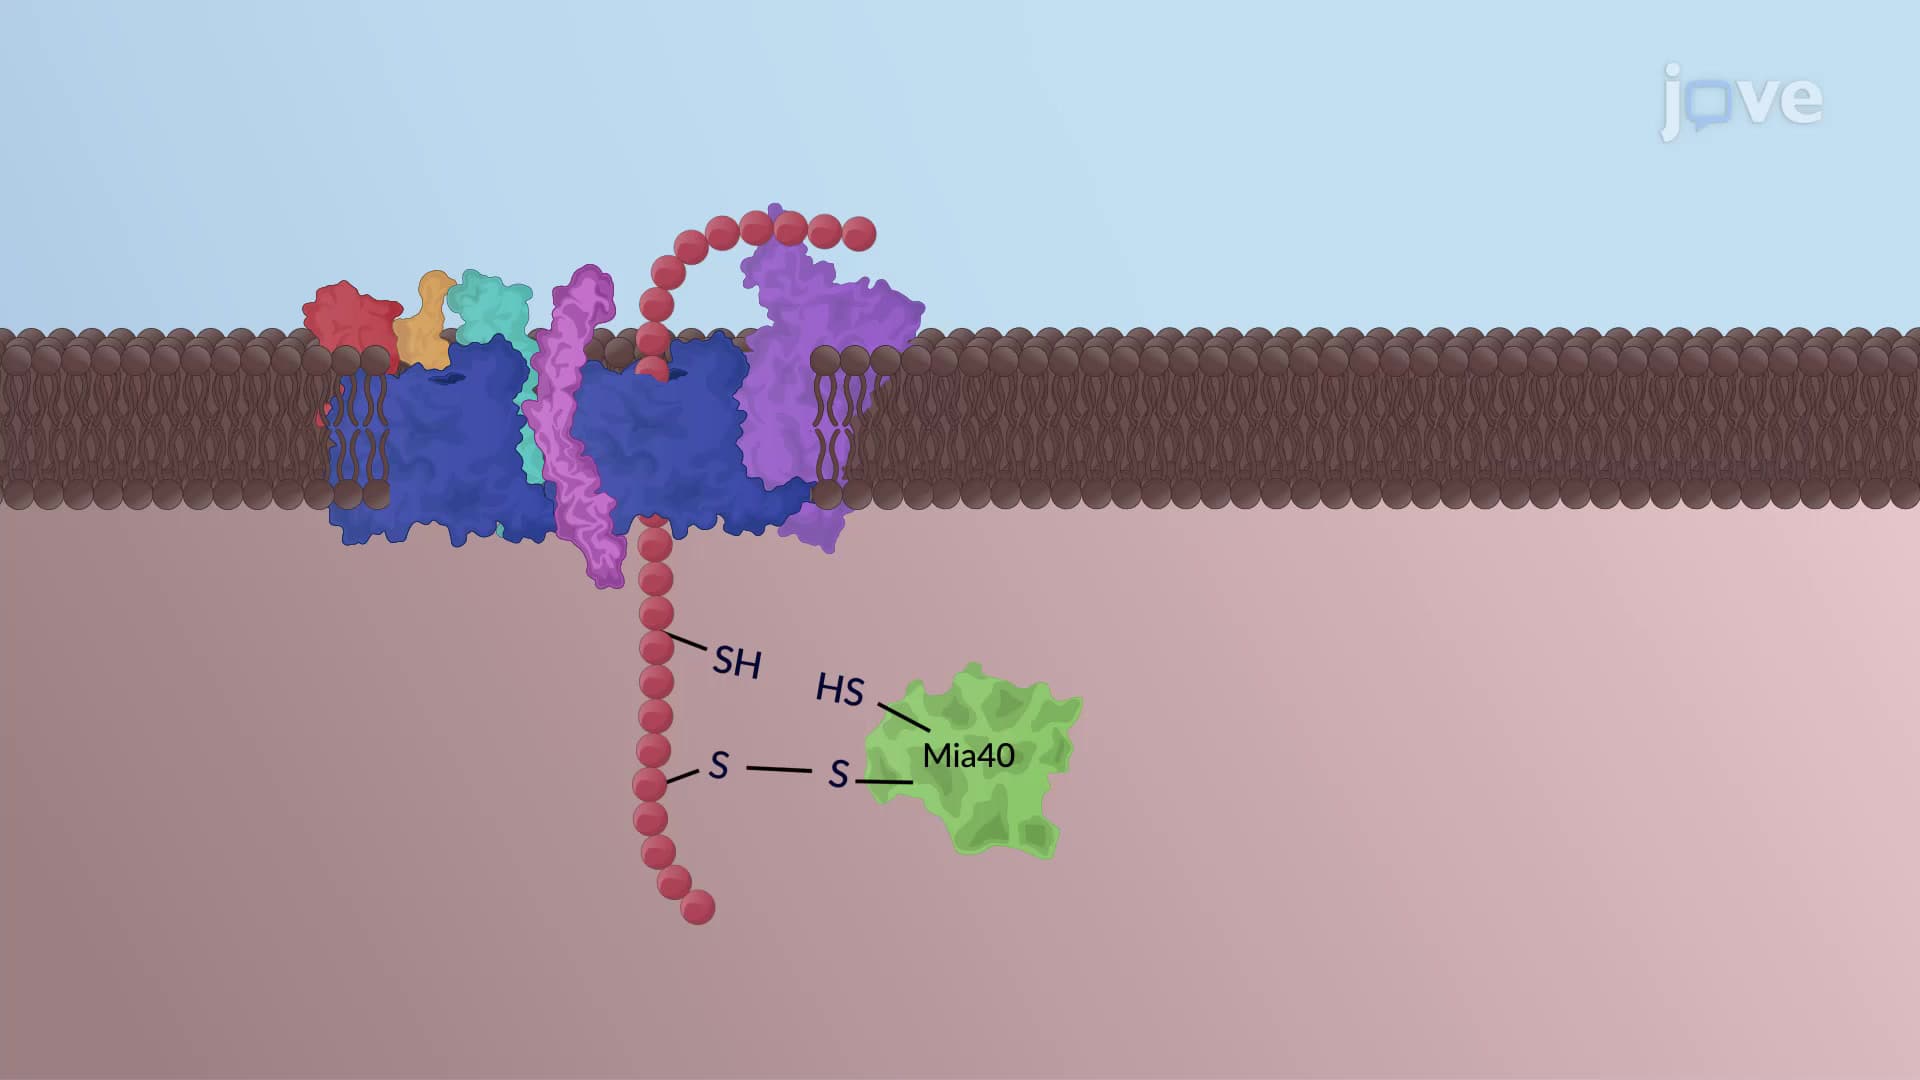
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:37
Energy to Drive Translocation
Generally, polypeptides are unfolded by two distinct...
 01:45
Vesicular Tubular Clusters
With the help of motor proteins such...
 01:29
Protein Folding Quality Check in the RER