Volatile anesthetics bind rat synaptic snare proteins
Related Experiment Video
Updated: Aug 15, 2026
Optogenetic Activation of Afferent Pathways in Brain Slices and Modulation of Responses by Volatile Anesthetics
Published on: July 23, 2020
Peter Nagele1, J Brett Mendel, William J Placzek
1Department of Anesthesiology, Washington University School of Medicine, St. Louis, MO 63110, USA.

Background:
Volatile general anesthetics (VAs) have a number of synaptic actions, one of which is to inhibit excitatory neurotransmitter release; however, no presynaptic VA binding proteins have been identified. Genetic data in Caenorhabditis elegans have led to the hypothesis that a protein that interacts with the presynaptic protein syntaxin 1A is a VA target. Motivated by this hypothesis, the authors measured the ability of syntaxin 1A and proteins that interact with syntaxin to bind to halothane and isoflurane.
Methods:
Recombinant rat syntaxin 1A, SNAP-25B, VAMP2, and the ternary SNARE complex that they form were tested. Binding of VAs to these proteins was detected by F-nuclear magnetic resonance relaxation measurements. Structural alterations in the proteins were examined by circular dichroism and ability to form complexes.
Results:
Volatile anesthetics did not bind to VAMP2. At concentrations in the clinical range, VAs did bind to SNAP-25B; however, binding was detected only in preparations containing SNAP-25B homomultimers. VAs also bound at clinical concentrations to both syntaxin and the SNARE complex. Addition of an N-terminal His6 tag to syntaxin abolished its ability to bind VAs despite normal secondary structure and ability to form SNARE complexes; thrombin cleavage of the tag restored VA binding. Thus, the VA binding site(s) has structural requirements and is not simply any alpha-helical bundle. VAs at supraclinical concentrations produced an increase in helicity of the SNARE complex; otherwise, VA binding produced no gross alteration in the stability or secondary structure of the SNARE complex.
Conclusion:
SNARE proteins are potential synaptic targets of volatile anesthetics.
More Related Videos
 08:49
Assessing Changes in Volatile General Anesthetic Sensitivity of Mice after Local or Systemic Pharmacological Intervention
Published on: October 16, 2013
 08:38
Vibrodissociation of Neurons from Rodent Brain Slices to Study Synaptic Transmission and Image Presynaptic Terminals
Published on: May 25, 2011
Related Concept Videos
 01:28
Depolarizing Blockers: Mechanism of Action
Succinylcholine is the most commonly used depolarizing blocker. Chemically, it constitutes two molecules of acetylcholine joined together by an acetate methyl group. They act on the receptors in the same way as acetylcholine. Because succinylcholine...
 01:26
Chemical Synapses
Because chemical synapses depend on the release of neurotransmitter molecules from synaptic vesicles to pass on their signal, there is an approximately one millisecond delay between when the axon potential reaches the presynaptic terminal and when the neurotransmitter leads to opening of postsynaptic ion channels. Additionally, this signaling is...
01:26Chemical Synapses
Because chemical synapses depend on the release of neurotransmitter molecules from synaptic vesicles to pass on their signal, there is an approximately one millisecond delay between when the axon potential reaches the presynaptic terminal and when the neurotransmitter leads to opening of postsynaptic ion channels. Additionally, this signaling is...
 01:23
Local Anesthetics: Mechanism of Action
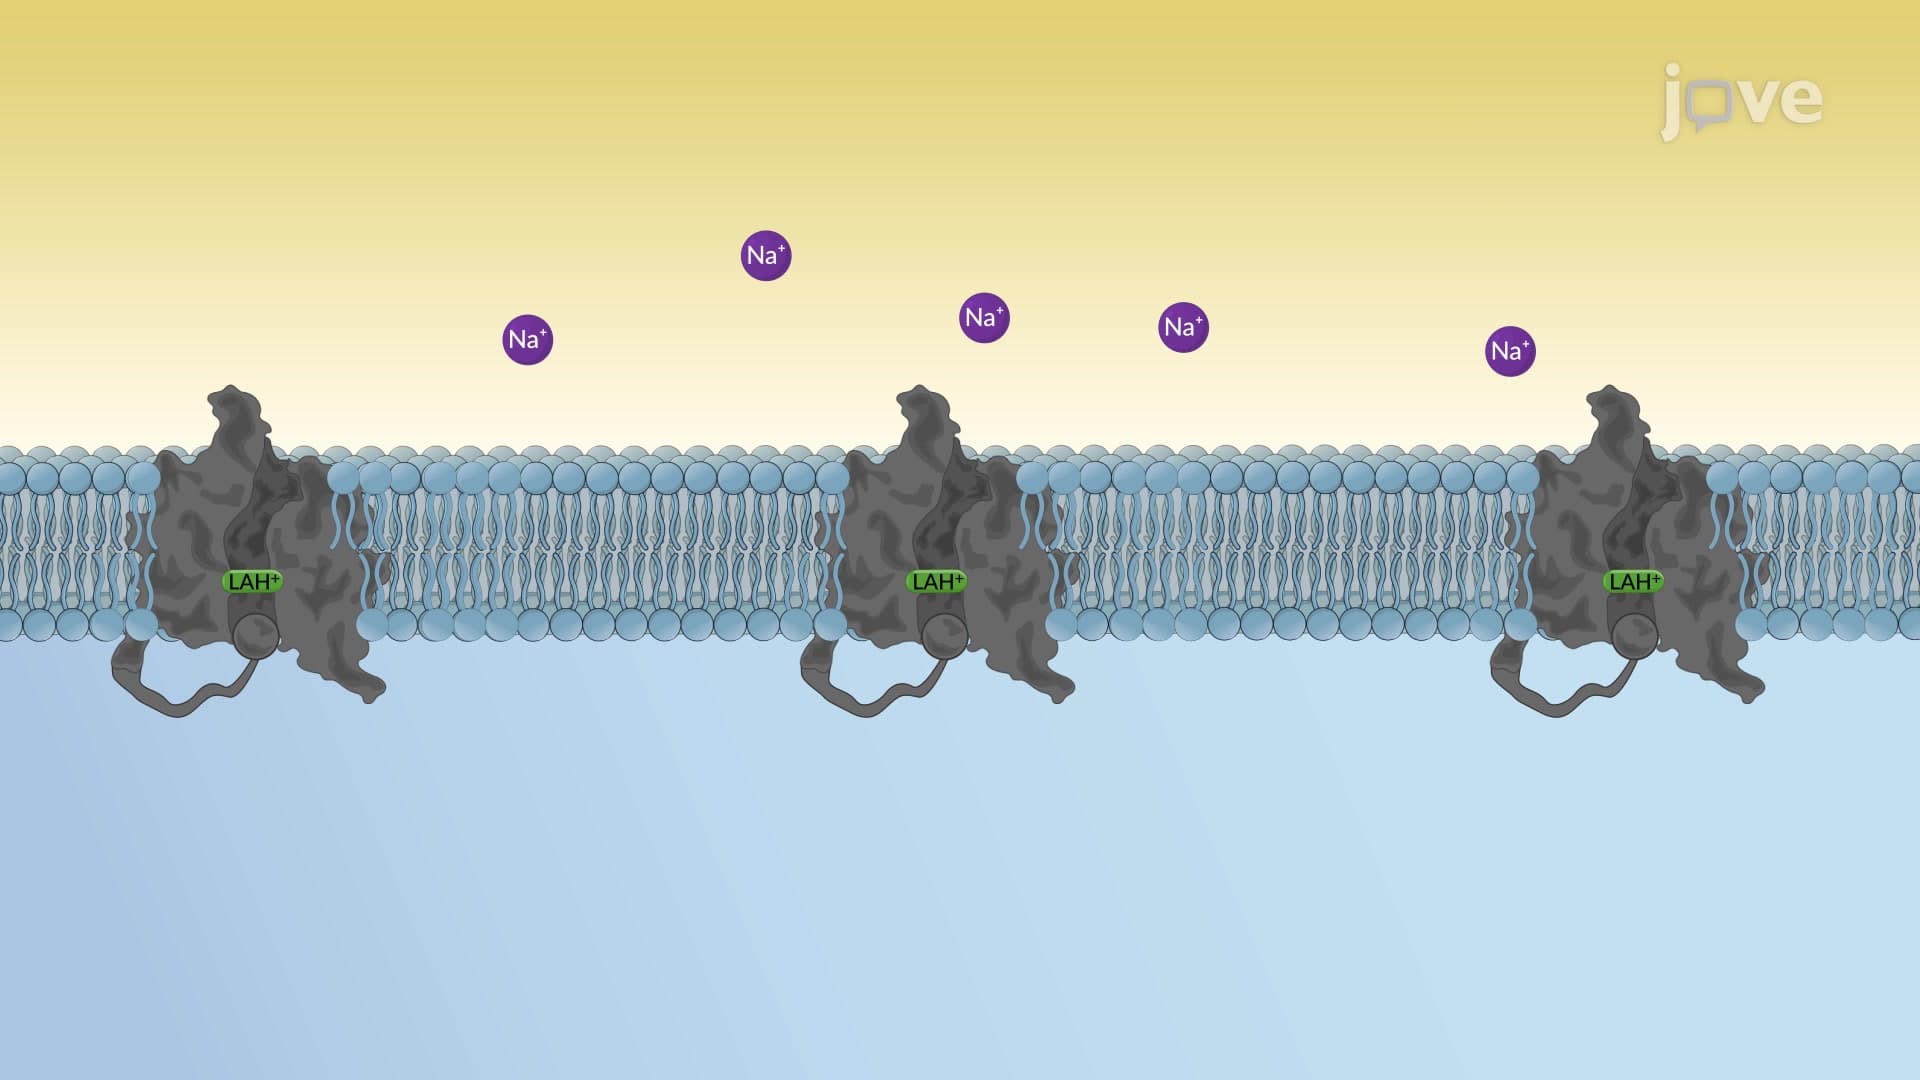
Local anesthetics are amphiphilic molecules consisting of a hydrophobic aromatic part linked to a hydrophilic group by an ester or amide linkage. They are weak bases and are usually available as salts, which increases their solubility and stability. Once administered, LAs exist in the body either...
 01:17
Nondepolarizing (Competitive) Neuromuscular Blockers: Mechanism of Action
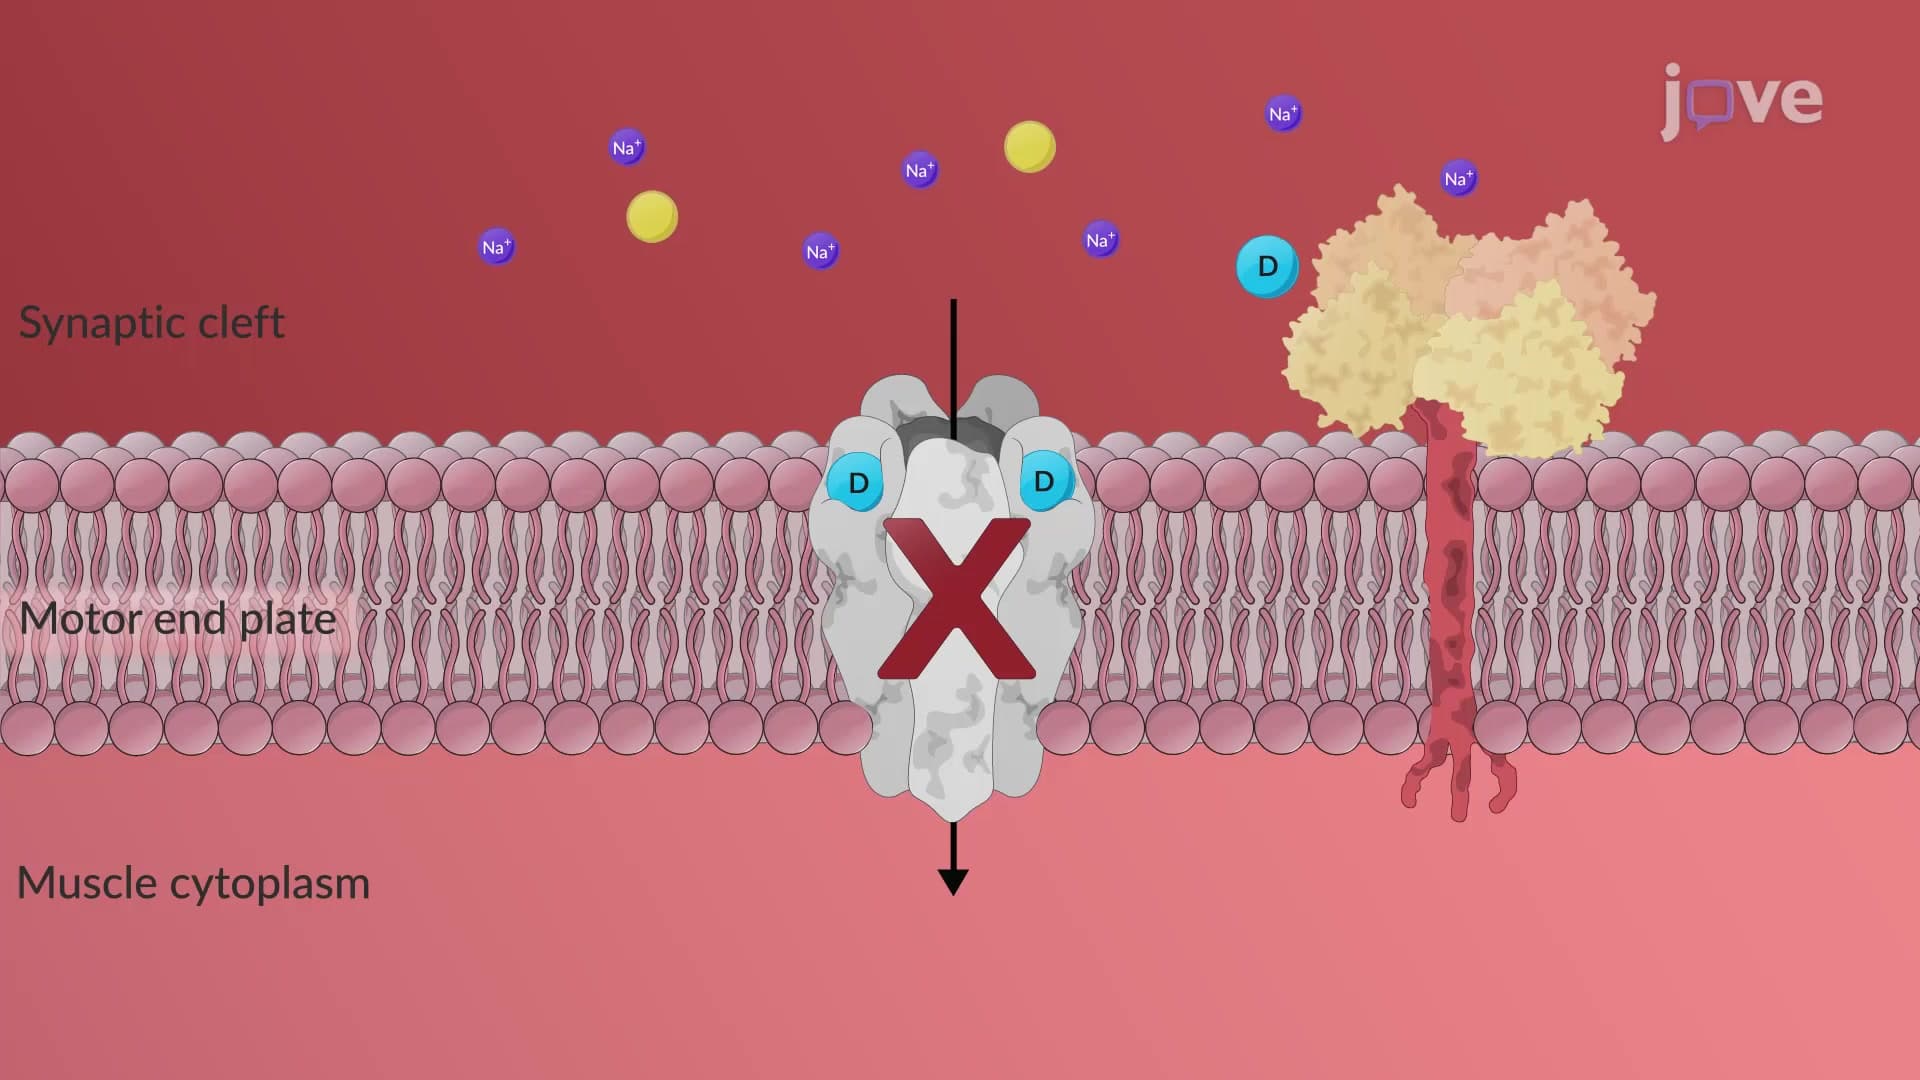
Competitive antagonists prevent acetylcholine from binding to its receptor, inhibiting membrane depolarization. Without conformational changes or intrinsic...
 01:30
Local Anesthetics: Chemistry and Structure-Activity Relationship