Related Experiment Video
Updated: Aug 8, 2026

Light-driven Enzymatic Decarboxylation
Published on: May 22, 2016
Transport of dicarboxylic acids in castor bean mitochondria
1Biology Department, University of California, Santa Cruz, California 95064.

Abstract:
Mitochondria from castor bean (Ricinus communis cv Hale) endosperm, purified on sucrose gradients, were used to investigate transport of dicarboxylic acids. The isolated mitochondria oxidized malate and succinate with respiratory control ratios greater than 2 and ADP/O ratios of 2.6 and 1.7, respectively. Net accumulation of (14)C from [(14)C]malate or [(14)C]succinate into the mitochondrial matrix during substrate oxidation was examined by the silicone oil centrifugation technique. In the presence of ATP, there was an appreciable increase in the accumulation of (14)C from [(14)C]malate or [(14)C]succinate accompanied by an increased oxidation rate of the respective dicarboxylate. The net accumulation of dicarboxylate in the presence of ATP was saturable with apparent K(m) values of 2 to 2.5 millimolar. The ATP-stimulated accumulation of dicarboxylate was unaffected by oligomycin but inhibited by uncouplers (2,4-dinitrophenol and carbonyl cyanide m-chlorophenylhydrazone) and inhibitors of the electron transport chain (antimycin A, KCN). Dicarboxylate accumulation was also inhibited by butylmalonate, benzylmalonate, phenylsuccinate, mersalyl and N-ethylmaleimide. The optimal ATP concentration for stimulation of dicarboxylate accumulation was 1 millimolar. CTP was as effective as ATP in stimulating dicarboxylate accumulation, and other nucleotide triphosphates showed intermediate or no effect on dicarboxylate accumulation. Dicarboxylate accumulation was phosphate dependent but, inasmuch as ATP did not increase phosphate uptake, the ATP stimulation of dicarboxylate accumulation was apparently not due to increased availability of exchangeable phosphate.The maximum rate of succinate accumulation (14.5 nanomoles per minute per milligram protein) was only a fraction of the measured rate of oxidation (100-200 nanomoles per minute per milligram protein). Efflux of malate from the mitochondria was shown to occur at high rates (150 nanomoles per minute per milligram protein) when succinate was provided, suggesting dicarboxylate exchange. The uptake of [(14)C]succinate into malate or malonate preloaded mitochondria was therefore determined. In the absence of phosphate, uptake of [(14)C]succinate into mitochondria preloaded with malate was rapid (27 nanomoles per 15 seconds per milligram protein at 4 degrees C) and inhibited by butylmalonate, benzylmalonate, and phenylsuccinate. Uptake of [(14)C]succinate into mitochondria preloaded with malonate showed saturation kinetics with an apparent K(m) of 2.5 millimolar and V(max) of 250 nanomoles per minute per milligram protein at 4 degrees C. The measured rates of dicarboxylate-dicarboxylate exchange in castor bean mitochondria are sufficient to account for the observed rates of substrate oxidation.
Related Concept Videos
 01:35
Loss of Carboxy Group as CO2: Decarboxylation of Malonic Acid Derivatives
 01:28
Overview of Fatty Acid Metabolism
Fatty acids are catabolized in a process called beta-oxidation, which takes place in the matrix of the mitochondria and converts their fatty acid chains into two-carbon units of acetyl groups. The acetyl...
 01:02
Loss of Carboxy Group as CO2: Decarboxylation of β-Ketoacids
 01:15
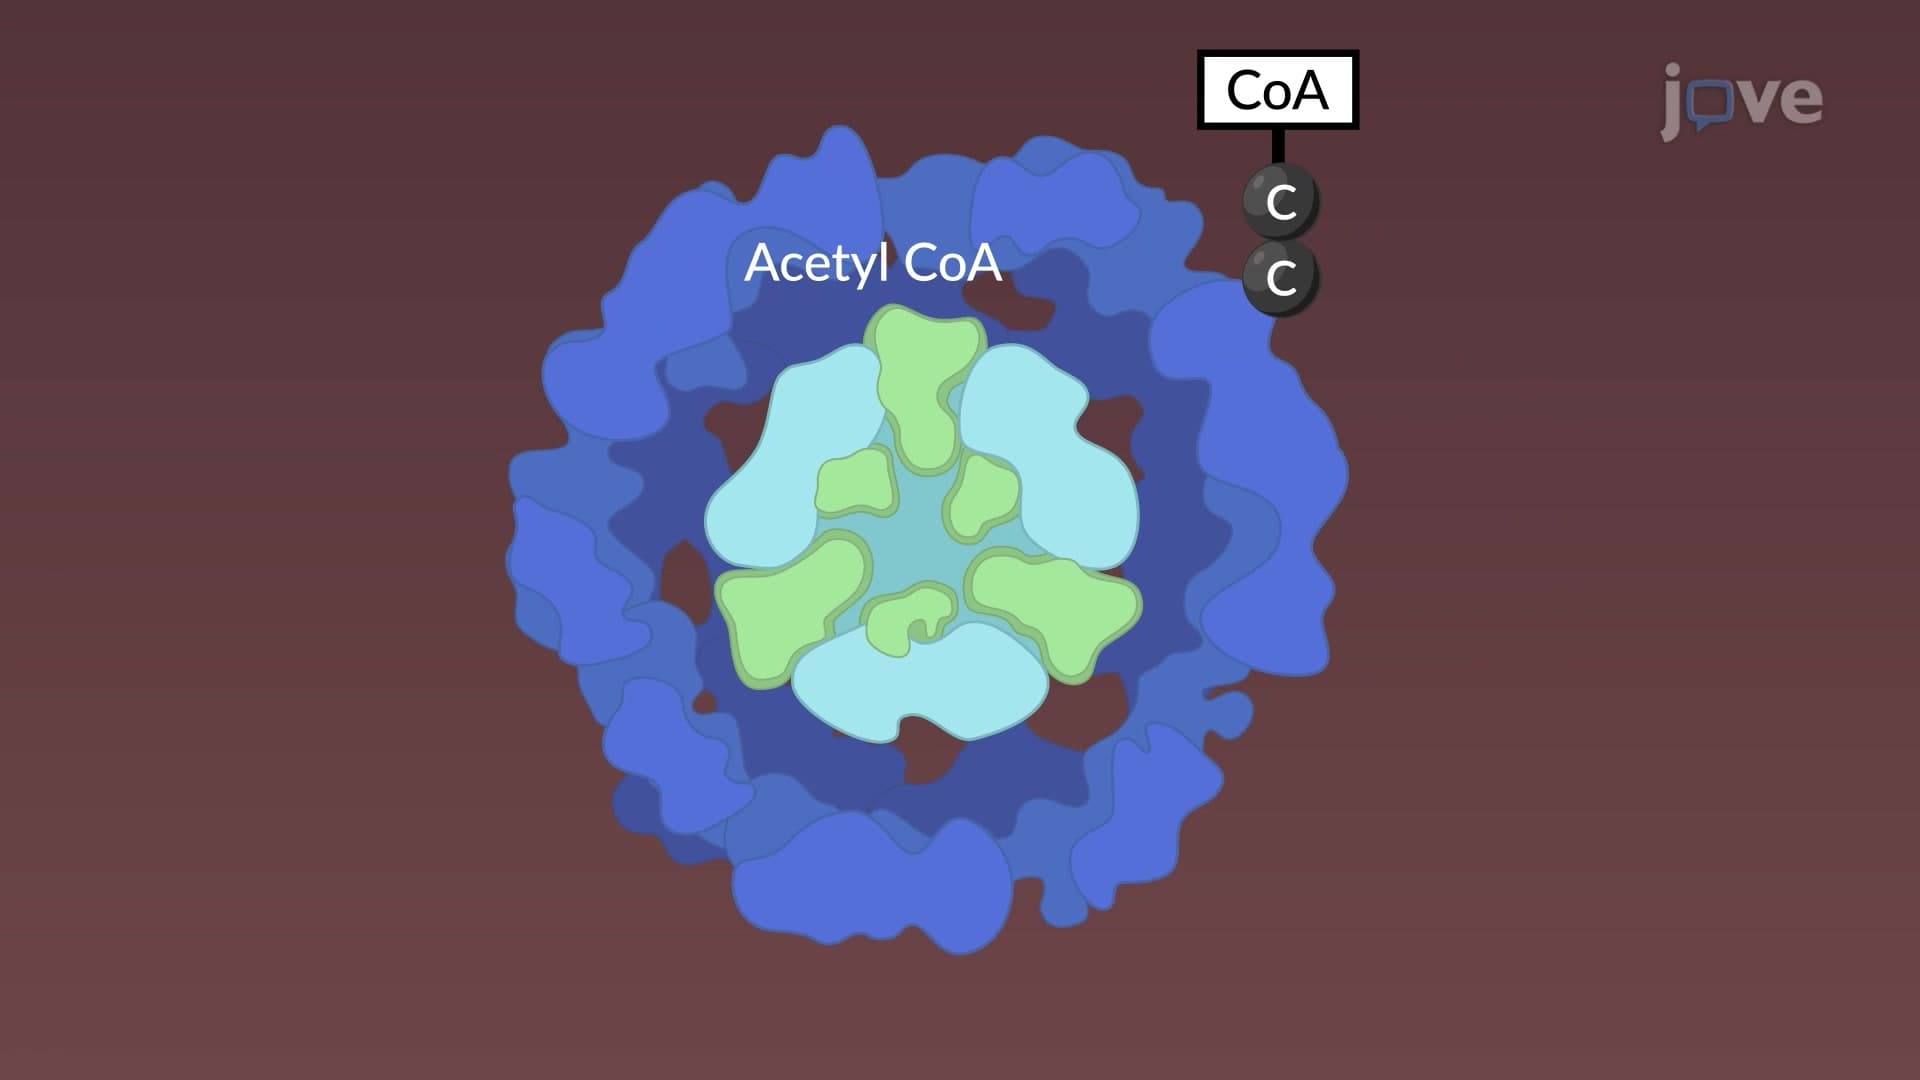
Pyruvate Oxidation
First, the enzyme pyruvate dehydrogenase removes the carboxyl group from pyruvate and releases it as carbon dioxide. The stripped molecule is then oxidized and releases electrons, which are then picked up by NAD+...
 01:16
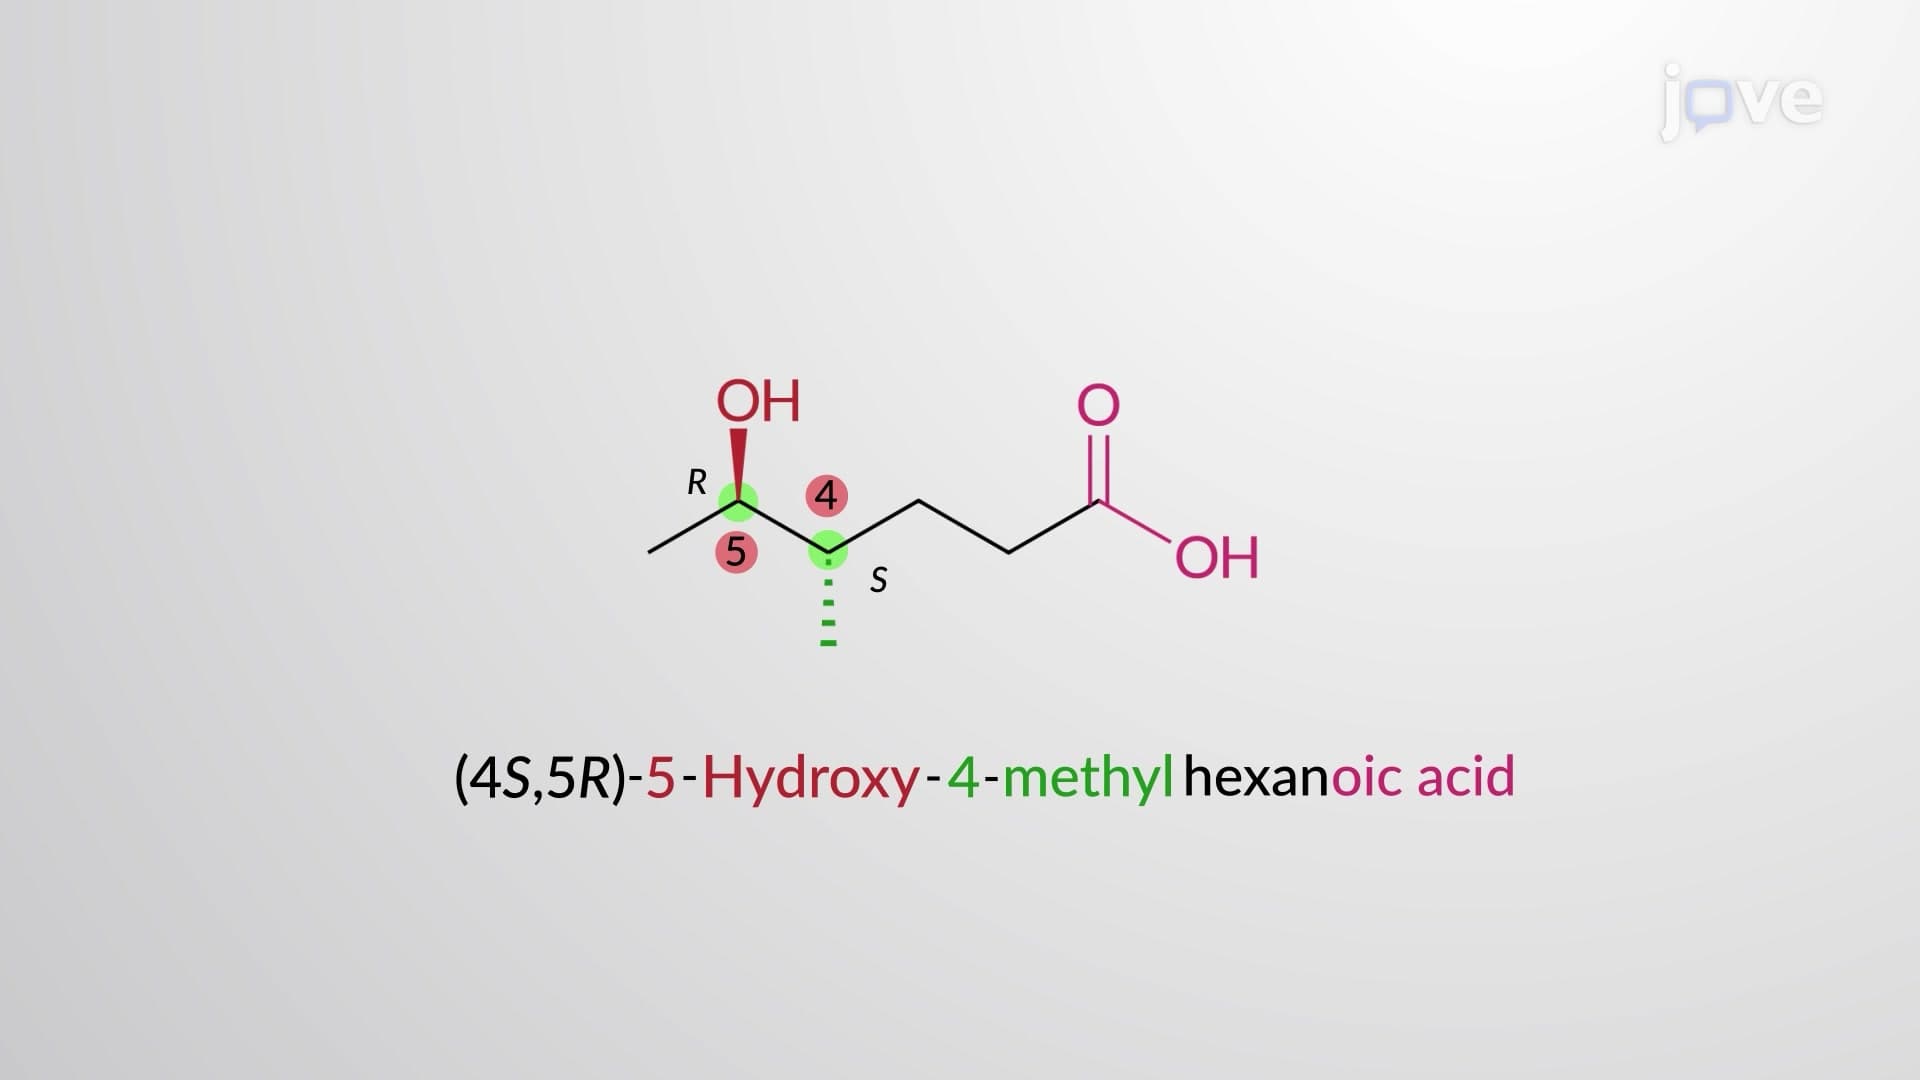
IUPAC Nomenclature of Carboxylic Acids
For acyclic saturated monocarboxylic acids, the longest hydrocarbon chain containing the –COOH carbon is identified as the parent chain. Then, the last -e of the parent hydrocarbon name is replaced with a suffix -oic acid.
 01:13
Carboxylic Acids to Esters: Acid-Catalyzed (Fischer) Esterification Mechanism