
The Brichos domain-containing C-terminal part of pro-surfactant protein C binds to an unfolded poly-val transmembrane
Hanna Johansson1, Kerstin Nordling1, Timothy E Weaver2
1Department of Molecular Biosciences, Swedish University of Agricultural Sciences, The Biomedical Centre, S-751 23 Uppsala, Sweden.

Abstract:
Native lung surfactant protein C (SP-C) is a 4.2-kDa acylpeptide that associates with alveolar surfactant phospholipids via a transmembrane alpha-helix. This helix contains mainly Val, although poly-Val is inefficient in helix formation, and helical SP-C can spontaneously convert to beta-sheet aggregates and amyloid-like fibrils. SP-C is cleaved out from a 21-kDa integral membrane protein, proSP-C, in the alveolar type II cell. Recently several mutations localized in the endoplasmic reticulum-lumenal (C-terminal) part of proSP-C (CTproSP-C) have been associated with intracellular accumulation of toxic forms of proSP-C, low levels of mature SP-C, and development of interstitial lung disease. CTproSP-C contains a approximately 100-residue Brichos domain of unknown function that is also found in other membrane proteins associated with amyloid formation, dementia, and cancer. Here we find that recombinant CTproSP-C binds lipid-associated SP-C, which is in beta-strand conformation, and that this interaction results in an increased helical content. In contrast, CTproSP-C does not bind alpha-helical SP-C. Recombinant CTproSP-C(L188Q), a mutation associated with interstitial lung disease, shows secondary and quaternary structures similar to those of wild type CTproSP-C but is unable to bind lipid-associated beta-strand SP-C. Transfection of CTproSP-C into HEK293 cells that express proSP-C(L188Q) increases the amount of proSP-C protein, whereas no effect is seen on cells expressing wild type proSP-C. These findings suggest that CTproSP-C binds nonhelical SP-C and thereby prevents beta-sheet aggregation and that mutations in CTproSP-C can interfere with this function.
More Related Videos
 09:49
Sedimentation Equilibrium of a Small Oligomer-forming Membrane Protein: Effect of Histidine Protonation on Pentameric Stability
Published on: April 2, 2015
 14:56
Expression and Purification of the Cystic Fibrosis Transmembrane Conductance Regulator Protein in Saccharomyces cerevisiae
Published on: March 10, 2012
Related Concept Videos
 01:26
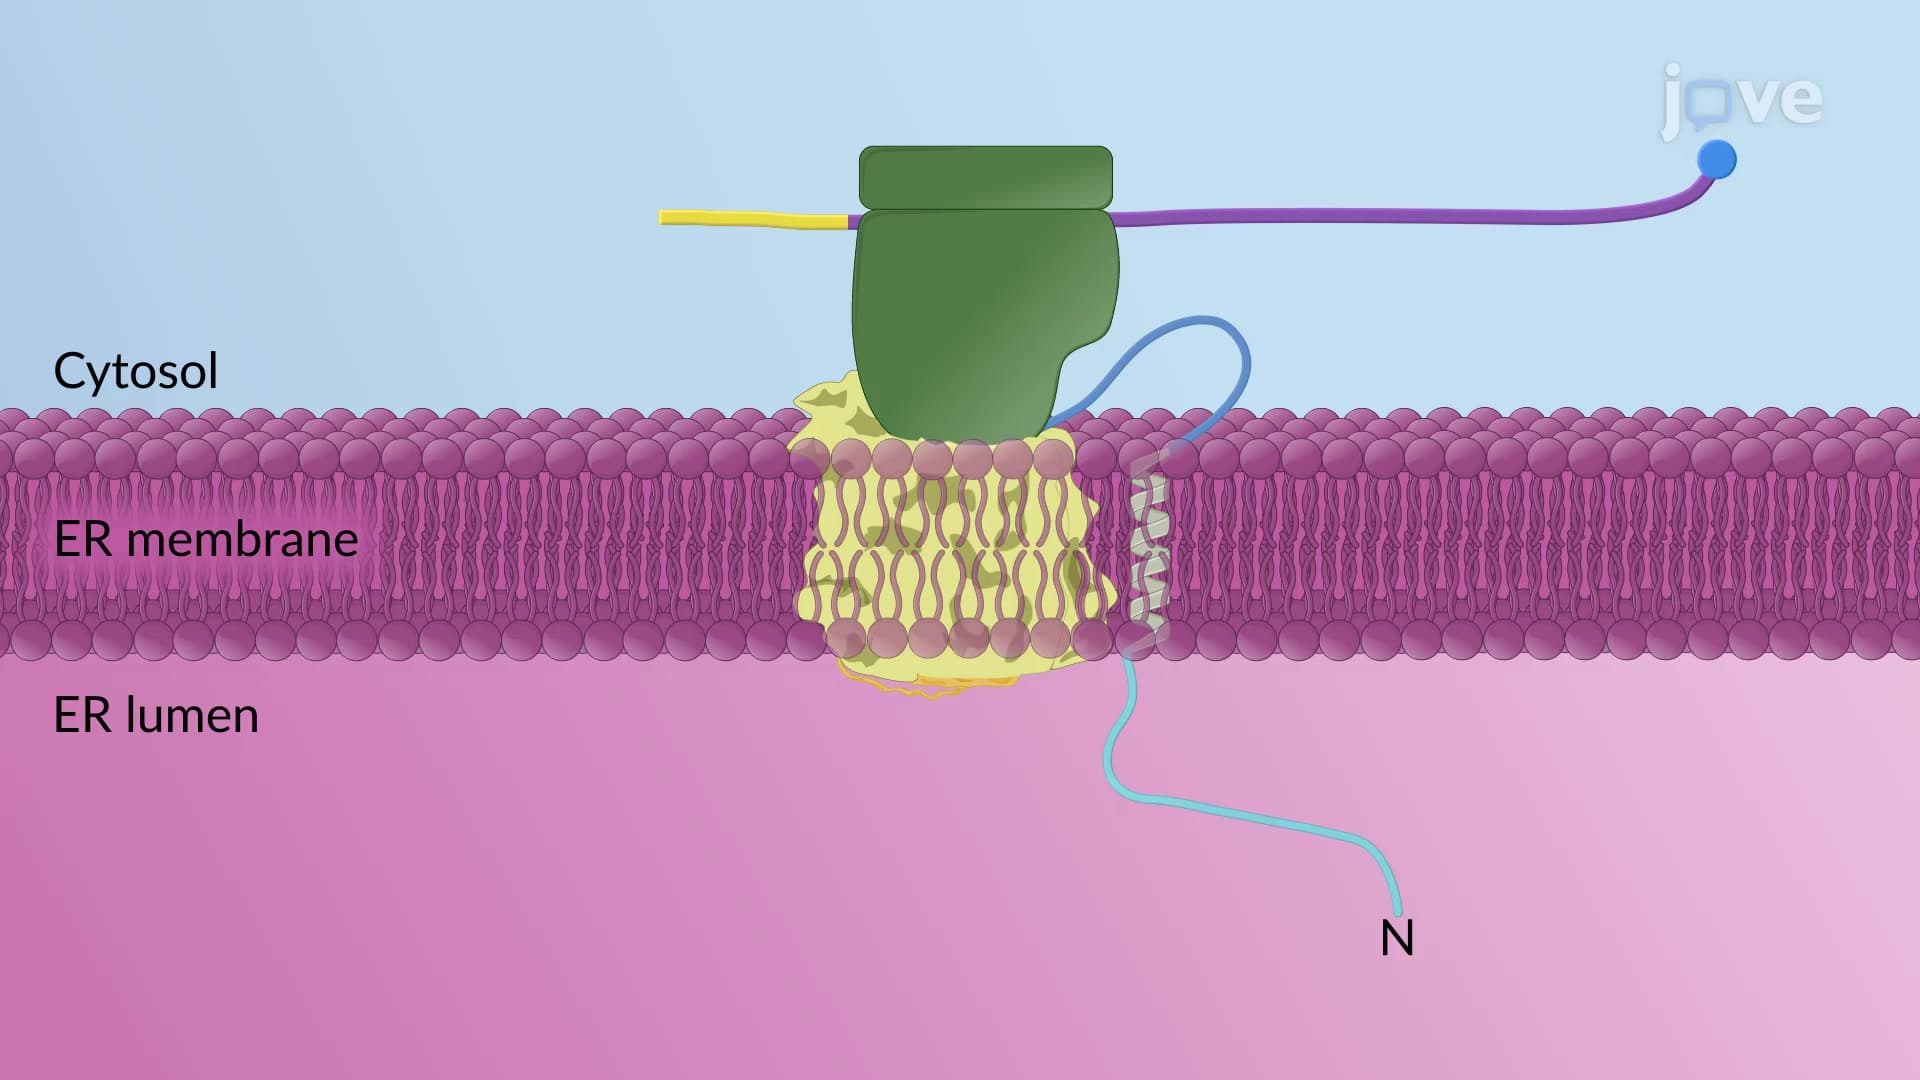
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 02:26
Conservation of Protein Domains Over Different Proteins
A limited set of protein domains often duplicate and recombine during evolution. These domains can be organized in different combinations to form...
 01:09
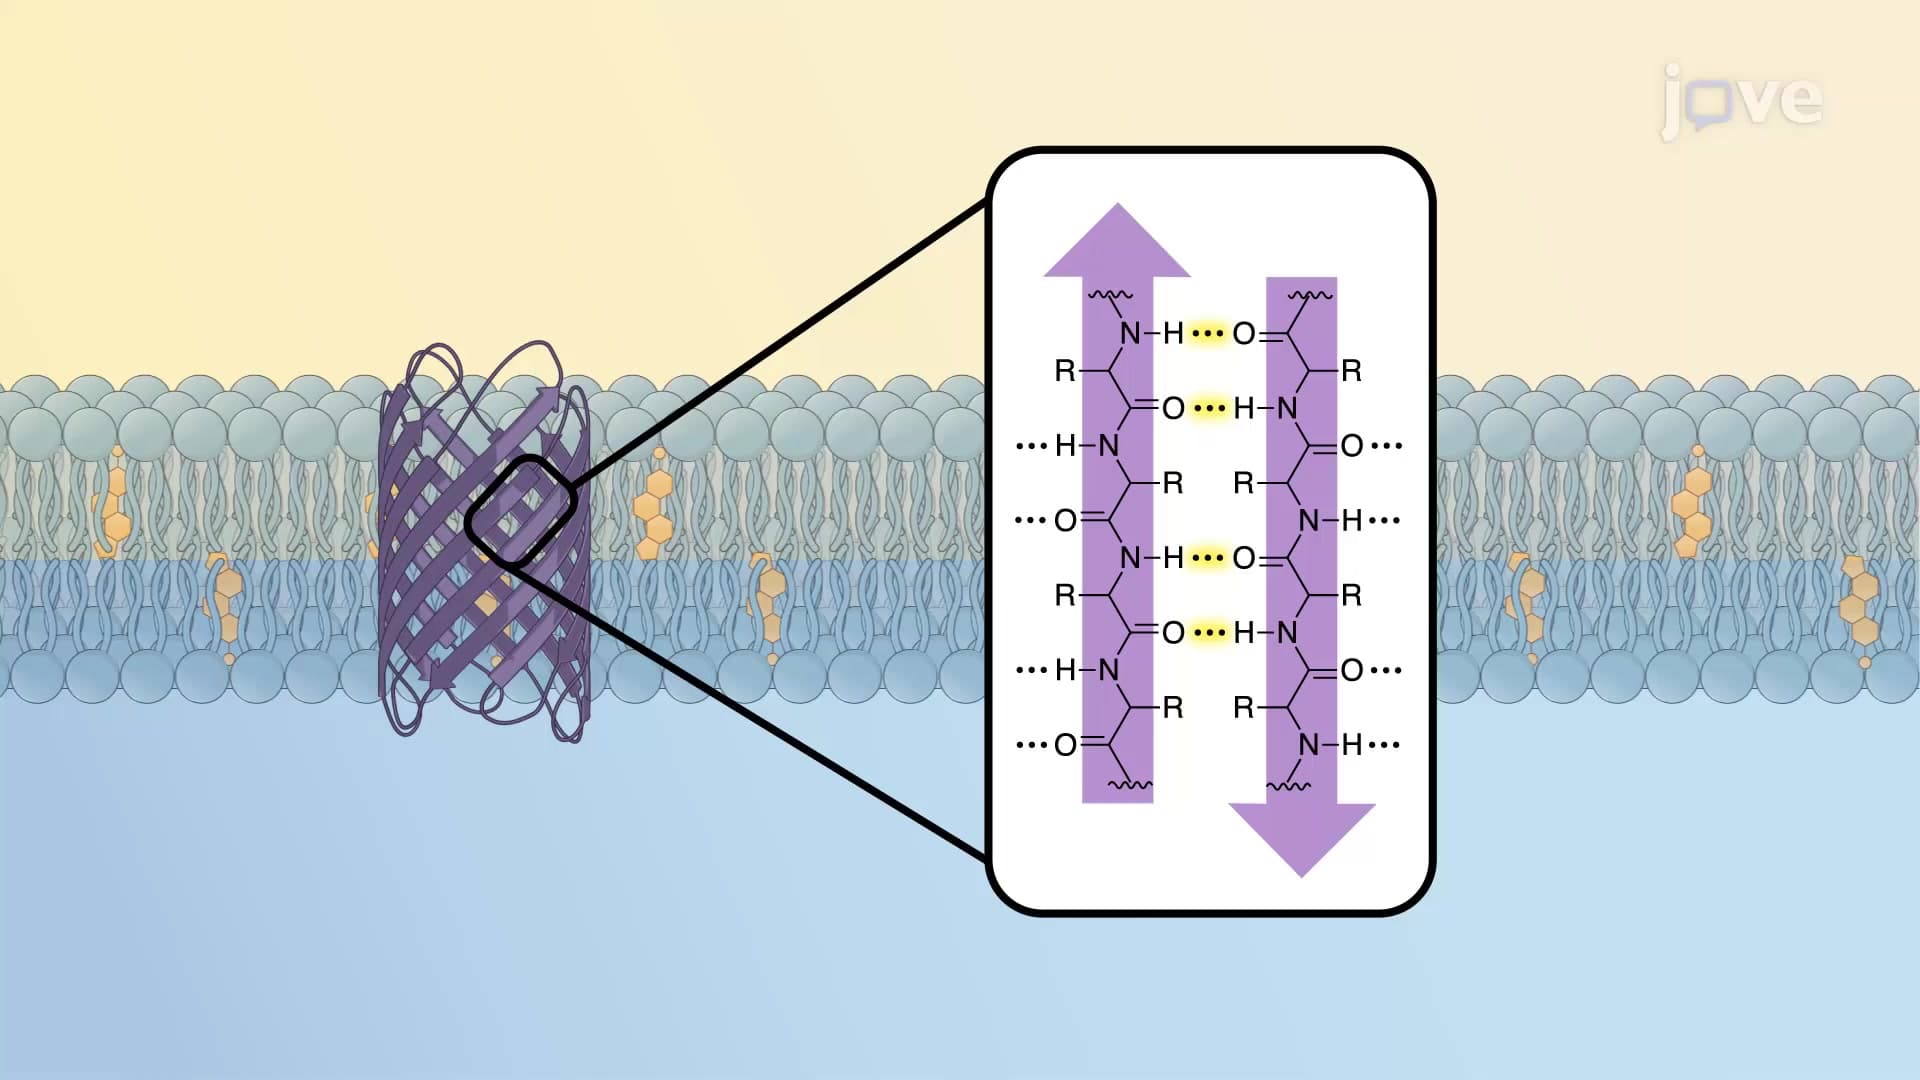
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as G-protein-linked receptors (GPCRs) and...
 01:29
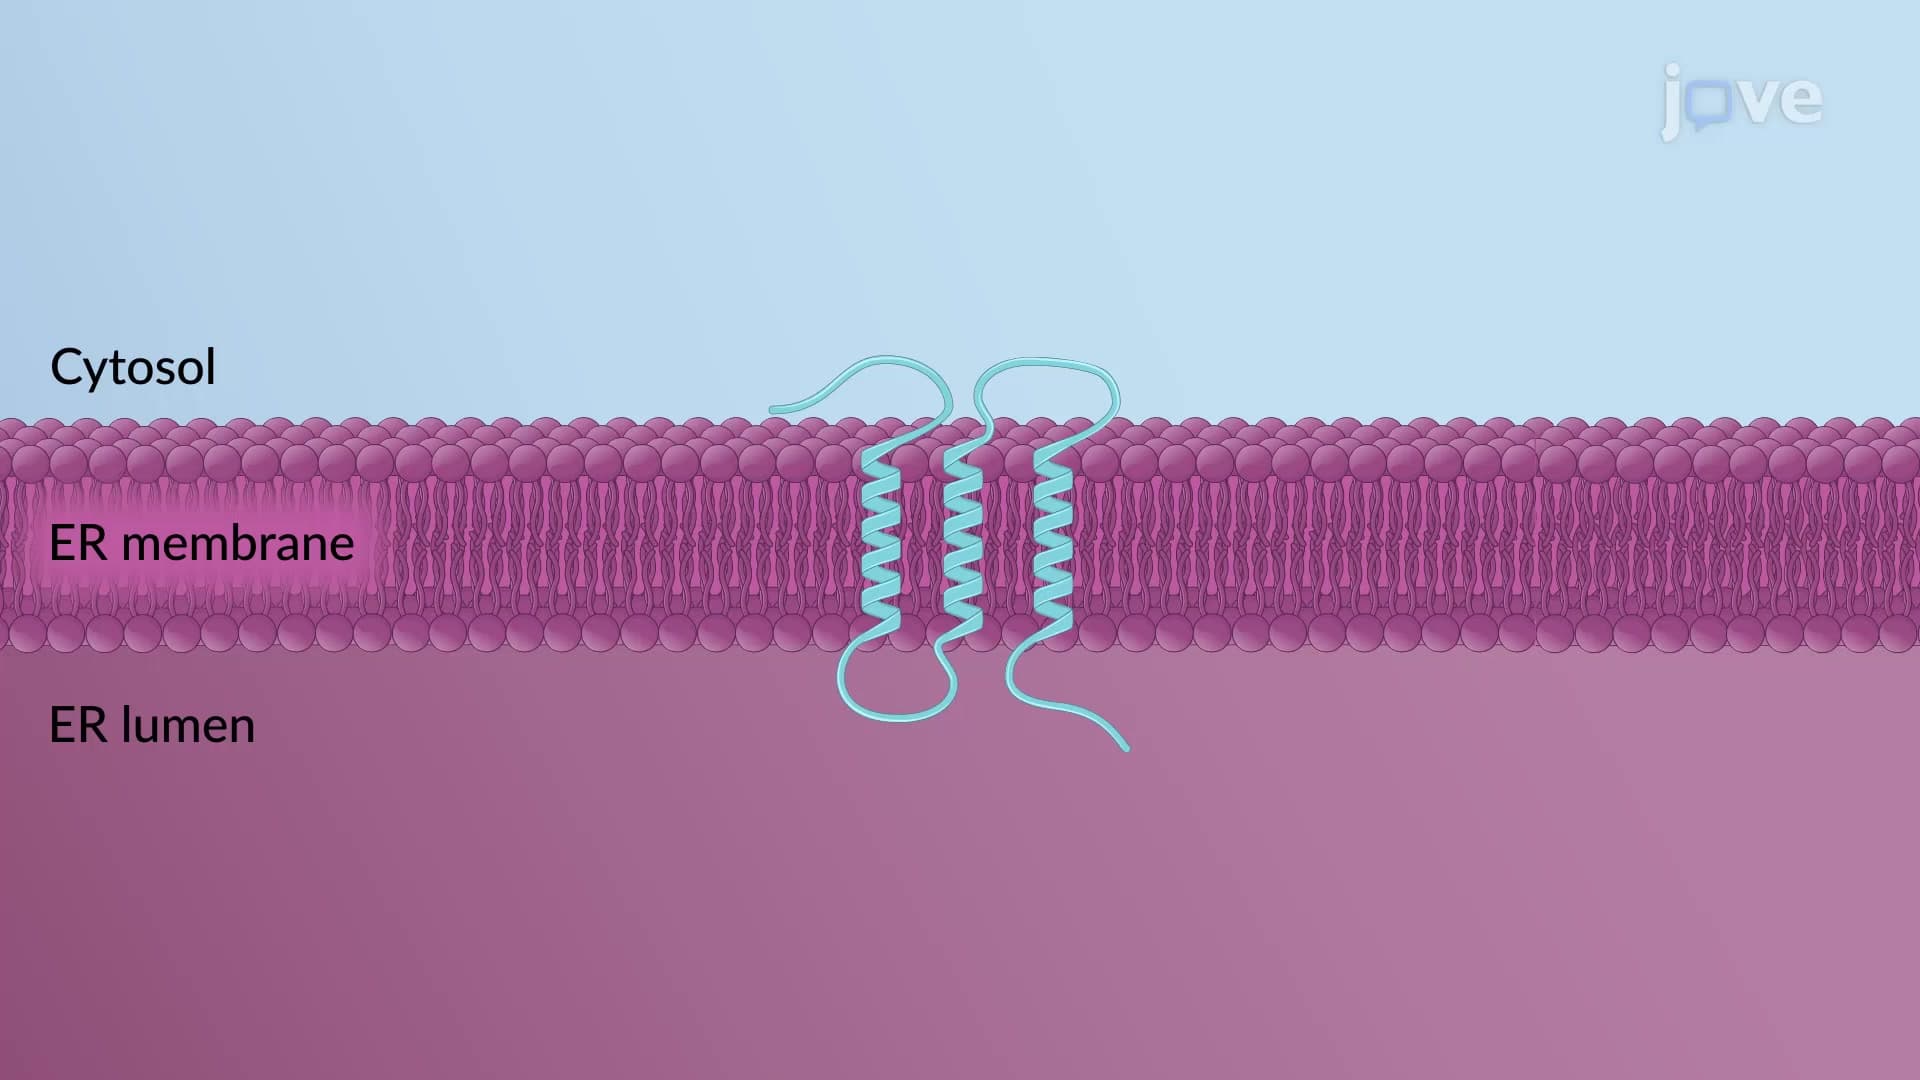
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
 01:45
Tail-anchoring of Proteins in the ER Membrane
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum