SNAREs--engines for membrane fusion

Reinhard Jahn1, Richard H Scheller

  • 1Department of Neurobiology, Max Planck Institute for Biophysical Chemistry, Am Fassberg, 37077 Göttingen, Germany. rjahn@gwdg.de

Related Concept Videos

SNAREs and Membrane Fusion01:43

SNAREs and Membrane Fusion

Once a transport vesicle has recognized its target organelle, the vesicular membrane needs to fuse with the target membrane to unload the cargo. Transmembrane proteins called SNAREs present on organelle membranes and their vesicles, mediate vesicle fusion.
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
Fusion of Secretory Vesicles with the Plasma Membrane01:26

Fusion of Secretory Vesicles with the Plasma Membrane

Proteins and neurotransmitters in secretory vesicles can be released from a cell upon vesicle docking, priming, and fusion with the plasma membrane. Vesicles are docked and primed in preparation for the quick exocytosis of their contents in response to a stimulus. The fusion process is mainly carried out by a SNAP Receptor or SNARE complex, consisting of synaptobrevin, syntaxin-1, and SNAP-25.
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
Rab Cascades01:25

Rab Cascades

Rab GTPases act in a regulated cascade during membrane fusion, helping the lipid bilayers mix. The Rab family of proteins are active when bound to GTP, and inactive when bound to GDP. Hence, they act as guanine nucleotide-dependent molecular switches. Rab-GTP recognizes and binds to long or short-range tethering proteins to capture the target vesicle. These tethers coordinate with SNAREs on the vesicle and the target membrane to assemble the trans SNARE complex that locks the mixing bilayers.
Mechanisms of Membrane Domain Formation00:59

Mechanisms of Membrane Domain Formation

Different physical properties of lipids and proteins allow them to localize and form distinct islands or domains in the membrane. Some membrane domains are formed due to protein-protein interactions, whereas others are formed due to the presence of specific lipids such as sphingolipids and sterols—for example, large proteins, such as bacteriorhodopsin, aggregate and create distinct domains.
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
Protein Translocation Machinery on the ER Membrane01:28

Protein Translocation Machinery on the ER Membrane

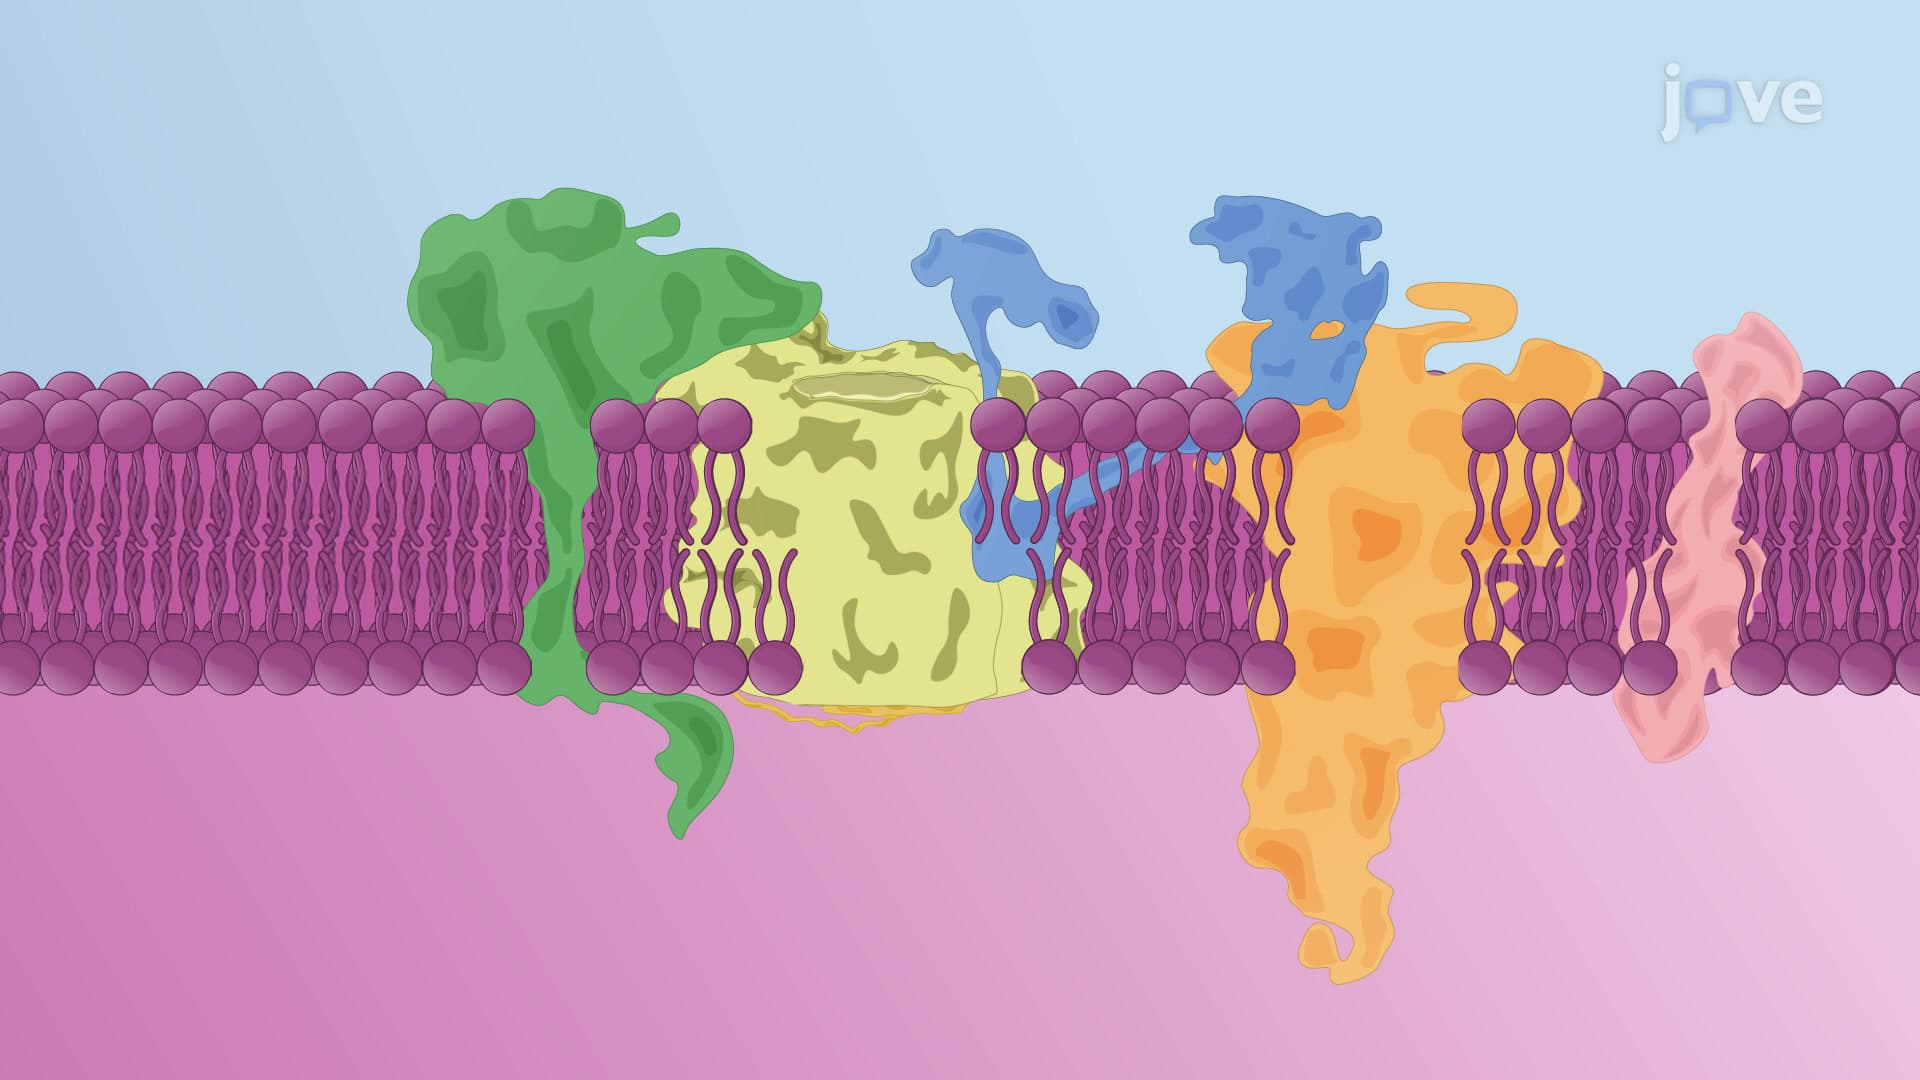
The translocon complex situated on the ER membrane is the main gateway for the protein secretory pathway. It facilitates the transport of nascent peptides into the ER lumen and their insertion into the ER membrane.
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
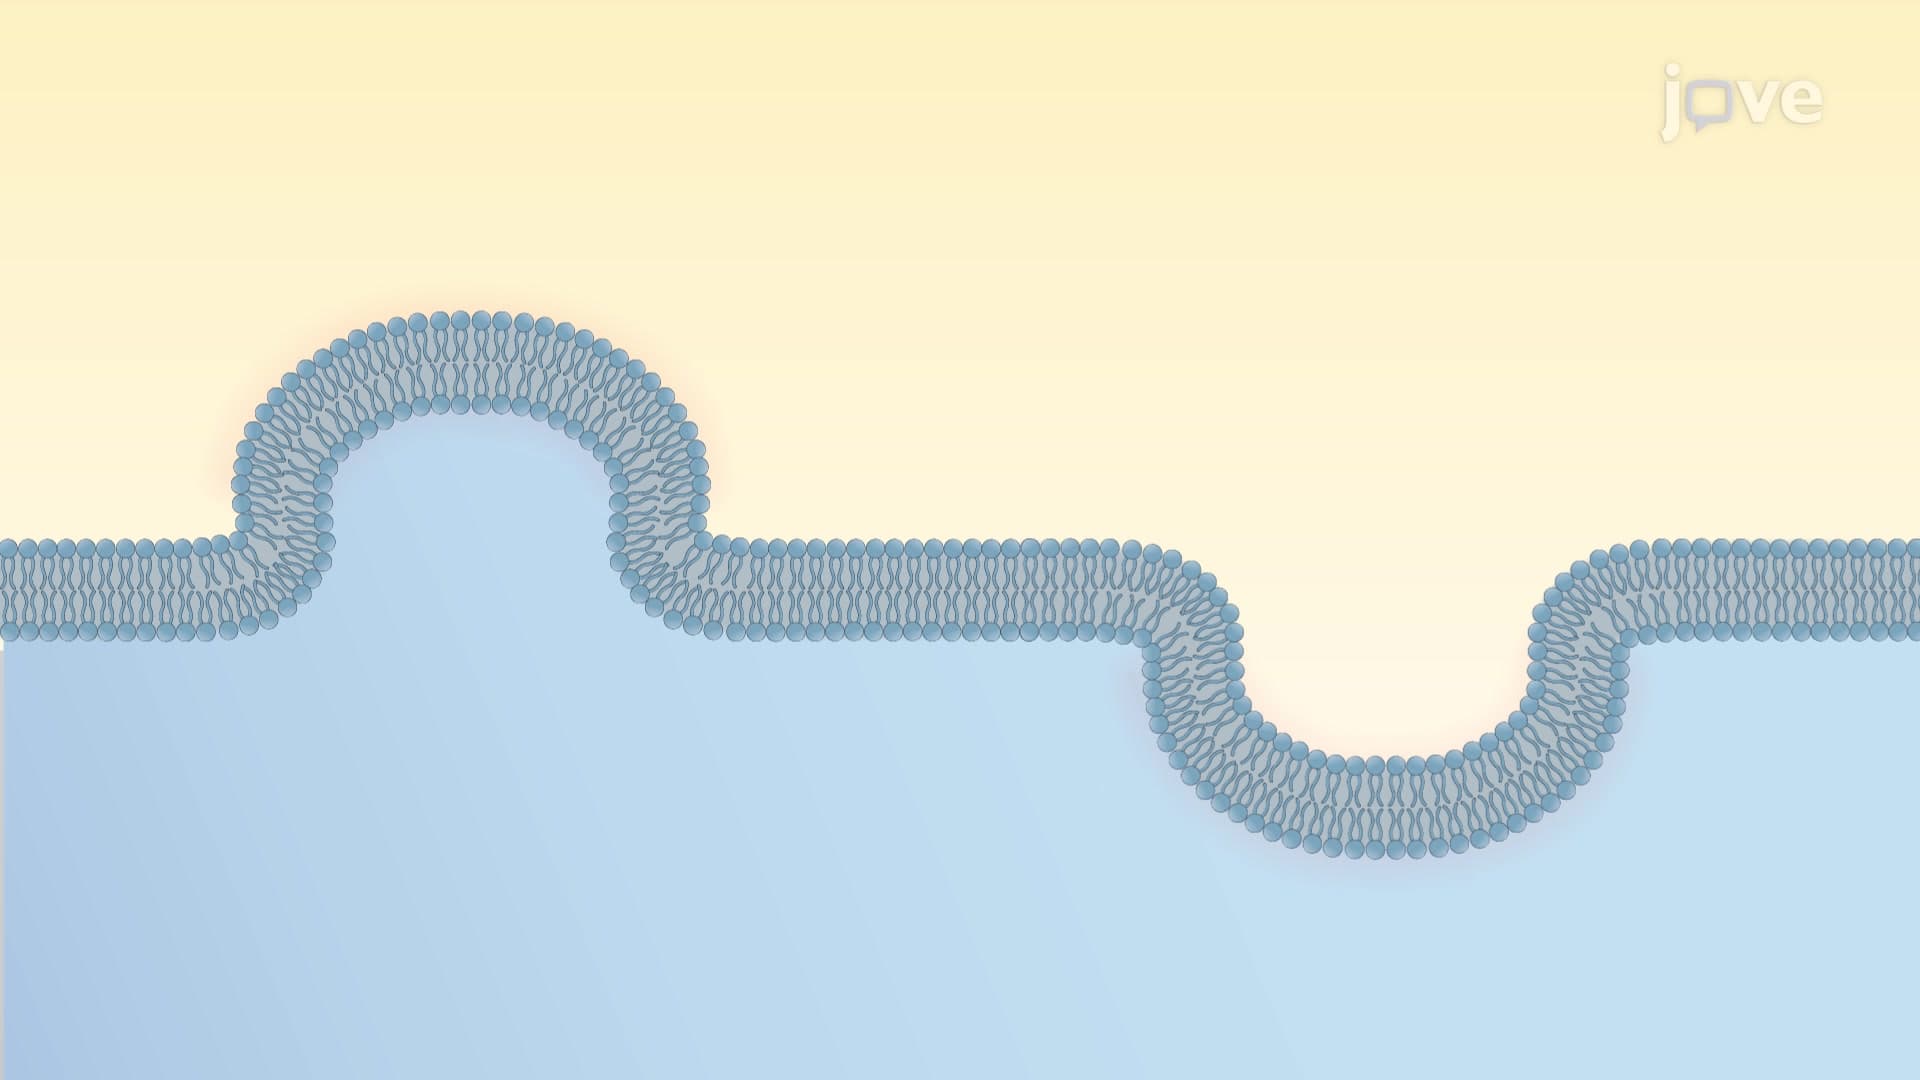
Mechanisms of Membrane-bending01:15

Mechanisms of Membrane-bending

The living membranes are flexible due to their fluid mosaic nature; however, their bending into different shapes is an active process regulated by specific lipids and proteins. The membrane bending can be transient as seen in vesicles or stable for a long time as in microvilli. Cells regulate the size, location, and duration of the membrane curvature.
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...