Related Experiment Video
Updated: Jul 19, 2026

Purification of the Membrane Compartment for Endoplasmic Reticulum-associated Degradation of Exogenous Antigens in Cross-presentation
Published on: August 21, 2017
Need for tripeptidyl-peptidase II in major histocompatibility complex class I viral antigen processing when
Sara Guil1, Marta Rodríguez-Castro, Francisco Aguilar
1Unidad de Inmunología Viral, Centro Nacional de Microbiología, Instituto de Salud Carlos III, E-28220 Majadahonda (Madrid), Spain.

CD8(+) T lymphocytes recognize infected cells that display virus-derived antigenic peptides complexed with major histocompatibility complex class I molecules. Peptides are mainly byproducts of cellular protein turnover by cytosolic proteasomes. Cytosolic tripeptidyl-peptidase II (TPPII) also participates in protein degradation. Several peptidic epitopes unexpectedly do not require proteasomes, but it is unclear which proteases generate them. We studied antigen processing of influenza virus nucleoprotein epitope NP(147-155), an archetype epitope that is even destroyed by a proteasome-mediated mechanism. TPPII, with the assistance of endoplasmic reticulum trimming metallo-aminopeptidases, probably ERAAP (endoplasmic reticulum aminopeptidase associated with antigen processing), was crucial for nucleoprotein epitope generation both in the presence of functional proteasomes and when blocked by lactacystin, as shown with specific chemical inhibitors and gene silencing. Different protein contexts and subcellular targeting all allowed epitope processing by TPPII as well as trimming. The results show the plasticity of the cell's assortment of proteases for providing ligands for recognition by antiviral CD8(+) T cells. Our observations identify for the first time a set of proteases competent for antigen processing of an epitope that is susceptible to destruction by proteasomes.
CD8(+) T lymphocytes recognize infected cells that display virus-derived antigenic peptides complexed with major histocompatibility complex class I molecules. Peptides are mainly byproducts of cellular protein turnover by cytosolic proteasomes. Cytosolic tripeptidyl-peptidase II (TPPII) also participates in protein degradation. Several peptidic epitopes unexpectedly do not require proteasomes, but it is unclear which proteases generate them. We studied antigen processing of influenza virus nucleoprotein epitope NP(147-155), an archetype epitope that is even destroyed by a proteasome-mediated mechanism. TPPII, with the assistance of endoplasmic reticulum trimming metallo-aminopeptidases, probably ERAAP (endoplasmic reticulum aminopeptidase associated with antigen processing), was crucial for nucleoprotein epitope generation both in the presence of functional proteasomes and when blocked by lactacystin, as shown with specific chemical inhibitors and gene silencing. Different protein contexts and subcellular targeting all allowed epitope processing by TPPII as well as trimming. The results show the plasticity of the cell's assortment of proteases for providing ligands for recognition by antiviral CD8(+) T cells. Our observations identify for the first time a set of proteases competent for antigen processing of an epitope that is susceptible to destruction by proteasomes.
Related Concept Videos
 01:31
Antigen Processing Pathways
MHC Class I: Presenting Endogenous...
 01:26
Antigens Involved in Adaptive Immunity
Complete Antigens
Complete antigens possess both immunogenicity and reactivity.
 01:13
The Proteasome
In this pathway, the target proteins are first tagged with small proteins called ubiquitin. This involves participation of a series of enzymes including— E1 (ubiquitin-activating enzyme), E2 (ubiquitin-conjugating enzyme), and E3 (ubiquitin...
 02:18
The Proteasome
In this pathway, the target proteins are first tagged with small proteins called ubiquitin. A series of enzymes carry out the ubiquitination of the target proteins - E1 (ubiquitin-activating enzyme), E2 (ubiquitin-conjugating enzyme), and E3...
 01:19
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:19
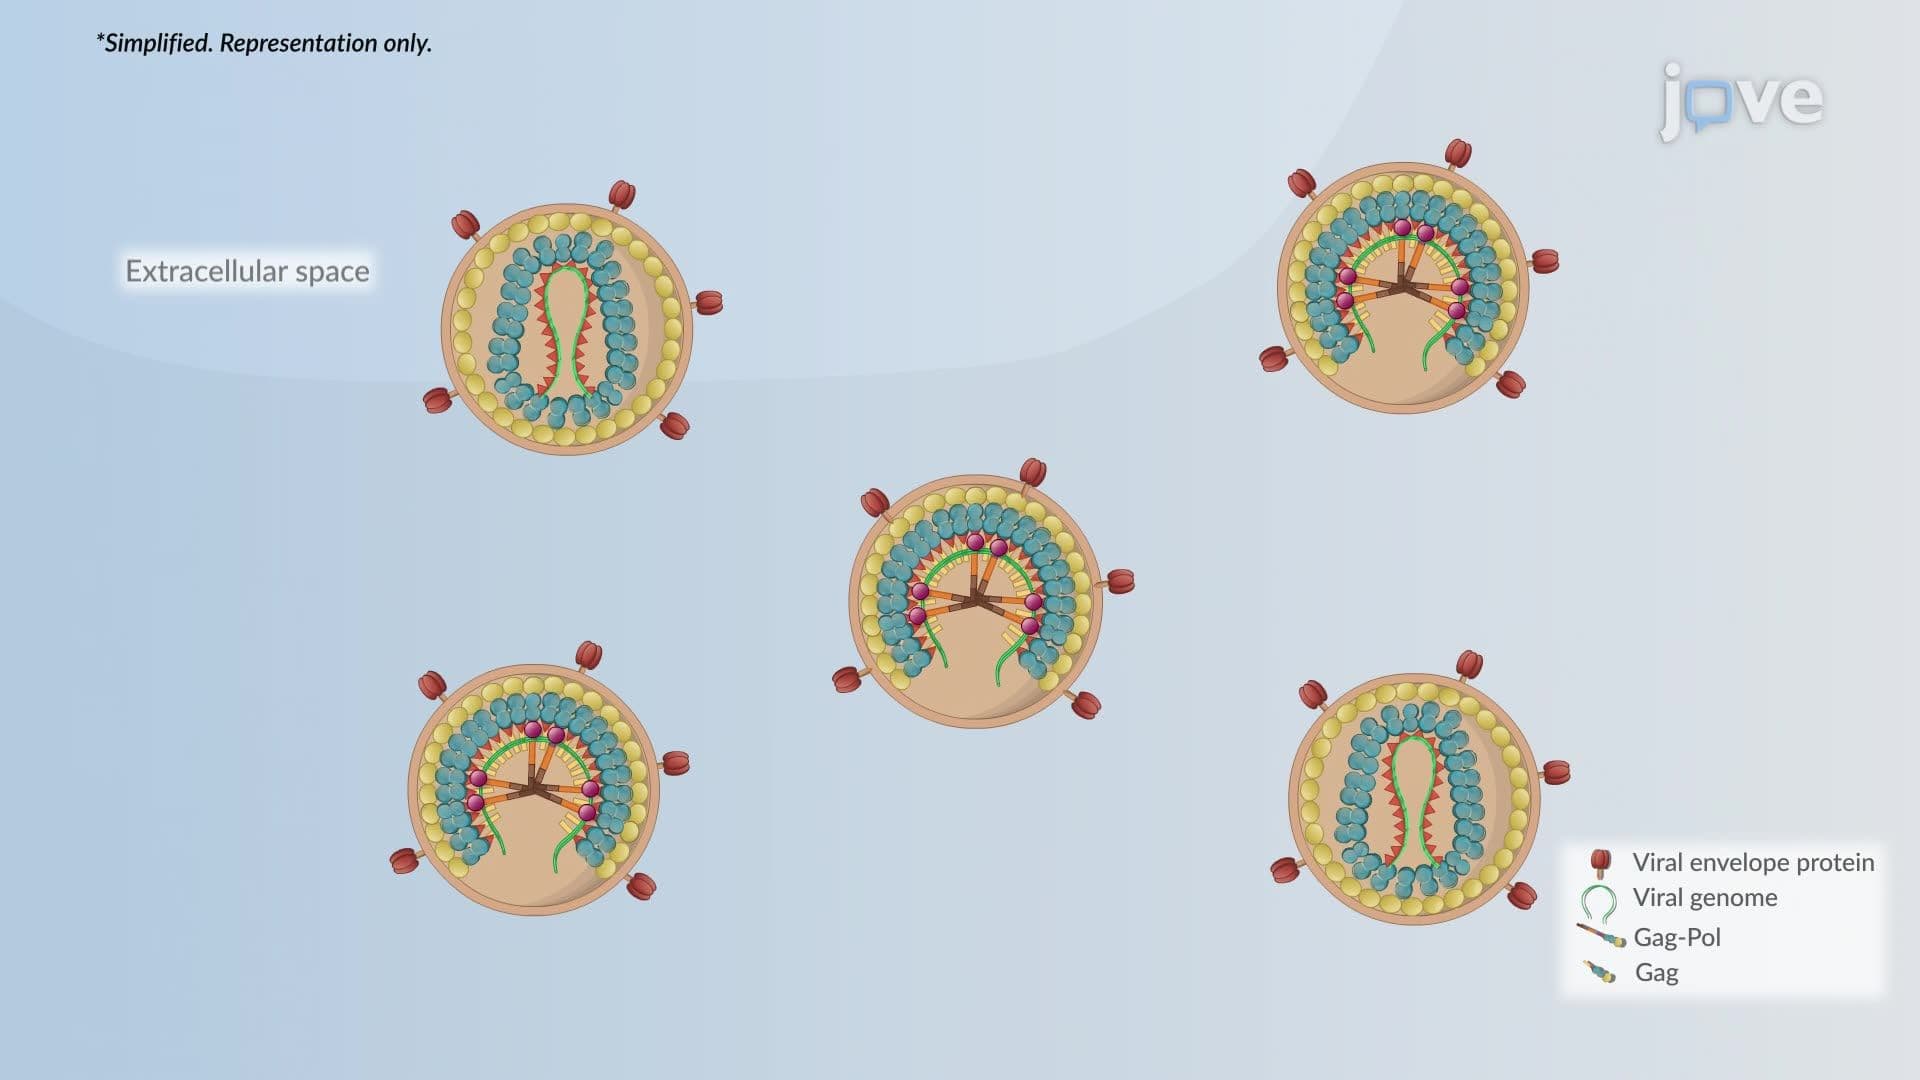
Inhibitors of Virion Maturation and Assembly