Related Experiment Video
Updated: Jul 18, 2026

Genetic Screen for Identification of Multicopy Suppressors in Schizosaccharomyces pombe
Published on: September 13, 2022
The end1 gene of Schizosaccharomyces pombe coding for a DNase is identical with the pnu1 gene coding for an RNase
1Institute of Cell Biology, University of Bern, CH-3012 Bern, Switzerland.

Abstract:
The DNA nuclease activity encoded by the end1 gene, and its inactivation by mutation, was described in connection with the characterization of DNA topoisomerases in the fission yeast Schizosaccharomyces pombe (Uemura and Yanagida, 1984). Subsequently, end1 mutant strains were used for the preparation of cell extracts for the study of enzymes and intermediates involved in DNA metabolism. The molecular identification of the end1 gene and its identity with the pnu1 gene is presented. The end1-458 mutation alters glycine to glutamate in the conserved motif TGPYLP. The pnu1 gene codes for an RNase that is induced by nitrogen starvation (Nakashima et al., 2002b). Thus, the End1/Pnu1 protein, like related mitochondrial proteins in other organisms, is an example of a sugar-non-specific nuclease. The analysis of strains carrying a pnu1 deletion revealed no defects in meiotic recombination and spore viability.
Related Concept Videos
 00:58
Eukaryotic RNA Polymerases
All three eukaryotic RNAPs require specific transcription factors, of which the...
 02:57
piRNA - Piwi-interacting RNAs
 03:18
Non-LTR Retrotransposons
 02:53
Ribosomal RNA Synthesis
Ribosome biogenesis begins with the synthesis of 5S and 45S pre-rRNAs by distinct RNA polymerases. The primary transcripts are extensively processed and modified before they are bound and folded by ribosomal proteins and assembly factors,...
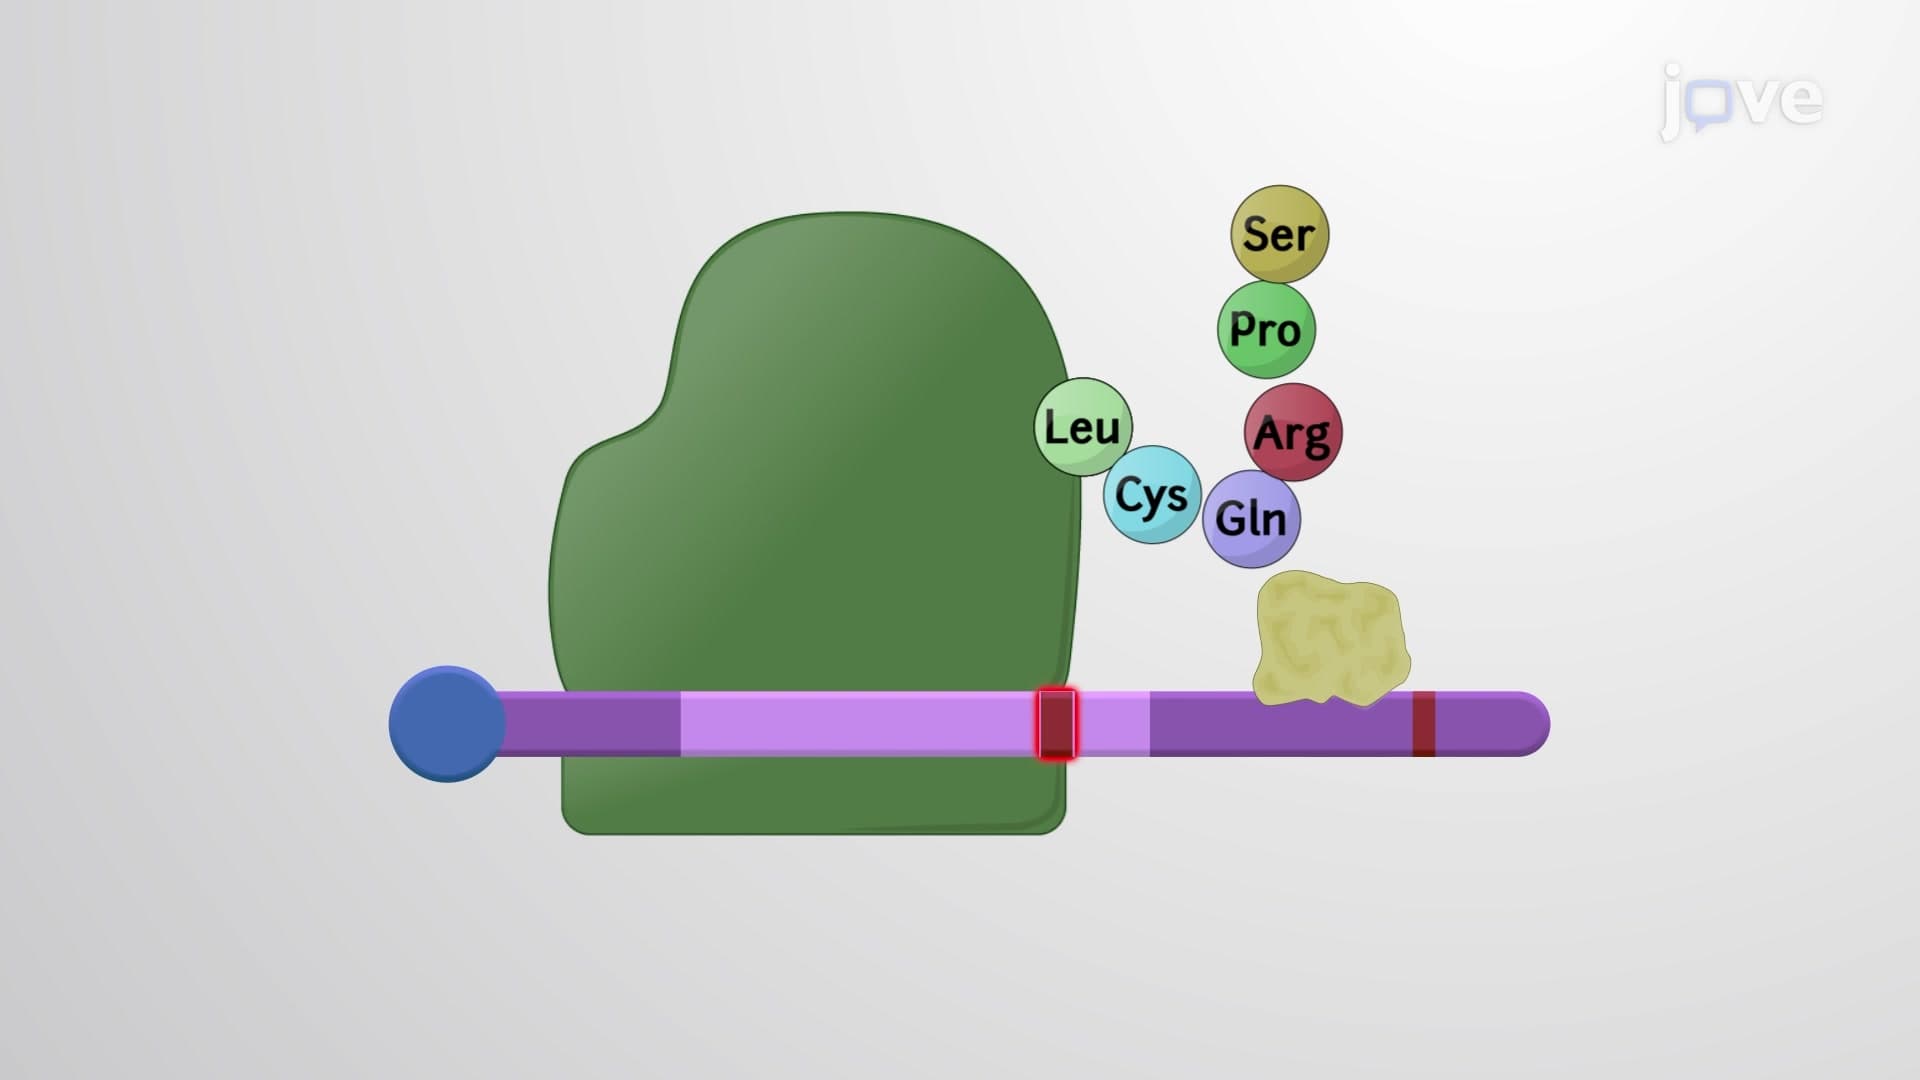 02:27
Nonsense-mediated mRNA Decay
Usually, Upf3 binds to an Exon Junction Complex (EJC) at mRNA splice sites. If a ribosome fully translates the mRNA,...
 02:32
Exon Recombination
Exon shuffling follows “splice frame rules.” Each exon has three reading...