Related Experiment Video
Updated: Jul 13, 2026

A High-content Assay for Monitoring AMPA Receptor Trafficking
Published on: January 28, 2019
Rigidity of the subunit interfaces of the trimeric glutamate transporter GltT during translocation
Maarten Groeneveld1, Dirk-Jan Slotboom
1Department of Biochemistry, University of Groningen, Groningen Biomolecular Science and Biotechnology Institute, Nijenborgh 4, 9747 AG Groningen, The Netherlands.

Abstract:
Glutamate transporters are trimeric membrane proteins in which each protomer contains a separate translocation path. To determine whether structural rearrangements take place at the subunit interfaces during transport, intersubunit disulfide bridges were introduced in the bacterial transporter GltT. None of the intersubunit cross-links, which had been designed across the entire interface, affected the glutamate transport activity, indicating that the subunit interfaces are rigid during turnover.
Related Concept Videos
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
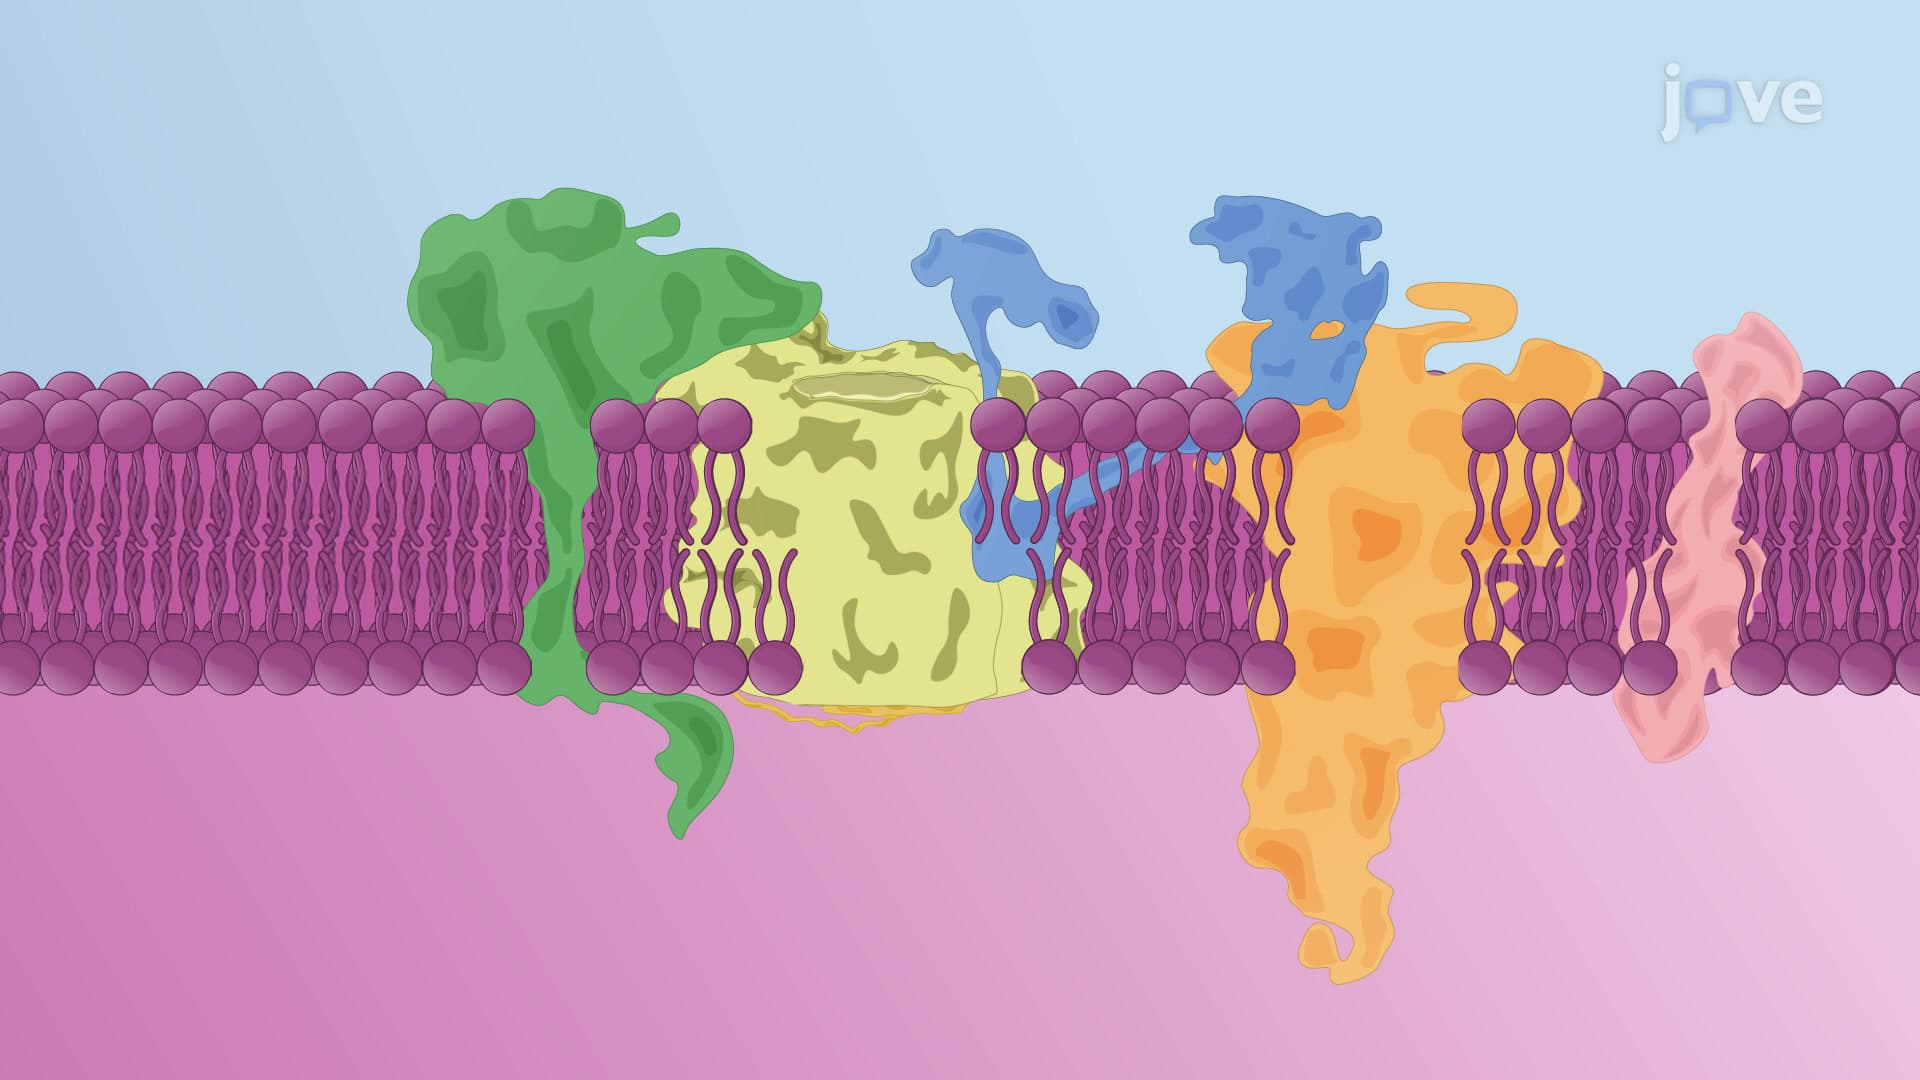
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
 01:37
Energy to Drive Translocation
Generally, polypeptides are unfolded by two distinct...
 01:34
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...
 01:27
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
 01:29
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...