Related Experiment Video
Updated: Jul 7, 2026
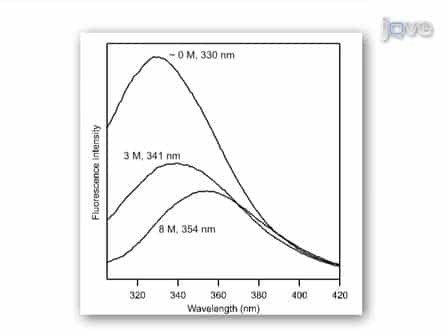

Thermodynamics of Membrane Protein Folding Measured by Fluorescence Spectroscopy
Published on: April 28, 2011
Estimating free-energy barrier heights for an ultrafast folding protein from calorimetric and kinetic data
Raquel Godoy-Ruiz1, Eric R Henry, Jan Kubelka
1Departamento de Quimica Fisica Facultad de Ciencias, Universidad de Granada, 18071 Granada, Spain.

Abstract:
Differential scanning calorimetry was used to measure the temperature dependence of the absolute heat capacity of the 35-residue subdomain of the villin headpiece, a protein that folds in 5 mus and is therefore assumed to have a small free-energy barrier separating folded and unfolded states. To obtain an estimate of the barrier height from the calorimetric data, two models, a variable-barrier model and an Ising-like model, were used to fit the heat capacity in excess of the folded state over the temperature range 15-125 degrees C. The variable-barrier model is based on an empirical mathematical form for the density of states, with four adjustable parameters and the enthalpy (H) as a reaction coordinate. The Ising-like model is based on the inter-residue contact map of the X-ray structure with exact enumeration of approximately 10(5) possible conformations, with two adjustable parameters in the partition function, and either the fraction of native contacts (Q) or the number of ordered residues (P) as reaction coordinates. The variable-barrier model provides an excellent fit to the data and yields a barrier height at the folding temperature ranging from 0.4 to 1.1 kcal mol(-1), while the Ising-like model provides a less good fit and yields barrier heights of 2.3 +/- 0.1 kcal mol(-1) and 2.1 +/- 0.1 kcal mol(-1) for the Q and P reaction coordinates, respectively. In both models, the barrier to folding increases with increasing temperature. Assuming a sufficiently large activation energy for diffusion on the free-energy surfaces, both models are consistent with the observation of a temperature-independent folding rate in previously published laser temperature-jump experiments. Analysis of this kinetic data, using an approximate form for the pre-exponential factor of Kramers theory and the 70 ns relaxation time for the fast phase that precedes the unfolding/refolding relaxation to determine the diffusion coefficient, results in a barrier height of 1.6 +/- 0.3 kcal mol-1 for an unspecified reaction coordinate. Although no independent test of the validity of the H, Q, or P reaction coordinates is given, the barrier-height estimates obtained with the three reaction coordinates are in quite good agreement with the value derived from a Kramers analysis of the kinetics that makes no assumptions about the reaction coordinate. However, the higher estimates obtained using Q or P appear more consistent with the finding of barrier-crossing kinetics of a villin mutant that folds in 700 ns, corresponding to a 1.3 kcal mol-1 reduction in the folding barrier relative to wild-type. All of the results suggest that the free-energy barrier to folding is sufficiently low that it should be possible to engineer this protein or find solution conditions that would eliminate the barrier to create the "downhill" folding scenario of Wolynes and Onuchic.
Related Concept Videos
 01:19
Protein Dynamics in Living Cells
Fluorescent recovery after photobleaching (FRAP) is a fluorescent-protein-based detection technique used to quantify protein movement rates within the cell. This method exposes a small portion of the cell to an intense laser beam. The laser beam causes permanent photobleaching of the fluorophore-tagged proteins in the exposed region. As the bleached...
 02:18
The Equilibrium Binding Constant and Binding Strength
 01:22
Protein Folding