Insect ion transport peptides are derived from alternatively spliced genes and differentially expressed in the central and peripheral nervous system
Related Experiment Video
Updated: Jun 26, 2026
In vivo Interrogation of Central Nervous System Translatome by Polyribosome Fractionation
Published on: April 30, 2014
1Department of Zoology, Stockholm University, Svante Arrhenius väg 14, 10691 Stockholm, Sweden. dircksen@zoologi.su.se

Abstract:
Insect ionic and fluid homeostasis relies upon the Malpighian tubules (MT) and different hindgut compartments. Primary urine formed in MTs is finally modified by ion, solute and water reabsorptive processes primarily in the hindgut under the control of several large peptide hormones. One of these, the ion transport peptide (ITP), is a chloride transport-stimulating and acid secretion-inhibiting hormone similar to crustacean hyperglycaemic hormones (CHHs). In locusts, moths and fruit flies, ITP together with the slightly longer ITPL isoforms, inactive in hindgut bioassays, arise by alternative splicing from very similar itp genes. ITP and ITPL are differentially distributed in (1) pars lateralis/retrocerebral complex neurosecretory cells (NSCs) containing both splice forms, (2) interneurons with either one of the splice forms, (3) hindgut-innervating abdominal ITP neurons (in Drosophila only), and (4) intrinsic, putative sensory NSCs in peripheral neurohaemal perisympathetic/perivisceral organs or transverse nerves (usually containing ITPL). Both splice forms occur as hormones released into the haemolymph in response to feeding or stress stimuli. ITPL mainly released from the peripheral NSCs is discussed as a competitive inhibitor (as established in vitro) of ITP action on yet to be identified hindgut ITP receptors. Furthermore, some evidence has been provided for possible ecdysis-related functions of ITP and/or ITPL in moths. The comparative data on the highly similar gene, precursor and primary structures and similar differential distributions in insect and crustacean NSCs suggest that CHH/ITP and ITPL neuropeptide-producing cells and their gene products share common phylogenetic ancestry.
Related Concept Videos
 01:19
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:34
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...
 01:45
Overview of Protein Sorting and Transport
Protein sorting can be of two types: signal-based sorting and vesicle-based trafficking. In signal-based sorting, specific amino acid sequences called sorting signals target proteins to the proper location inside the cell either via gated transport or by protein translocation. In gated transport, folded...
 02:18
Alternative RNA Splicing
There are five types of alternative RNA splicing that vary in the ways the pre-mRNA segments are removed or retained in the mature mRNA. The first...
 01:27
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
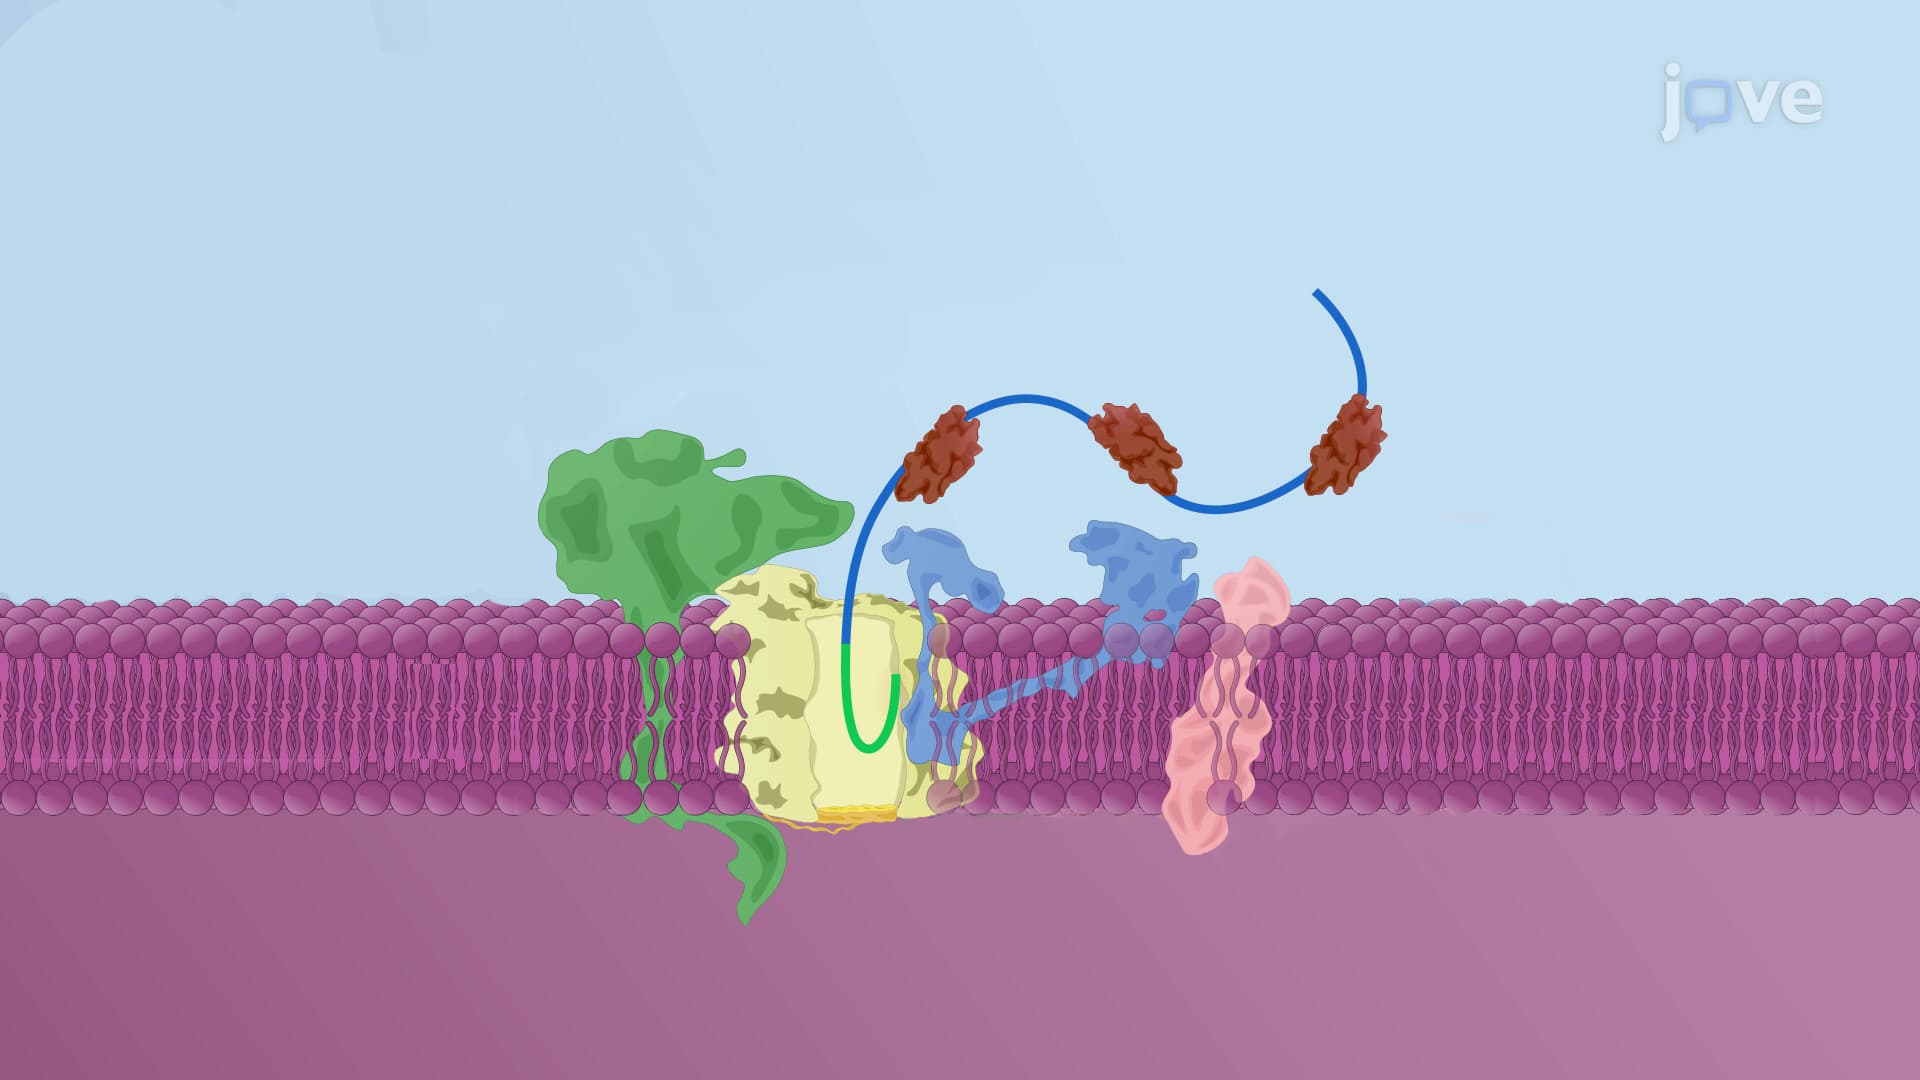
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
 01:19
Membrane Asymmetry Regulating Transporters
Flippase
Eukaryotic flippases are type-IV P-type ATPases or P4-ATPases belonging to P-type ATPase family proteins that are membrane-bound pumps involved in the ATP-mediated transport of ions and molecules across the membrane. Flippases flip specific phospholipids from the outer to the inner leaflet of a membrane. All P4-ATPases have one...