Energetics of stalk intermediates elucidated from hydrostatic pressure effects on membrane fusion
Daniel Milshteyn1, Jacob R Winnikoff2, Joel E Morgan3
1Department of Biochemistry & Molecular Biophysics, University of California San Diego, La Jolla, CA, USA.

Abstract:
Membrane fusion is an essential process in cells that requires a balance of lipid composition to establish biophysical properties conducive to topology changes. During fusion, lipids of opposing membranes must invert and overcome energy barriers associated with forming highly curved stalk and pore intermediates. While theoretical work has modeled the effect of lipid intrinsic curvature on stalk formation, quantifying the relationship experimentally has proven to be a challenge due to the inability to vary lipid curvature without concomitantly changing other properties that affect fusion. Here we address this hurdle by using hydrostatic pressure to modulate lipid intrinsic curvature independently of chemical composition. Using high-pressure stopped-flow fluorimetry, we measured rates of calcium-mediated lipid mixing between populations of vesicles, a process that is strongly inhibited by pressure. We correlated mean lipid intrinsic curvature across pressure with lipid mixing rates by incorporating complementary small-angle x-ray scattering measurements for each individual lipid component. This analysis showed that lipid mixing rates, a proxy for hemifusion, correlated with mean monolayer spontaneous curvature as we varied either lipid composition or pressure. Consistent with previous theoretical models, we find a linear relation between lipid monolayer spontaneous curvature and the energy barrier to lipid mixing; the slope magnitude of this relation supports the stalk hypothesis.
Related Concept Videos
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:15
Mechanisms of Membrane-bending
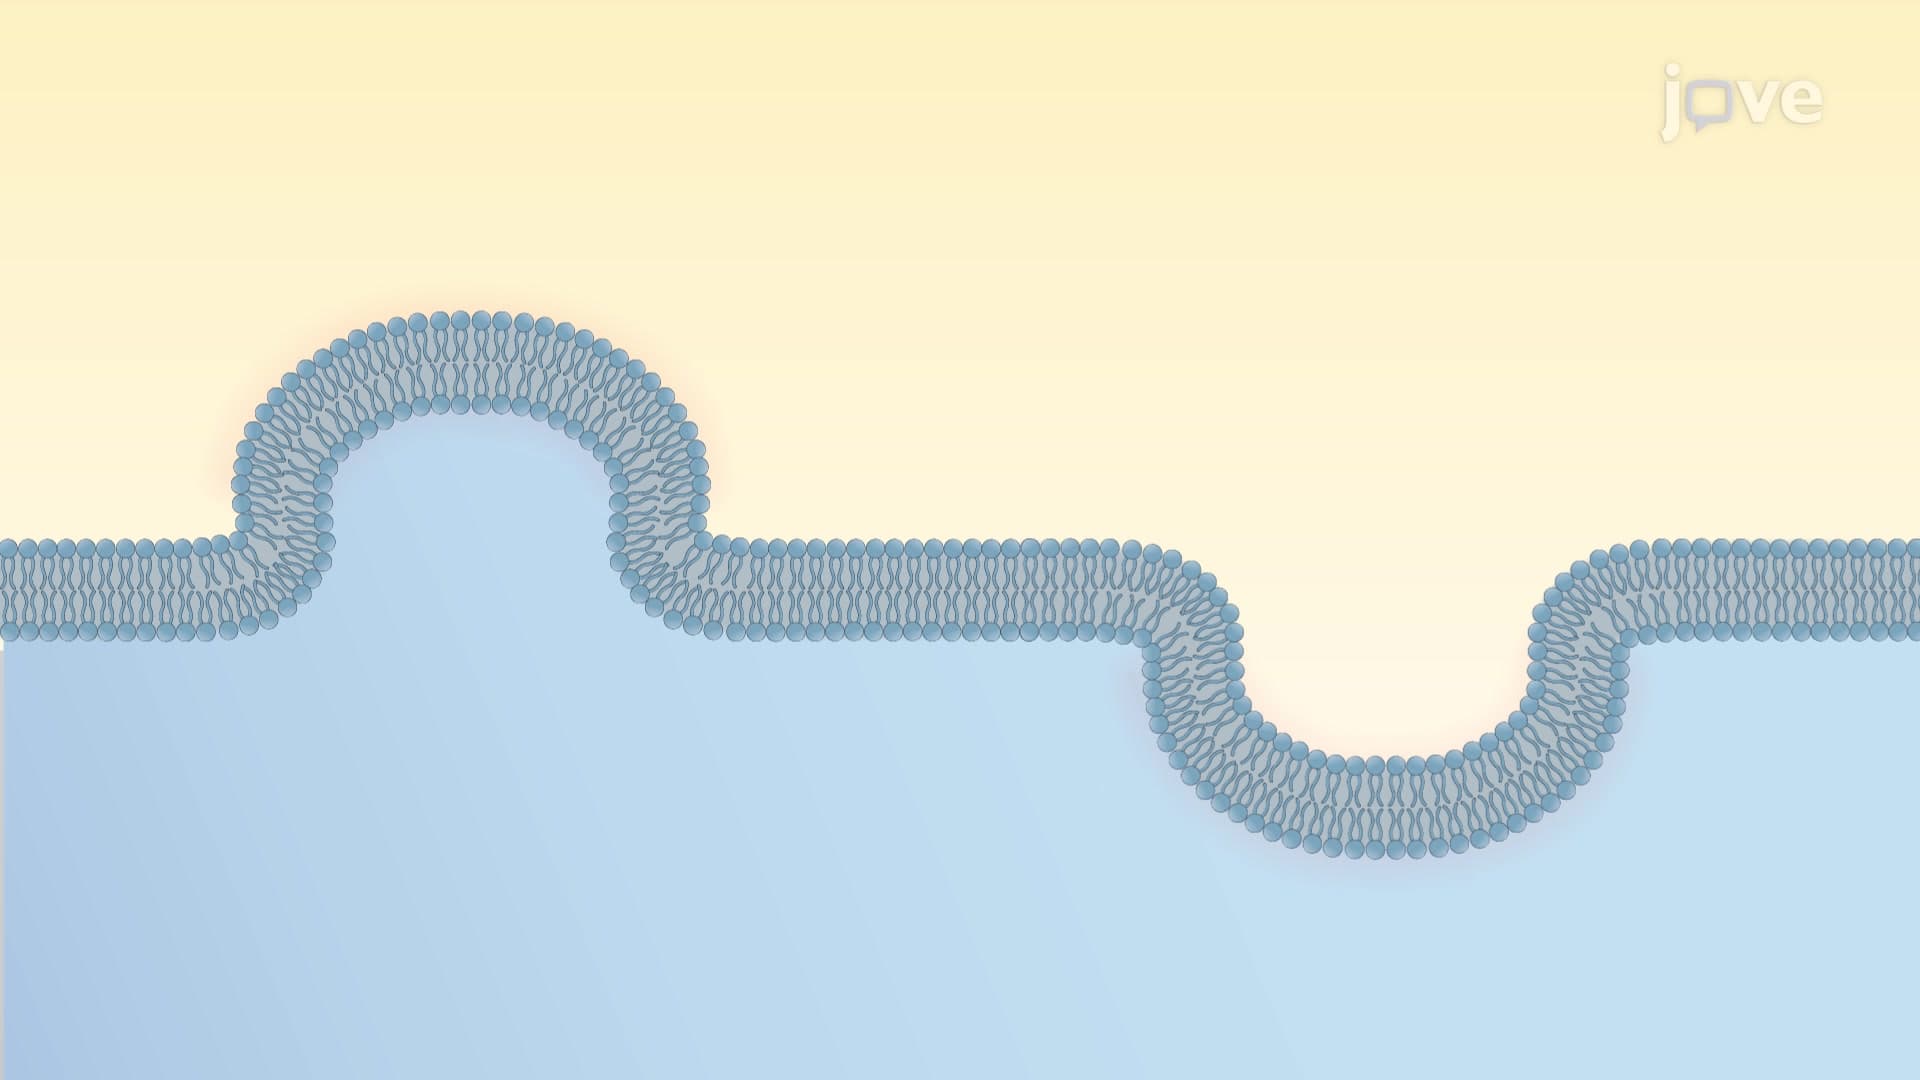
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
 01:27
ATP Driven Pumps I: An Overview
There are four main types of ATP-driven pumps - P-type, V-type, F-type, and ABC transporter. All these pumps are of varying complexities and are...
 01:32
Pinching-off of Coated Vesicles
 01:18
ATP Synthase: Structure
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...