Related Experiment Video
Updated: May 23, 2026

In Vitro Ubiquitination and Deubiquitination Assays of Nucleosomal Histones
Published on: July 25, 2019
Ubiquitination is involved in secondary growth, not initial formation of polyglutamine protein aggregates in C.
Gregory A Skibinski1, Lynn Boyd
1Department of Biological Sciences, University of Alabama in Huntsville, Huntsville AL 35899, USA. boydl@uah.edu

Background:
Protein misfolding and subsequent aggregation are hallmarks of several human diseases. The cell has a variety of mechanisms for coping with misfolded protein stress, including ubiquitin-mediated protein degradation. In fact, the presence of ubiquitin at protein aggregates is a common feature of protein misfolding diseases. Ubiquitin conjugating enzymes (UBCs) are part of the cascade of enzymes responsible for the regulated attachment of ubiquitin to protein substrates. The specific UBC used during ubiquitination can determine the type of polyubiquitin chain linkage, which in turn plays an important role in determining the fate of the ubiquitinated protein. Thus, UBCs may serve an important role in the cellular response to misfolded proteins and the fate of protein aggregates.
Results:
The Q82 strain of C. elegans harbors a transgene encoding an aggregation prone tract of 82 glutamine residues fused to green fluorescent protein (Q82::GFP) that is expressed in the body wall muscle. When measured with time-lapse microscopy in young larvae, the initial formation of individual Q82::GFP aggregates occurs in approximately 58 minutes. This process is largely unaffected by a mutation in the C. elegans E1 ubiquitin activating enzyme. RNAi of ubc-22, a nematode homolog of E2-25K, resulted in higher pre-aggregation levels of Q82::GFP and a faster initial aggregation rate relative to control. Knockdown of ubc-1 (RAD6 homolog), ubc-13, and uev-1 did not affect the kinetics of initial aggregation. However, RNAi of ubc-13 decreases the rate of secondary growth of the aggregate. This result is consistent with previous findings that aggregates in young adult worms are smaller after ubc-13 RNAi. mCherry::ubiquitin becomes localized to Q82::GFP aggregates during the fourth larval (L4) stage of life, a time point long after most aggregates have formed. FLIP and FRAP analysis indicate that mCherry::ubiquitin is considerably more mobile than Q82::GFP within aggregates.
Conclusions:
These data indicate that initial formation of Q82::GFP aggregates in C. elegans is not directly dependent on ubiquitination, but is more likely a spontaneous process driven by biophysical properties in the cytosol such as the concentration of the aggregating species. The effect of ubiquitination appears to be most significant in later, secondary aggregate growth.
Related Concept Videos
 02:58
Regulated Protein Degradation
Protein degradation plays two important roles in the cells. It helps to protect cells from misfolded or damaged proteins before they lead to a...
 01:29
Protein Folding Quality Check in the RER
 01:13
The Proteasome
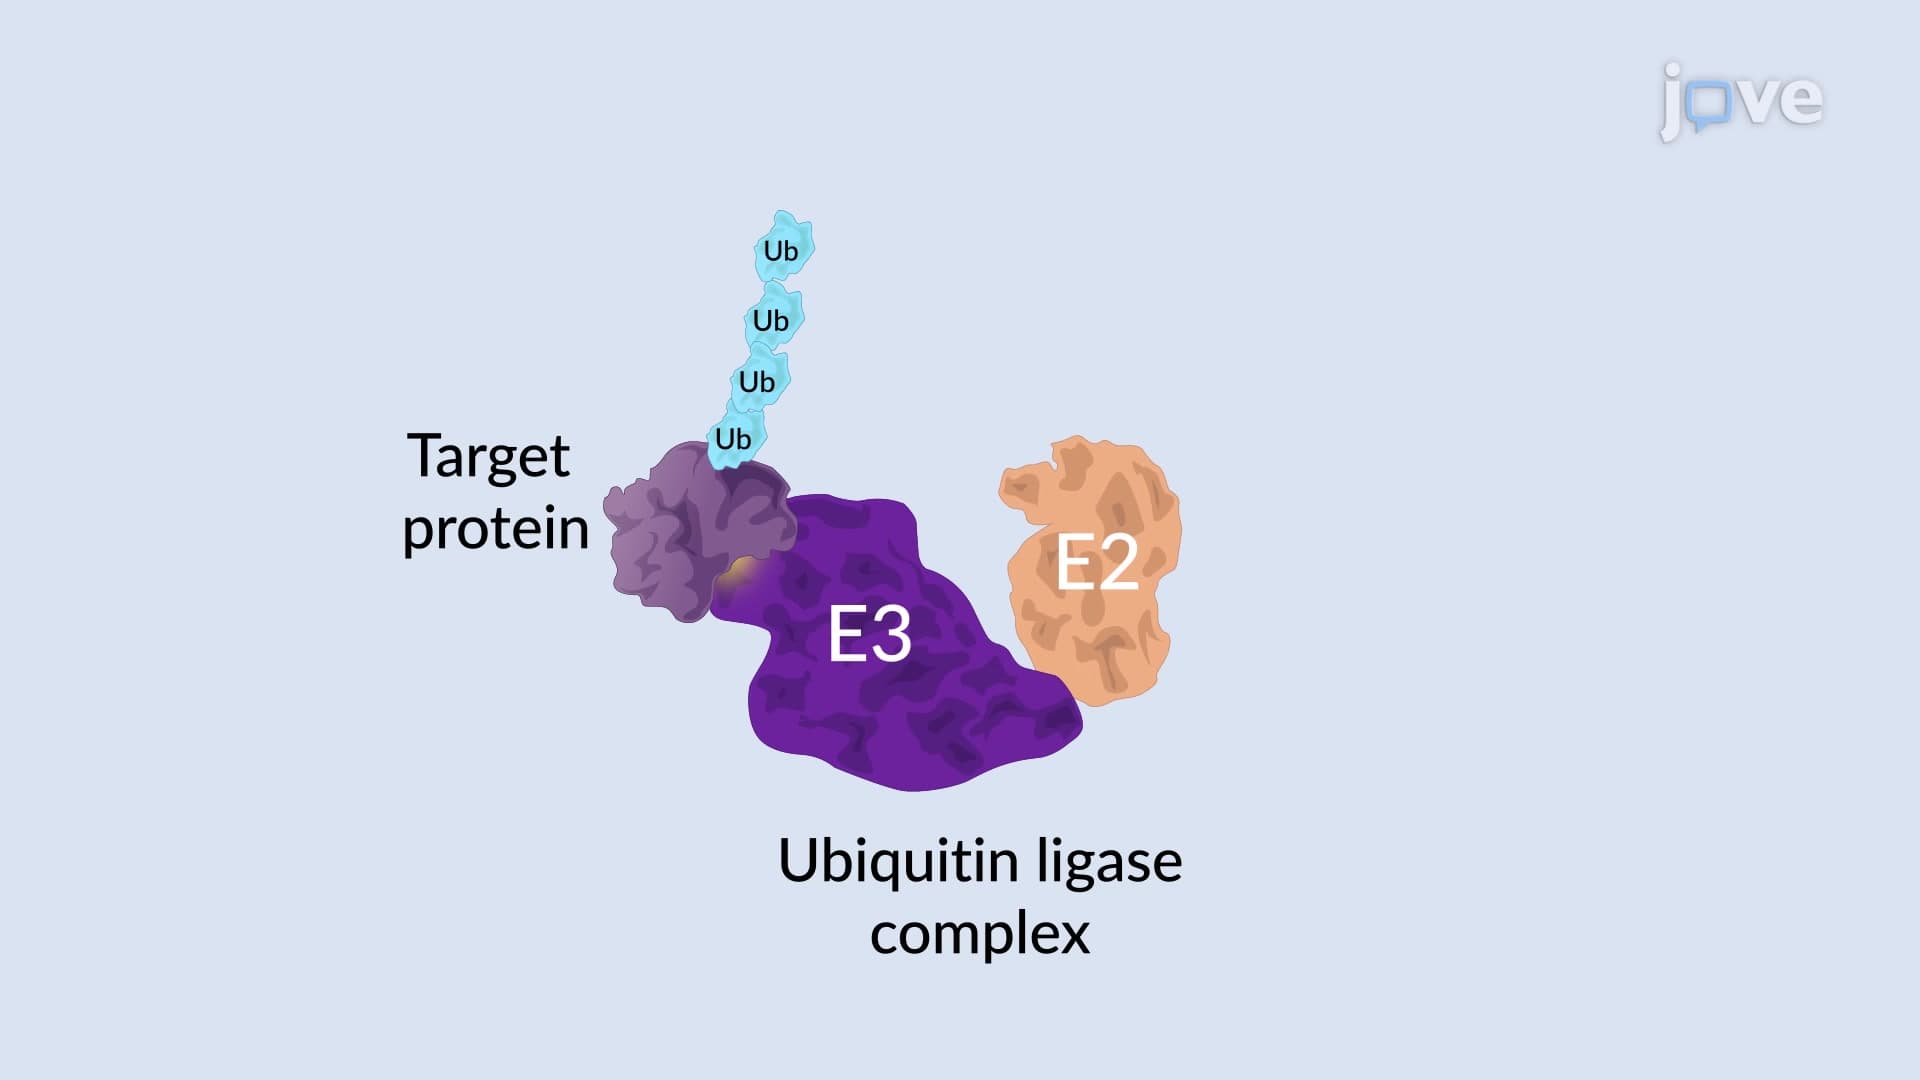
In this pathway, the target proteins are first tagged with small proteins called ubiquitin. This involves participation of a series of enzymes including— E1 (ubiquitin-activating enzyme), E2 (ubiquitin-conjugating enzyme), and E3 (ubiquitin...
 02:18
The Proteasome
In this pathway, the target proteins are first tagged with small proteins called ubiquitin. A series of enzymes carry out the ubiquitination of the target proteins - E1 (ubiquitin-activating enzyme), E2 (ubiquitin-conjugating enzyme), and E3...
 02:04
Covalently Linked Protein Regulators
These groups modify specific amino acids in a protein.
 01:27
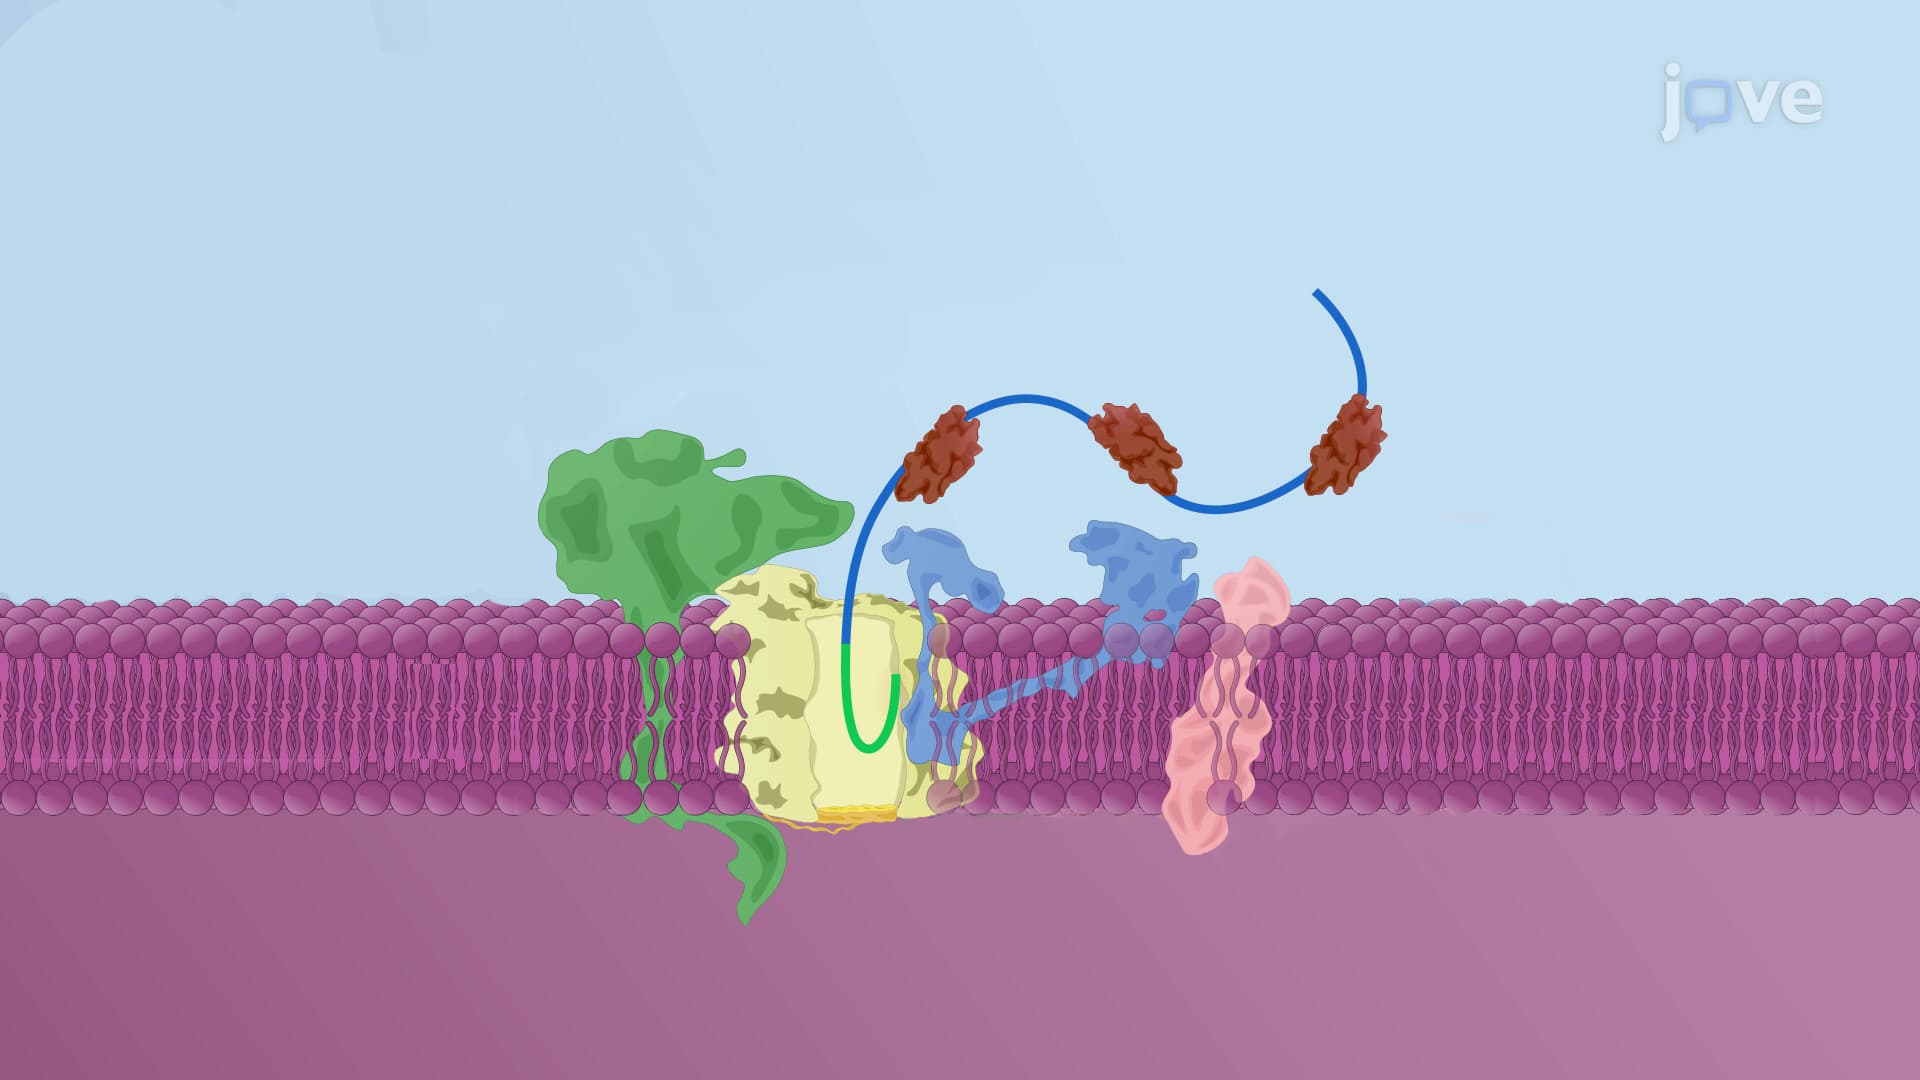
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...