Related Experiment Video
Updated: May 20, 2026
Growth-based Determination and Biochemical Confirmation of Genetic Requirements for Protein Degradation in Saccharomyces cerevisiae
Published on: February 16, 2015
Cytosolic entry of Shiga-like toxin a chain from the yeast endoplasmic reticulum requires catalytically active Hrd1p
Shuyu Li1, Robert A Spooner, Randolph Y Hampton
1School of Life Sciences, University of Warwick, Coventry, United Kingdom.

Background:
Escherichia coli Shiga-like toxin 1 normally traffics to the endoplasmic reticulum (ER) in sensitive mammalian cells from where the catalytic A chain (SLTxA1) dislocates to the cytosol to inactivate ribosomes. Currently, no molecular details of the dislocation process are available. To investigate the mechanism of the dislocation step we expressed SLTxA1 in the ER of Saccharomyces cerevisiae.
Methodology And Principal Findings:
Using a combination of growth studies and biochemical tracking in yeast knock-out strains we show that SLTxA1 follows an ER-associated degradation (ERAD) pathway to enter the cytosol in a step mediated by the transmembrane Hrd1p ubiquitin ligase complex. ER-to-cytosol dislocation of the bulk population of SLTxA1 requires Cdc48p and its ubiquitin-handling co-factor Npl4p, and this population of toxin is terminally dispatched by proteasomal degradation. A small sub-population of SLTxA1 uncouples from this classical ERAD pathway and recovers catalytic activity in the cytosol. The pathway that leads to toxicity is also Hrd1p-dependent but, unlike that for the related ricin A chain toxin, SLTxA1 dislocation does require the catalytic cysteine of Hrd1p. However it does not depend on canonical ubiquitylation since toxin variants lacking endogenous lysyl residues also utilize this pathway, and furthermore there is no requirement for a number of Cdc48p co-factors.
Conclusions And Significance:
The fraction of SLTxA1 that disengages from the ERAD pathway thus does so upstream of Cdc48p interactions and downstream of Hrd1p interactions, in a step that possibly involves de-ubiquitylation. Mechanistically therefore, the dislocation of this toxin is quite distinct from that of conventional ERAD substrates that are normally degraded, and the toxins partially characterised to date that do not require the catalytic cysteine of the major Hrd1p component of the dislocation apparatus.
Related Concept Videos
 01:32
Export of Misfolded Proteins out of the ER
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
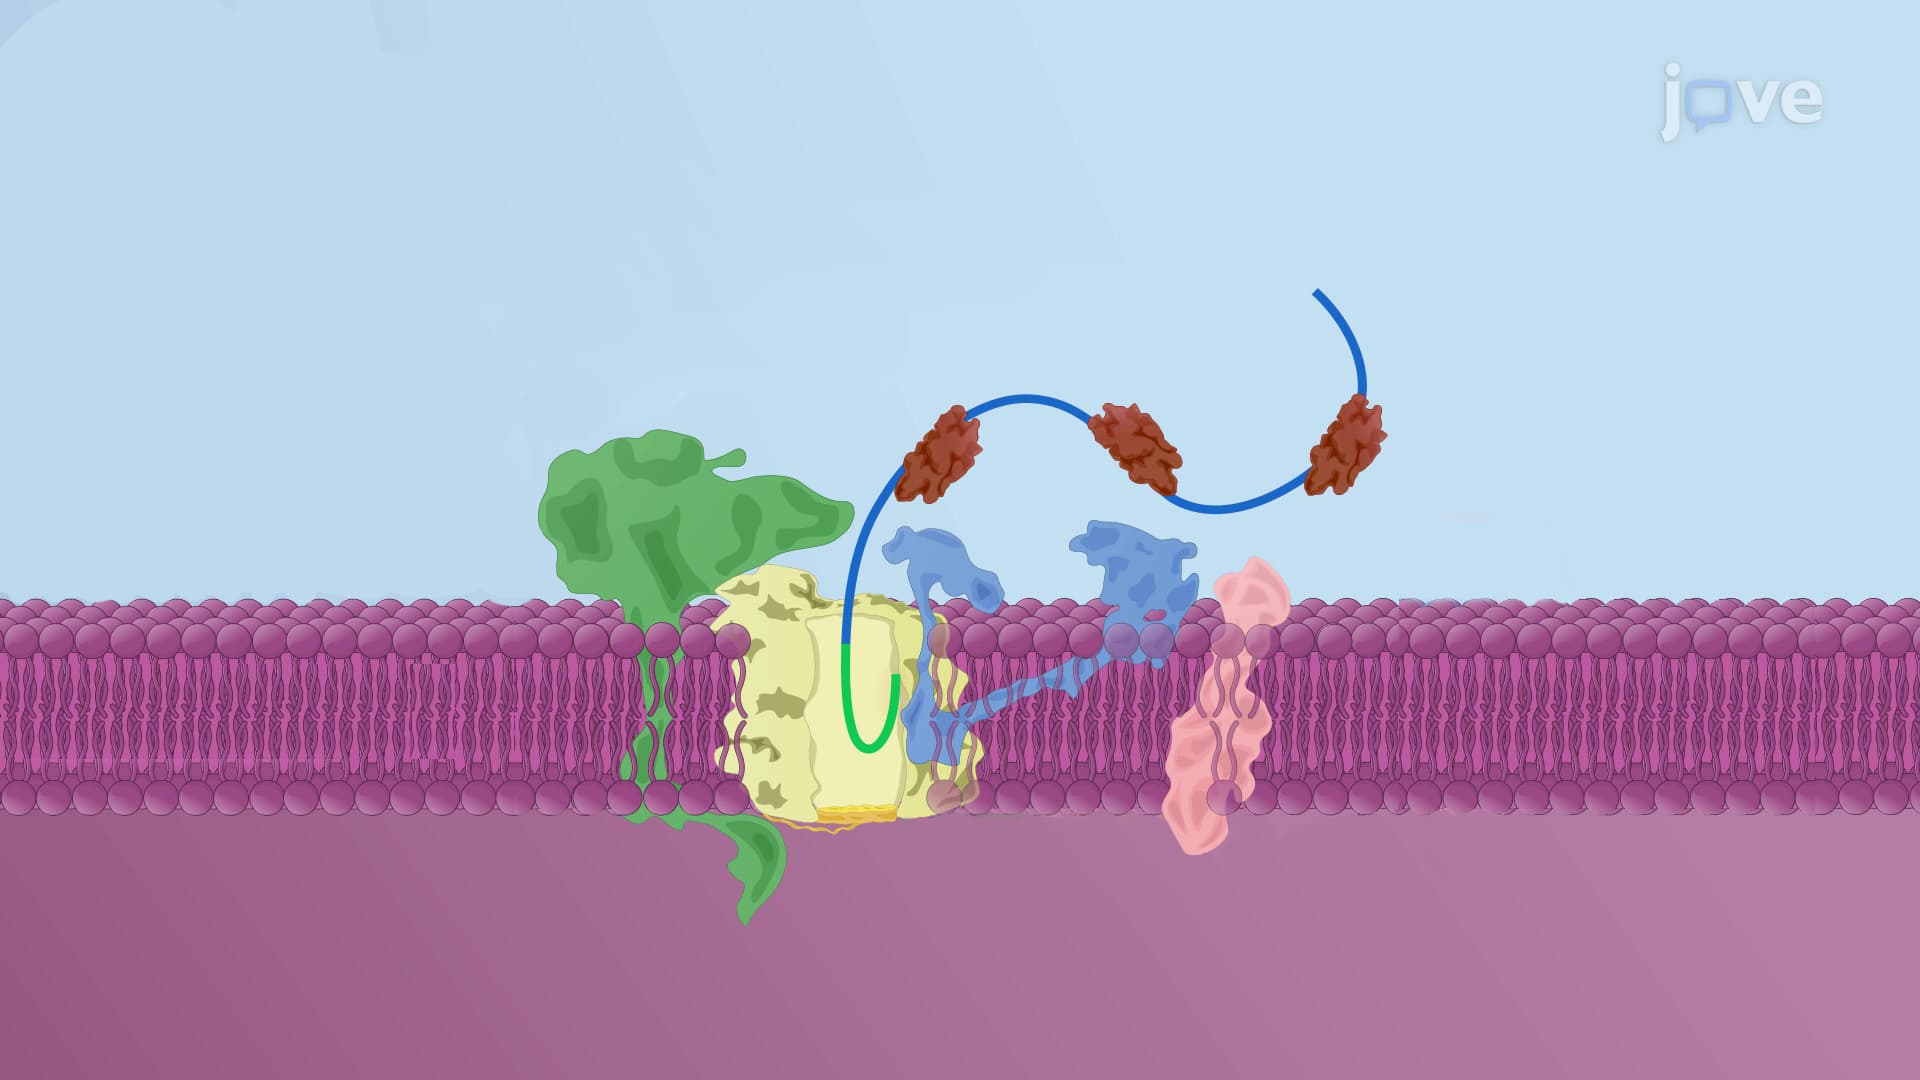
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:27
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
 01:37
Energy to Drive Translocation
Generally, polypeptides are unfolded by two distinct...
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.