
Incorporation of cis- and trans-4,5-difluoromethanoprolines into polypeptides
Vladimir S Kubyshkin1, Pavel K Mykhailiuk, Sergii Afonin
1Karlsruhe Institute of Technology (KIT), Institute of Organic Chemistry and CFN, Fritz-Haber-Weg 6, 76131 Karlsruhe, Germany.

Abstract:
Substituted prolines exert diverse effects on the backbone conformation of proteins. Novel difluoro-analogues were obtained by adding difluorocarbene to N-Boc-4,5-dehydroproline methyl ester, which gave the trans-adduct as the sole product with 71% yield. Upon cleavage of the N-protection group the free amino acid decomposed rapidly. Its incorporation into the proline-rich cell-penetrating "sweet arrow peptide" was thus accomplished using a dipeptide strategy. Two building blocks, containing either cis- or trans-4,5-difluoromethanoproline, were obtained by difluorocyclopropanation of the aminoacyl derivatives of 4,5-dehydroproline. The resulting dipeptides were stable under standard conditions of Fmoc solid phase peptide synthesis and, thus, suitable to study conformational effects.
Related Concept Videos
 01:19
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:25
Protein Folding
Protein Structure Is Critical to Its Biological Function
Proteins perform a wide range of biological functions such as catalyzing chemical reactions, providing...
 02:37
Disubstituted Cyclohexanes: cis-trans Isomerism
In cyclohexane, the substituents can occupy different positions generating distinct isomers.
 01:27
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
 01:29
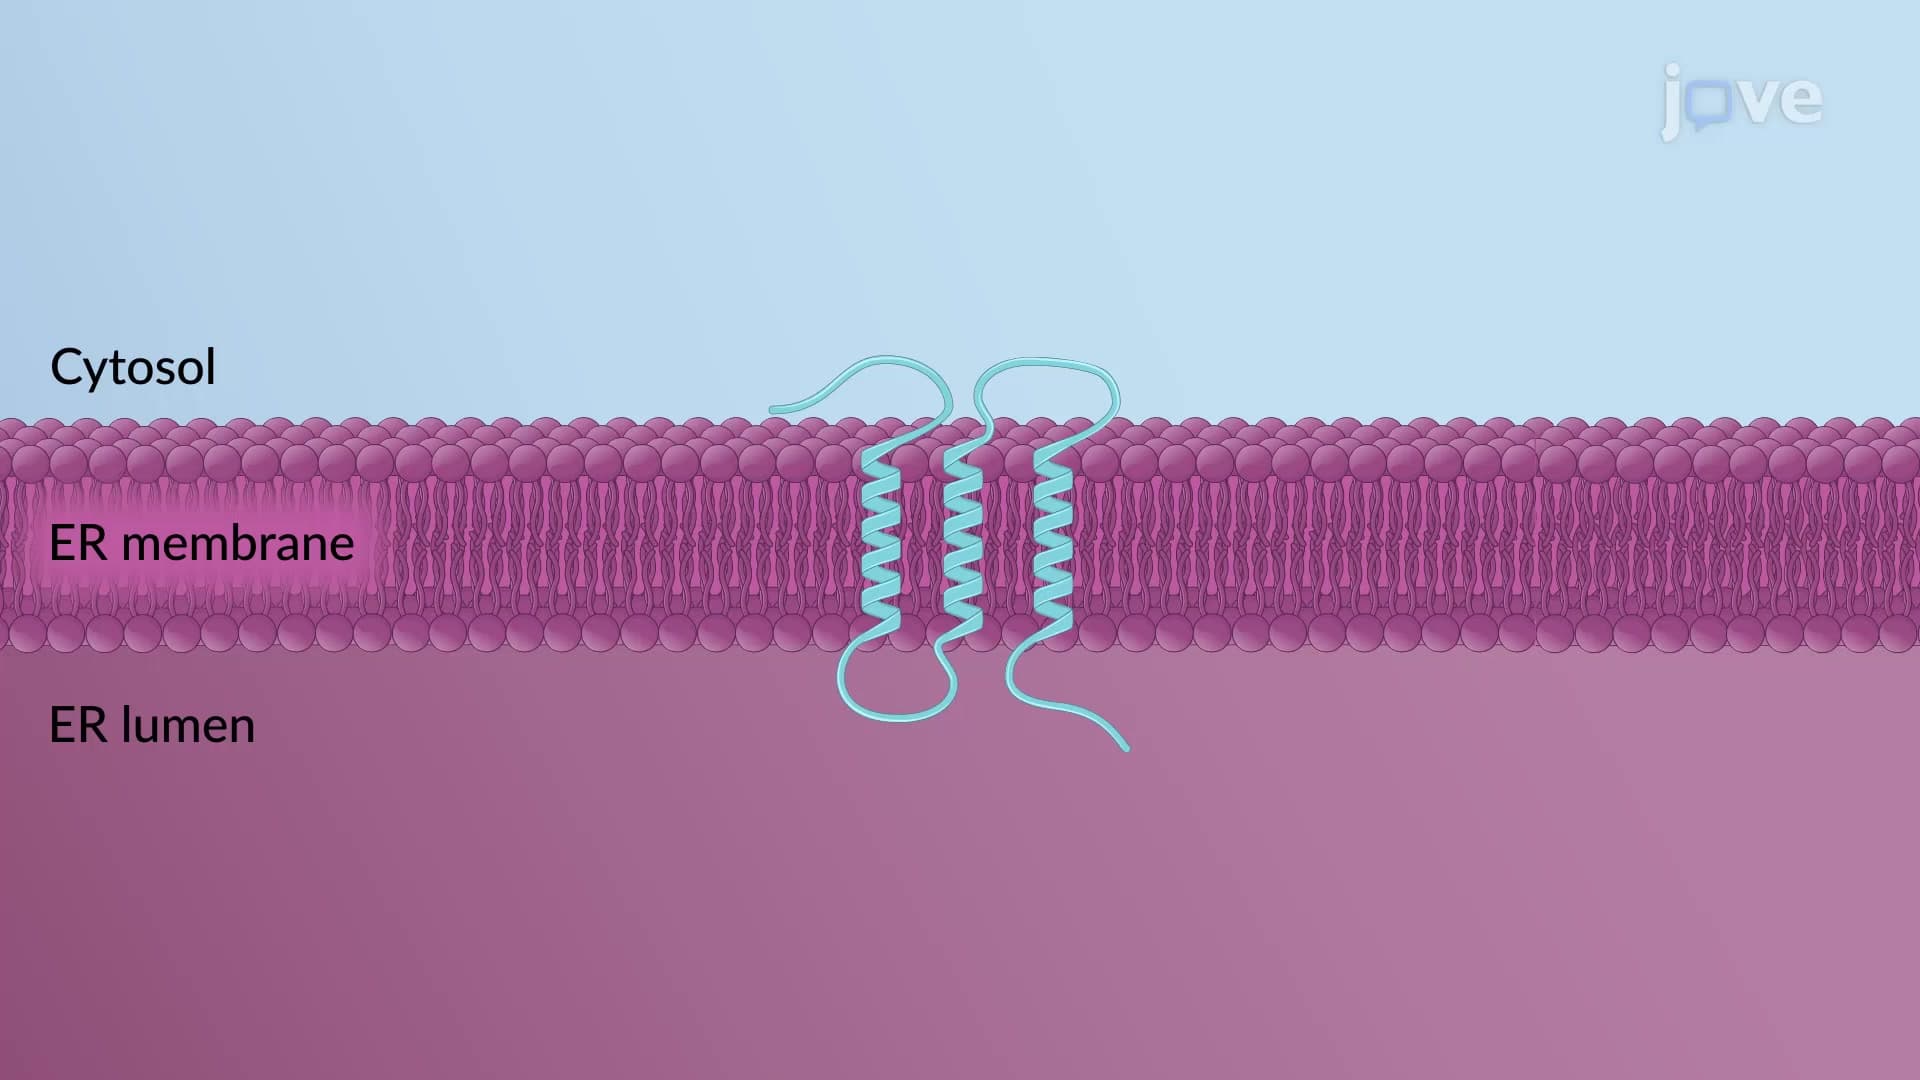
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...