Related Experiment Video
Updated: May 17, 2026

Monitoring Protein Adsorption with Solid-state Nanopores
Published on: December 2, 2011
Translocation dynamics of freely jointed Lennard-Jones chains into adsorbing pores
Christopher J Rasmussen1, Aleksey Vishnyakov, Alexander V Neimark
1Department of Chemical and Biochemical Engineering, Rutgers, The State University of New Jersey, 98 Brett Road, Piscataway, New Jersey 08854, USA.

Abstract:
Polymer translocation into adsorbing nanopores is studied by using the Fokker-Planck equation of chain diffusion along the energy landscape calculated with Monte Carlo simulations using the incremental gauge cell method. The free energy profile of a translocating chain was found by combining two independent sub-chains, one free but tethered to a hard wall, and the other tethered inside an adsorbing pore. Translocation dynamics were revealed by application of the Fokker-Planck equation for normal diffusion. Adsorption of polymer chains into nanopores involves a competition of attractive adsorption and repulsive steric hindrance contributions to the free energy. Translocation times fell into two regimes depending on the strength of the adsorbing pore. In addition, we found a non-monotonic dependence of translocation times with increasing adsorption strength, with sharp peak associated with local free energy minima along the translocation coordinate.
More Related Videos
 13:22
Adhesion Frequency Assay for In Situ Kinetics Analysis of Cross-Junctional Molecular Interactions at the Cell-Cell Interface
Published on: November 2, 2011
 07:49
Spontaneous Formation and Rearrangement of Artificial Lipid Nanotube Networks as a Bottom-Up Model for Endoplasmic Reticulum
Published on: January 22, 2019
Related Concept Videos
 01:24
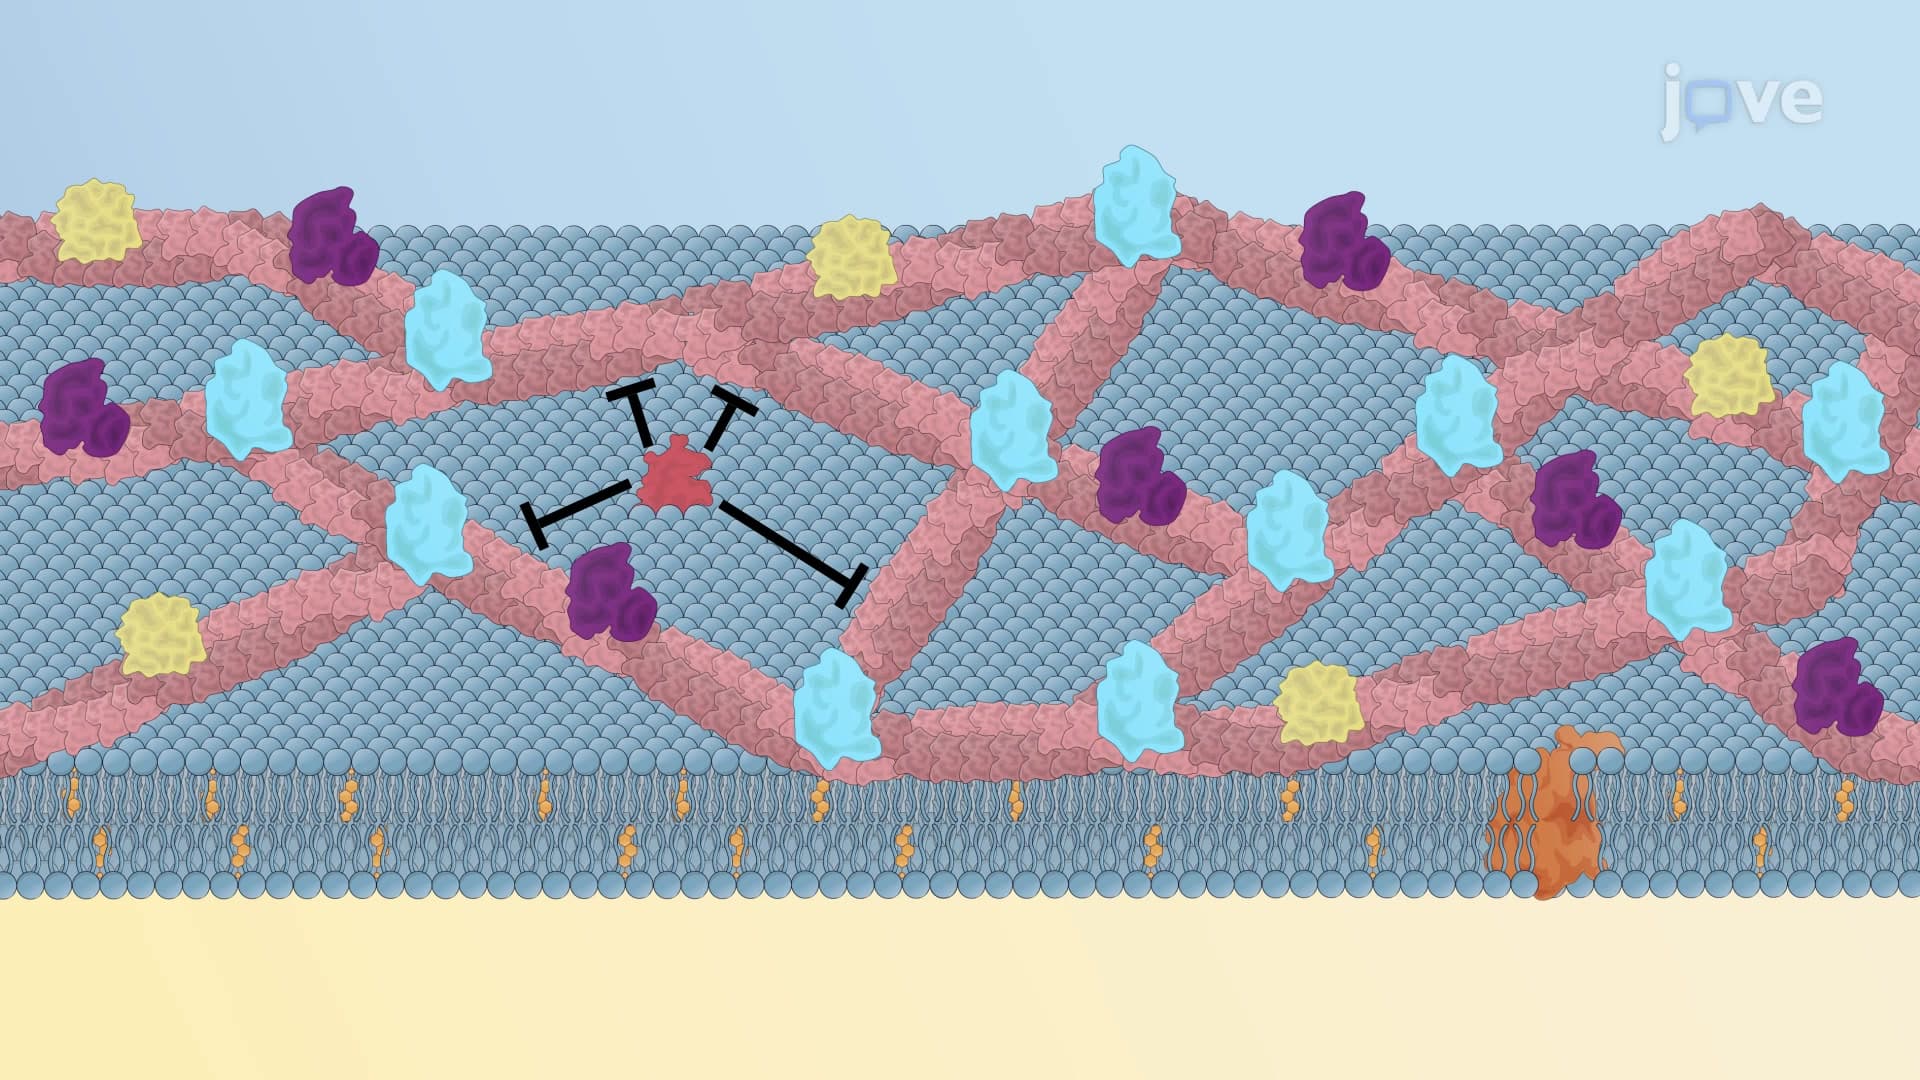
Protein Diffusion in the Membrane
 01:26
Tension Response at Adherens Junctions
α-Catenin as a Mechanosensory Protein
The α-catenin of adherens junctions is an allosteric protein with three VH (vinculin homology) domains...
 01:04
Anionic Chain-Growth Polymerization: Mechanism
 01:26
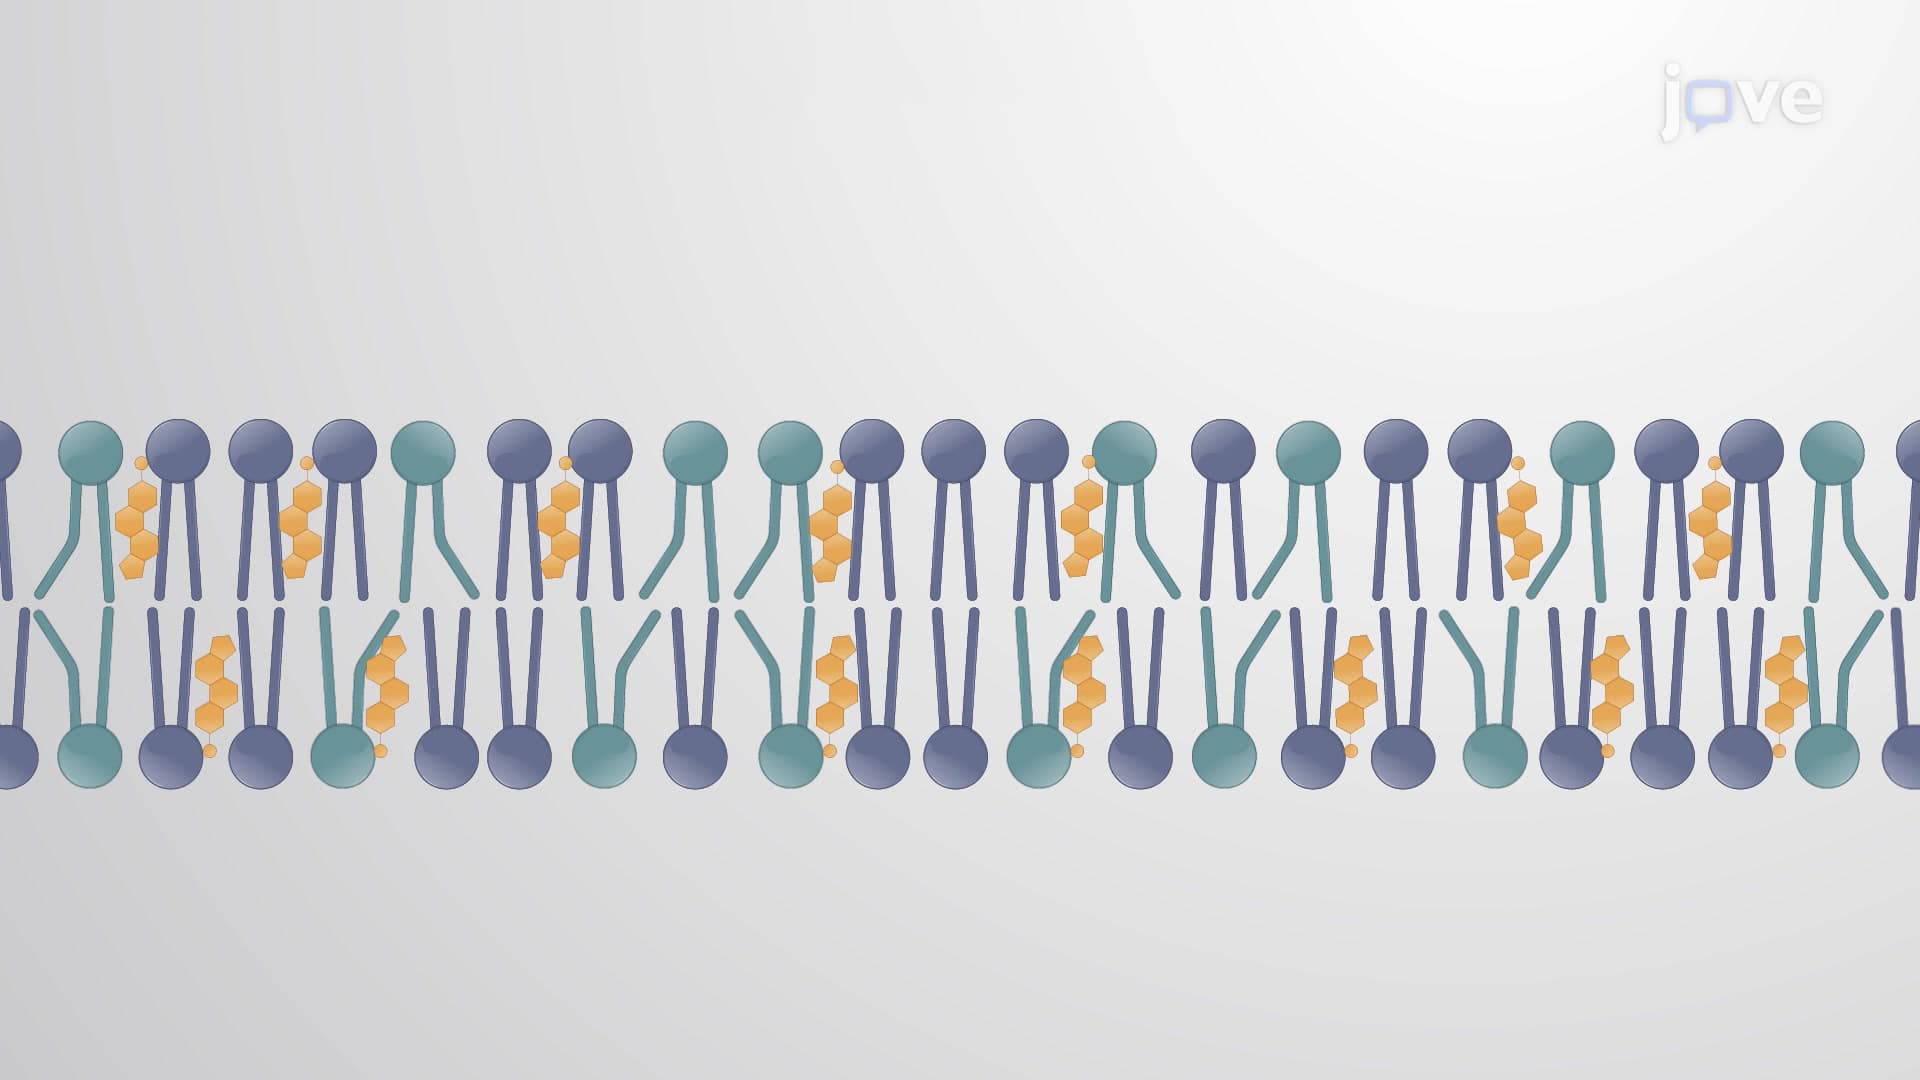
Membrane Fluidity
Mosaic nature of the membrane
The mosaic characteristic of the membrane helps the plasma membrane remain fluid. The integral proteins and lipids exist as separate but loosely-attached molecules in the membrane. The membrane is a relatively...
 00:49
Ligand Binding and Linkage
 01:27
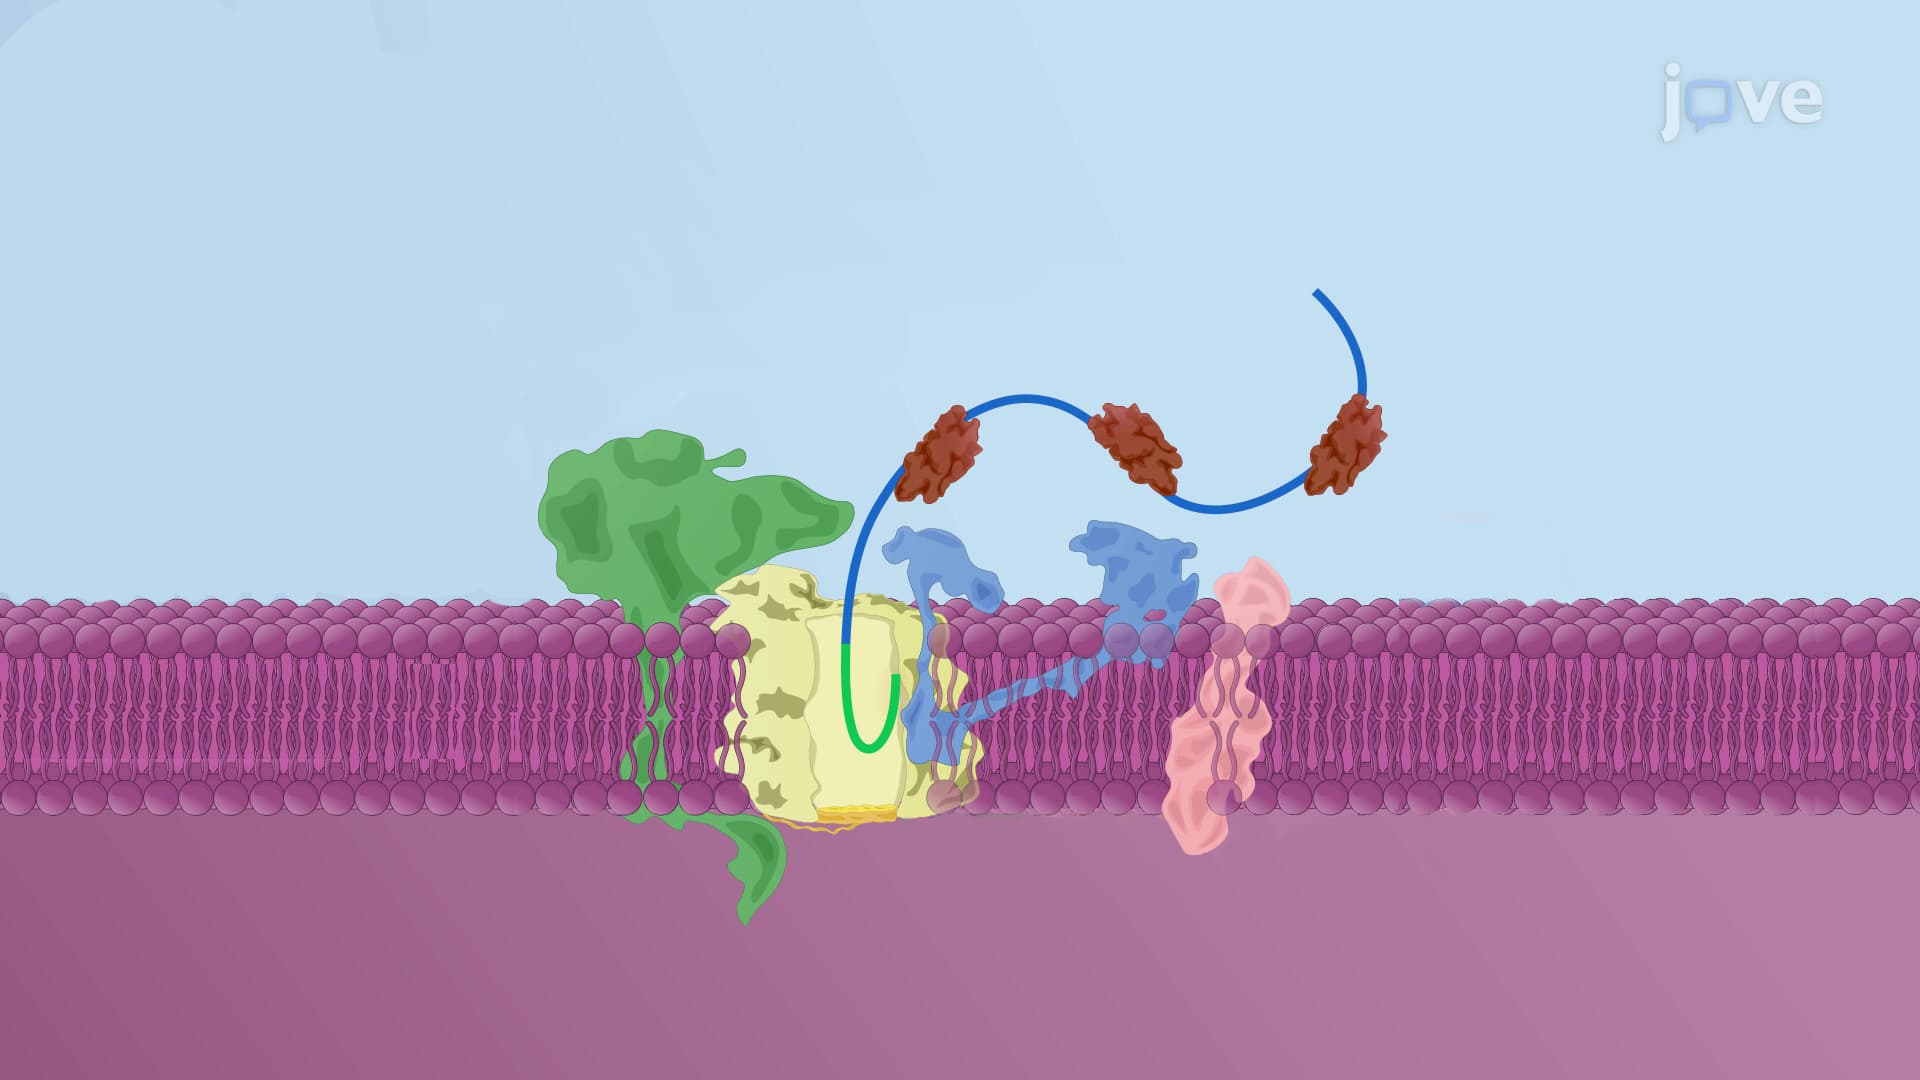
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...