Related Experiment Video
Updated: Feb 20, 2026
Lipid Bilayer Experiments with Contact Bubble Bilayers for Patch-Clampers
Published on: January 16, 2019
Exchange of Gramicidin between Lipid Bilayers: Implications for the Mechanism of Channel Formation
Kevin Lum1, Helgi I Ingólfsson1, Roger E Koeppe2
1Department of Physiology and Biophysics, Weill Cornell Medical College, New York, New York.

Abstract:
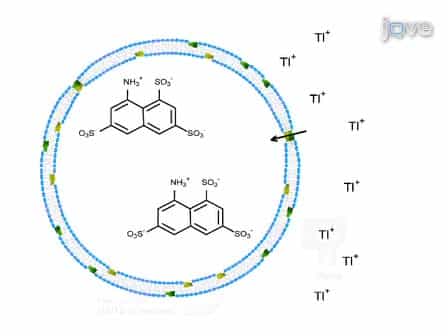
The canonical mechanism of gramicidin (gA) channel formation is transmembrane dimerization of nonconducting subunits that reside in opposite bilayer leaflets. The channels do not open and close; they appear and disappear due to subunit association and dissociation. Many different types of experiments support this monomer ↔ dimer mechanism. Recently, however, this mechanism was challenged, based on experiments with lipid vesicle-incorporated gA under conditions where vesicle fusion could be controlled. In these experiments, sustained channel activity was observed long after fusion had been terminated, which led to the proposal that gA single-channel current transitions result from closed-open transitions in long-lived bilayer-spanning dimers. This proposal is at odds with 40 years of experiments, but involves the key assumption that gA monomers do not exchange between bilayers. We tested the possibility of peptide exchange between bilayers using three different types of experiments. First, we demonstrated the exchange of gA between 1,2-dierucoyl-sn-glycero-3-phosphocholine (DC22:1PC) or 1,2-dioleoyl-sn-glycero-3-phosphocholine (DC18:1PC) lipid vesicles using a fluorescence assay for gA channel activity. Second, we added gA-free DC22:1PC vesicles to both sides of planar DC18:1PC bilayers preincubated with gA, which reduced channel activity up to 10-fold. Third, we added gA-containing DC22:1PC vesicles to one or both sides of DC18:1PC planar bilayers, which produced much higher channel activity when the gA-containing vesicles were added to both sides of the bilayer, as compared to one side only. All three types of experiments show that gA subunits can exchange between lipid bilayers. The exchange of subunits between bilayers thus is firmly established, which becomes a crucial consideration with respect to the mechanism of channel formation.
Related Concept Videos
 01:30
Ligand-Gated Ion Channel Receptor: Gating Mechanism
 01:17
Pore Transport and Ion-Pair Transport
Pore transport, also known as convective transport, is a process where small molecules like urea, water, and sugars rapidly cross cell membranes as though there were channels or pores in the membrane. Although direct microscopic evidence is limited but the concept of pores or channels is widely accepted based on physiological evidence. Despite the lack of direct...
 01:09
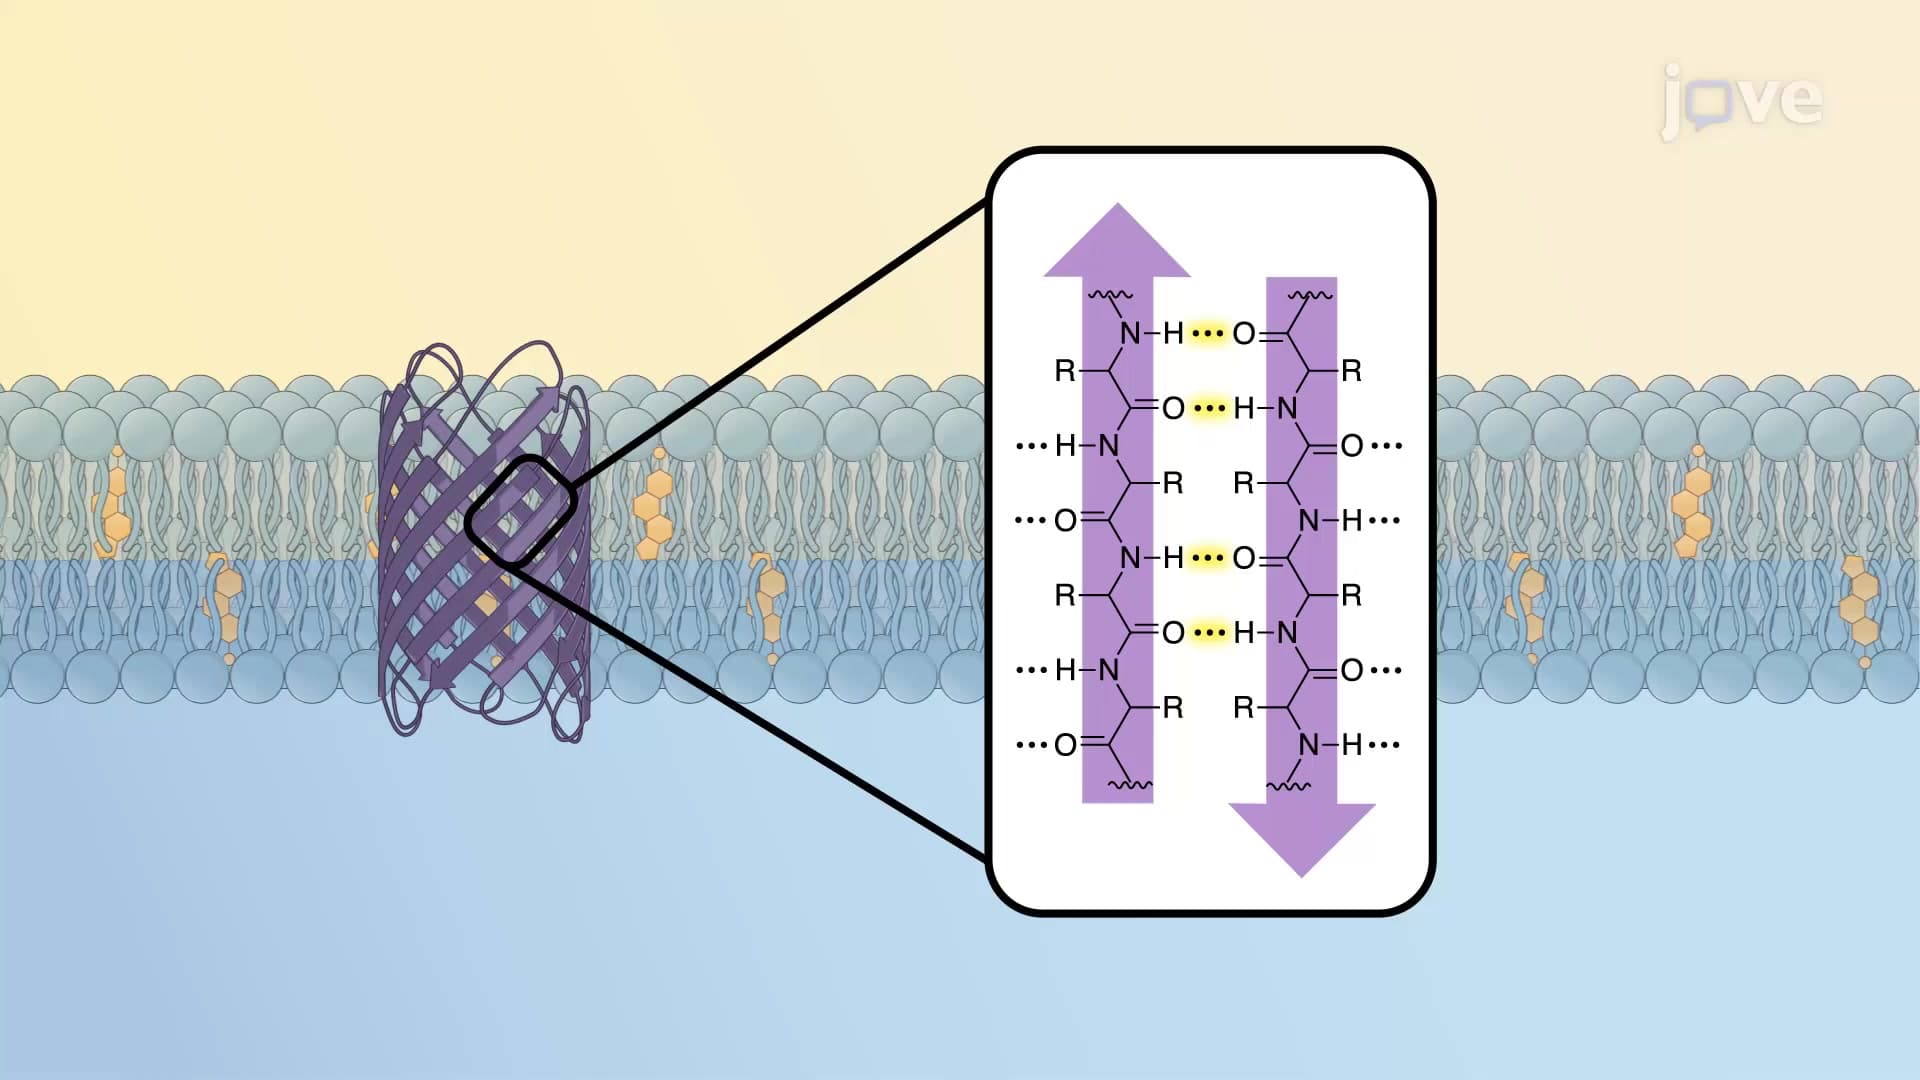
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as...
 01:19
Ligand-gated Ion Channels
Three Subfamilies of Ligand-gated Ion Channels
Ligand-gated ion channels fall into three subfamilies. The 'Cys-loop' includes the nicotinic acetylcholine receptors, γ-aminobutyric acid (GABA), glycine, and 5-hydroxytryptamine receptors. The second one is the 'Pore-loop' channels that...
 01:21
Electrochemical Gradient and Channel Proteins: An Overview
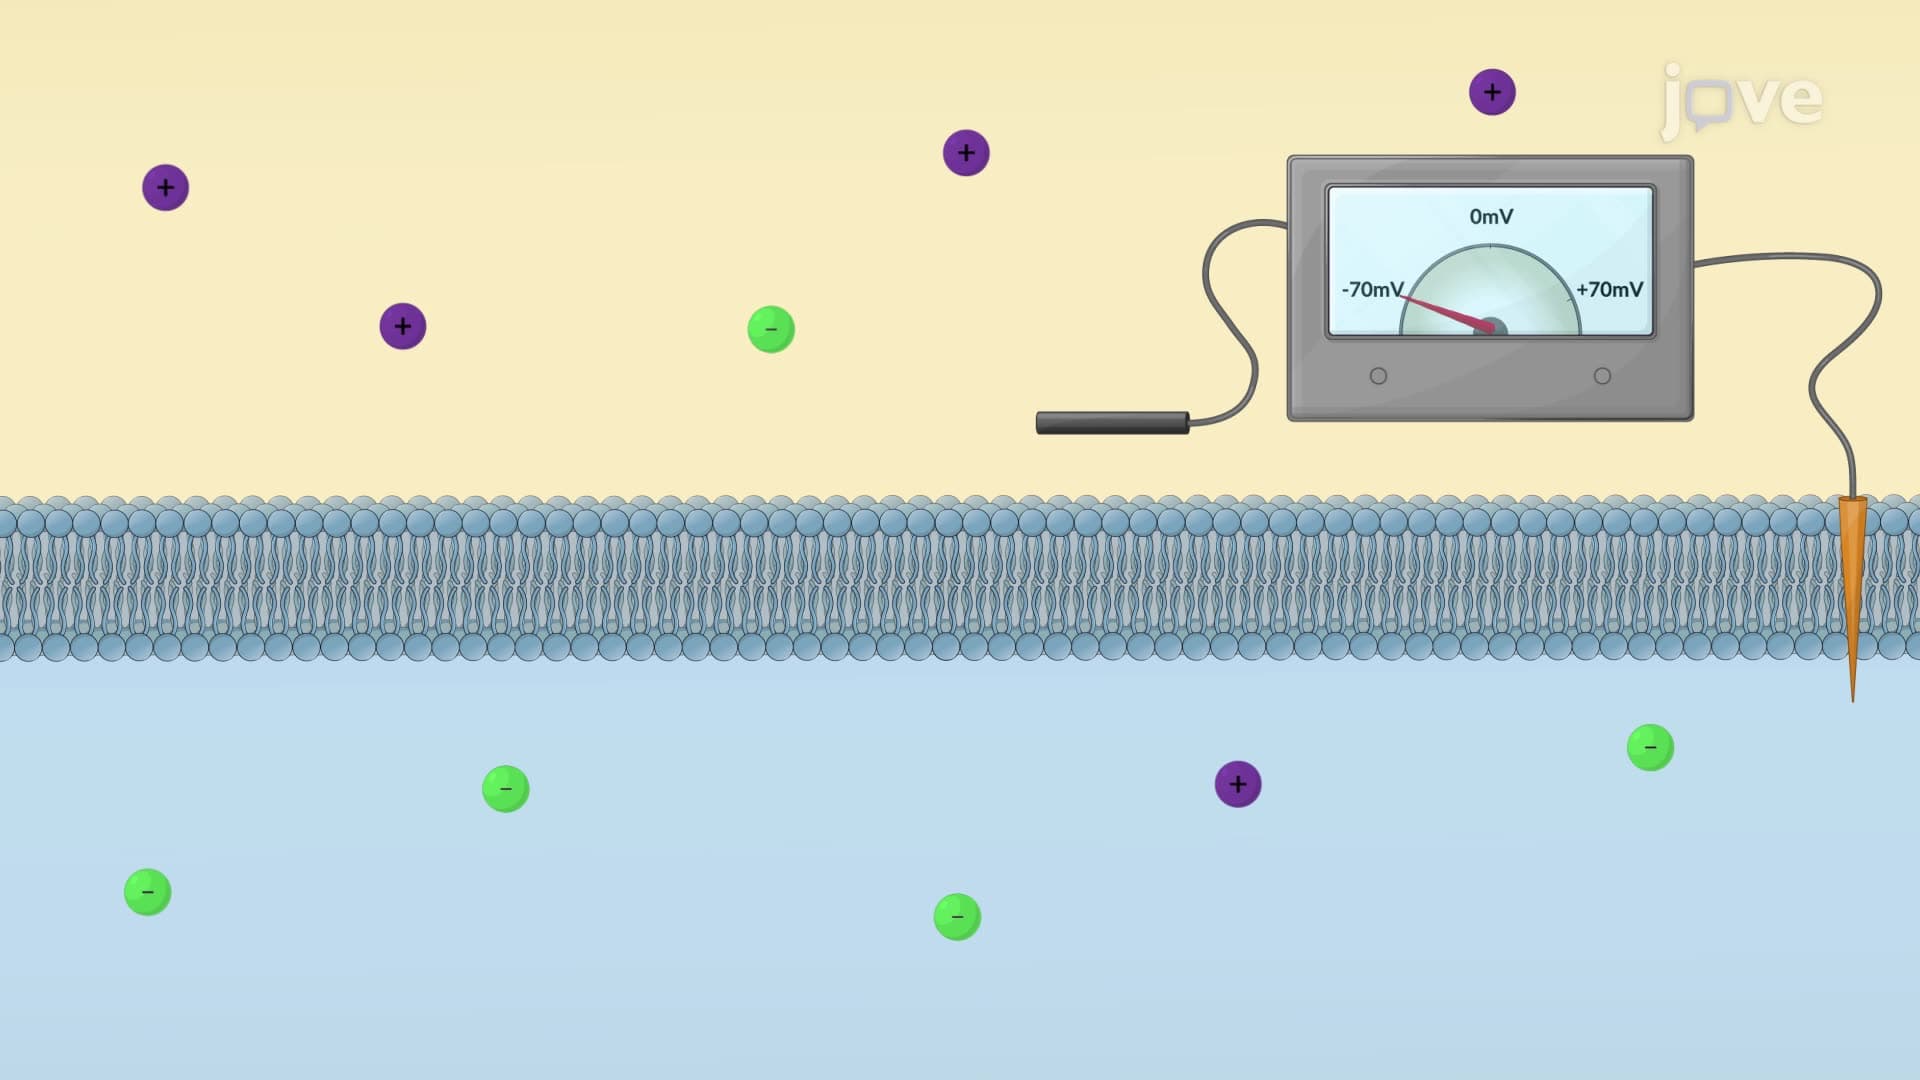
The electrical gradient: The electrical gradient across cell membranes refers to the difference in electric charge between the inside and outside of a cell. This difference drives the movement of ions towards or away from the cells. For instance, if the inside of the cell is more negatively charged relative to...
 01:19
Ion Channels
Ion channels are specialized integral membrane proteins on the plasma membrane that allow...