Related Experiment Video
Updated: Jan 23, 2026

Molecular Entanglement and Electrospinnability of Biopolymers
Published on: September 3, 2014
Cofilin drives rapid turnover and fluidization of entangled F-actin
Patrick M McCall1,2, Frederick C MacKintosh3,4, David R Kovar5,6
1Department of Physics, The University of Chicago, Chicago, IL 60637.

Abstract:
The shape of most animal cells is controlled by the actin cortex, a thin network of dynamic actin filaments (F-actin) situated just beneath the plasma membrane. The cortex is held far from equilibrium by both active stresses and polymer turnover: Molecular motors drive deformations required for cell morphogenesis, while actin-filament disassembly dynamics relax stress and facilitate cortical remodeling. While many aspects of actin-cortex mechanics are well characterized, a mechanistic understanding of how nonequilibrium actin turnover contributes to stress relaxation is still lacking. To address this, we developed a reconstituted in vitro system of entangled F-actin, wherein the steady-state length and turnover rate of F-actin are controlled by the actin regulatory proteins cofilin, profilin, and formin, which sever, recycle, and assemble filaments, respectively. Cofilin-mediated severing accelerates the turnover and spatial reorganization of F-actin, without significant changes to filament length. We demonstrate that cofilin-mediated severing is a single-timescale mode of stress relaxation that tunes the low-frequency viscosity over two orders of magnitude. These findings serve as the foundation for understanding the mechanics of more physiological F-actin networks with turnover and inform an updated microscopic model of single-filament turnover. They also demonstrate that polymer activity, in the form of ATP hydrolysis on F-actin coupled to nucleotide-dependent cofilin binding, is sufficient to generate a form of active matter wherein asymmetric filament disassembly preserves filament number despite sustained severing.
Related Concept Videos
 01:18
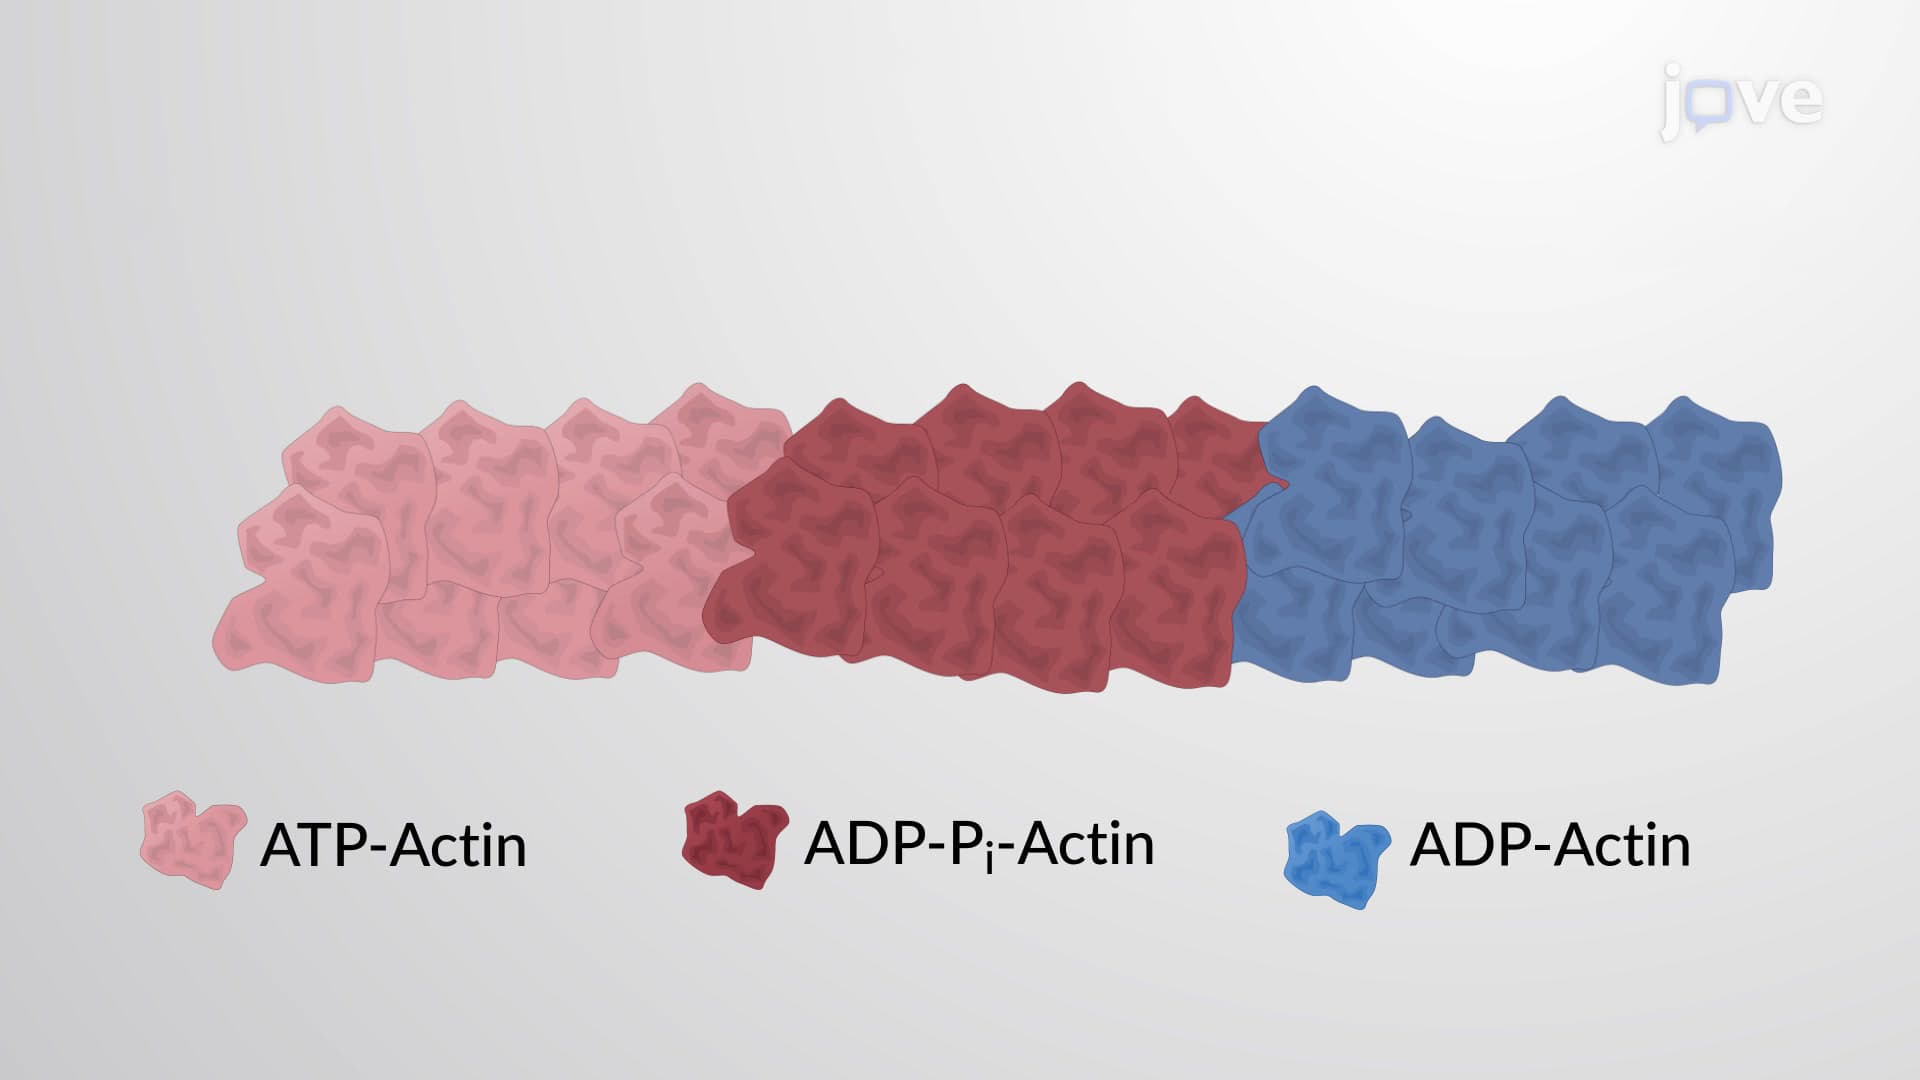
Actin Treadmilling
 01:37
Energy to Drive Translocation
Generally, polypeptides are unfolded by two distinct...
 01:19
Turnover Number and Catalytic Efficiency
Chymotrypsin is a pancreatic enzyme that breaks down proteins during digestion....
 02:15
M-Cdk Drives Transition Into Mitosis
Cyclin-dependent kinases, or Cdks, work in concert with cyclins to control cell cycle transitions. M-Cdk, a complex of Cdk1 bound to M cyclin, is a well-known example of this coordinated control that drives the transition from the G2 to the M phase.
M cyclin...
 01:26
Introduction to Actin
 01:42
Actin Polymerization
The nucleation phase involves forming a stable nucleus consisting of three actin monomers to form a new actin filament. Actin-binding proteins such as formins and Arp2/3 complex help filament growth post-nucleation. The Formins form straight...