Mud binds the kinesin-14 Ncd in Drosophila
Related Experiment Video
Updated: Nov 4, 2025
Isolation and Purification of Kinesin from Drosophila Embryos
Published on: April 27, 2012
Vincent Cutillas1, Christopher A Johnston1
1Department of Biology, University of New Mexico, Albuquerque, NM, USA.

Abstract:
Maintenance of proper mitotic spindle structure is necessary for error-free chromosome segregation and cell division. Spindle assembly is controlled by force-generating kinesin motors that contribute to its geometry and bipolarity, and balancing motor-dependent forces between opposing kinesins is critical to the integrity of this process. Non-claret dysjunctional (Ncd), a Drosophila kinesin-14 member, crosslinks and slides microtubule minus-ends to focus spindle poles and sustain bipolarity. However, mechanisms that regulate Ncd activity during mitosis are underappreciated. Here, we identify Mushroom body defect (Mud), the fly ortholog of human NuMA, as a direct Ncd binding partner. We demonstrate this interaction involves a short coiled-coil domain within Mud (MudCC) binding the N-terminal, non-motor microtubule-binding domain of Ncd (NcdnMBD). We further show that the C-terminal ATPase motor domain of Ncd (NcdCTm) directly interacts with NcdnMBD as well. Mud binding competes against this self-association and also increases NcdnMBD microtubule binding in vitro. Our results describe an interaction between two spindle-associated proteins and suggest a potentially new mode of minus-end motor protein regulation at mitotic spindle poles.
Insights
Mushroom body defect (Mud) protein directly binds Non-claret dysjunctional (Ncd) kinesin, regulating its activity. This interaction influences microtubule binding and self-association, potentially revealing a new mitotic spindle regulation mechanism.
Area of Science:
- Cell Biology
- Molecular Biology
- Genetics
Background:
- Proper mitotic spindle structure is crucial for accurate chromosome segregation during cell division.
- Kinesin motors, like Non-claret dysjunctional (Ncd), are essential for spindle assembly, geometry, and bipolarity.
- Regulatory mechanisms controlling Ncd activity during mitosis remain largely uncharacterized.
Purpose of the Study:
- To identify and characterize novel regulators of the kinesin-14 motor protein Ncd in *Drosophila*.
- To investigate the interaction between Ncd and its binding partner, Mushroom body defect (Mud).
- To elucidate the functional consequences of the Mud-Ncd interaction on Ncd activity and spindle organization.
Main Methods:
- Co-immunoprecipitation assays to confirm direct binding between Mud and Ncd.
- In vitro biochemical assays to map interaction domains (MudCC and NcdnMBD, NcdCTm and NcdnMBD).
- Microtubule binding assays to assess the effect of Mud on Ncd's interaction with microtubules.
Main Results:
- Mushroom body defect (Mud), the *Drosophila* ortholog of human NuMA, was identified as a direct binding partner of Ncd.
- The interaction involves Mud's coiled-coil domain (MudCC) binding Ncd's N-terminal microtubule-binding domain (NcdnMBD).
- Mud binding disrupts Ncd self-association (NcdCTm-NcdnMBD interaction) and enhances NcdnMBD microtubule binding.
Conclusions:
- A novel interaction between spindle-associated proteins Mud and Ncd has been characterized.
- Mud acts as a regulator of Ncd, modulating its self-association and microtubule binding properties.
- This study suggests a new mechanism for regulating minus-end directed motor protein activity at mitotic spindle poles.
Related Concept Videos
 01:43
The Movement of Organelles and Vesicles
 01:45
Destabilization of Microtubules
 01:32
Microtubule Associated Motor Proteins
 01:32
Pinching-off of Coated Vesicles
 01:39
Anaphase A and B
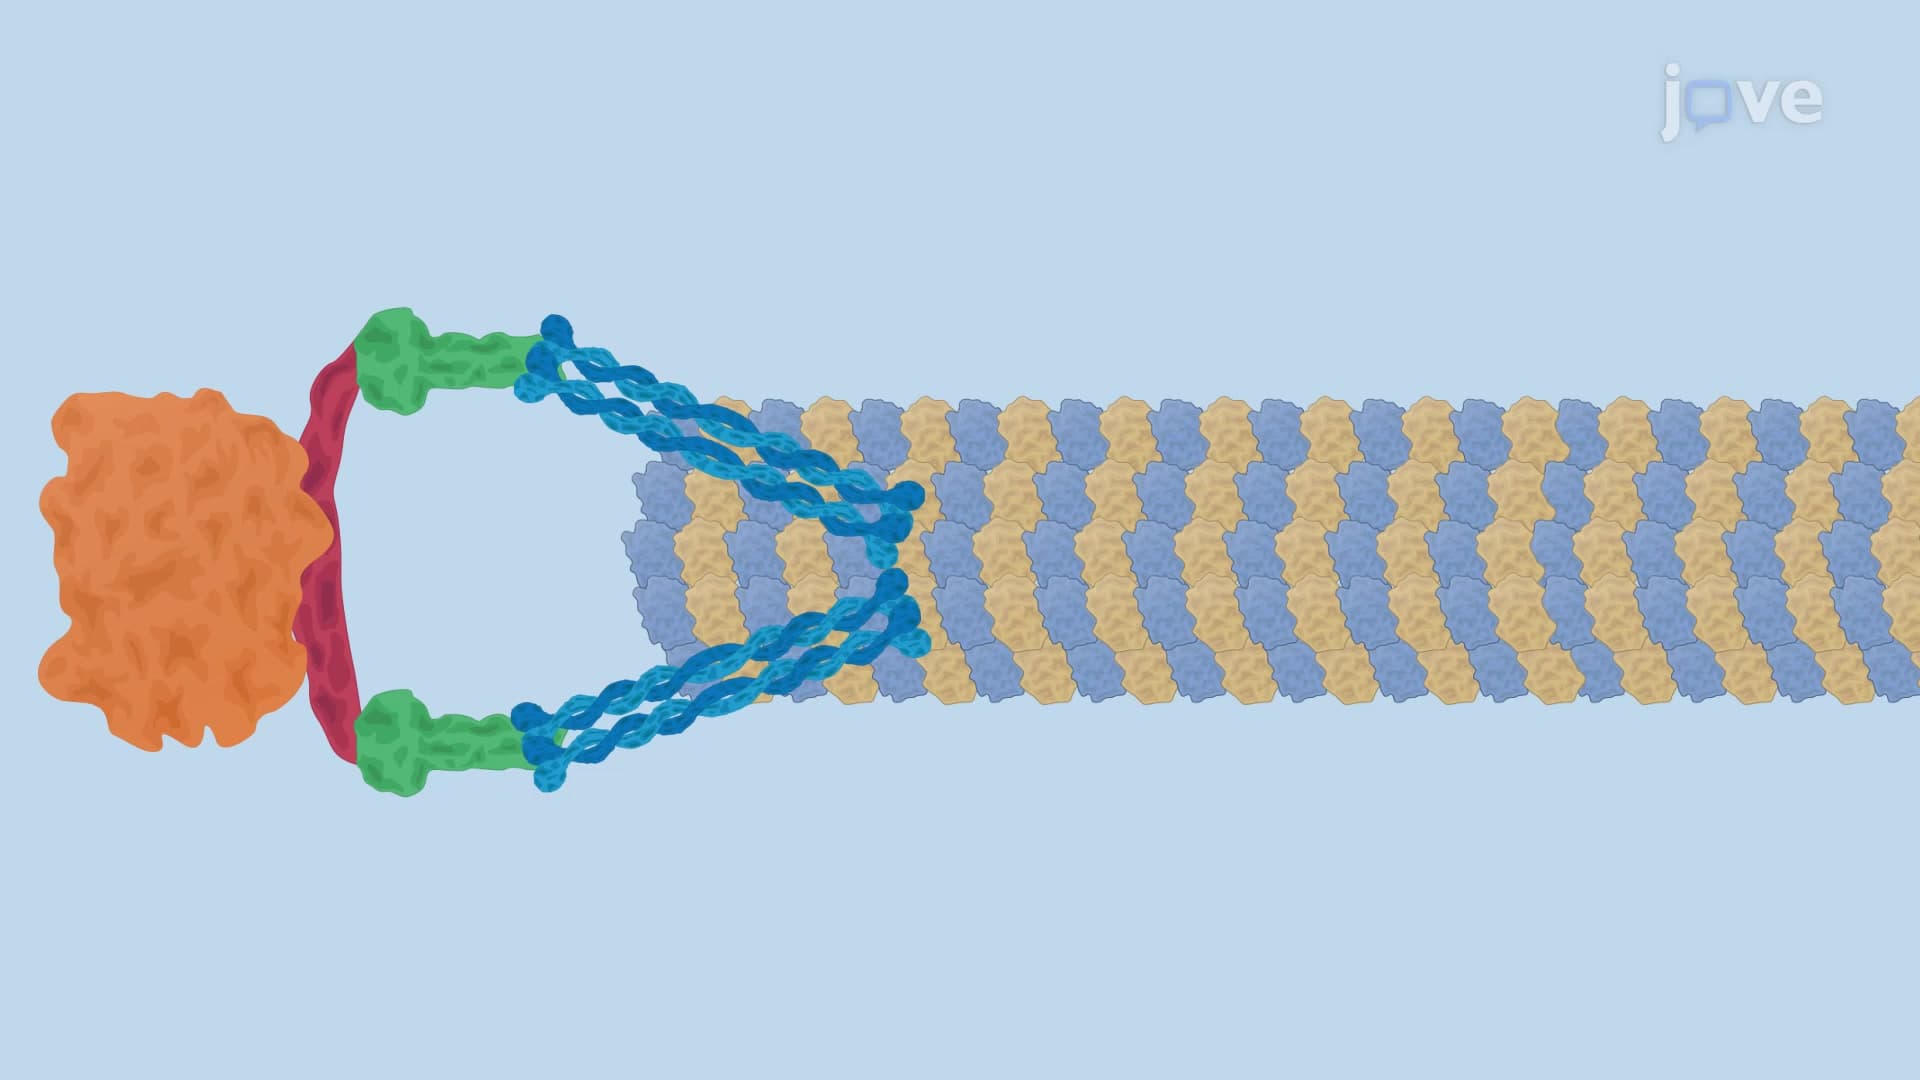
Plus-end depolymerization releases tubulin heterodimers from the terminal region of the microtubule. As tubulin subunits are lost, the Ndc80 complexes detach...
 02:57
Attachment of Sister Chromatids