Related Experiment Video
Updated: Jun 24, 2025

Membrane Remodeling of Giant Vesicles in Response to Localized Calcium Ion Gradients
Published on: July 16, 2018
Continuous Transformation from Membrane-Less Coacervates to Membranized Coacervates and Giant Vesicles: Toward
Yang Zhou1,2, Kehu Zhang1,2, Silvia Moreno1
1Leibniz-Institut für Polymerforschung Dresden e.V., Hohe Straße 6, Dresden, 01069, Germany.

Abstract:
The membranization of membrane-less coacervates paves the way for the exploitation of complex protocells with regard to structural and cell-like functional behaviors. However, the controlled transformation from membranized coacervates to vesicles remains a challenge. This can provide stable (multi)phase and (multi)compartmental architectures through the reconfiguration of coacervate droplets in the presence of (bioactive) polymers, bio(macro)molecules and/or nanoobjects. Herein, we present a continuous protocell transformation from membrane-less coacervates to membranized coacervates and, ultimately, to giant hybrid vesicles. This transformation process is orchestrated by altering the balance of non-covalent interactions through varying concentrations of an anionic terpolymer, leading to dynamic processes such as spontaneous membranization of terpolymer nanoparticles at the coacervate surface, disassembly of the coacervate phase mediated by the excess anionic charge, and the redistribution of coacervate components in membrane. The diverse protocells during the transformation course provide distinct structural features and molecular permeability. Notably, the introduction of multiphase coacervates in this continuous transformation process signifies advancements toward the creation of synthetic cells with different diffusible compartments. Our findings emphasize the highly controlled continuous structural reorganization of coacervate protocells and represents a novel step toward the development of advanced and sophisticated synthetic protocells with more precise compositions and complex (membrane) structures.
Related Concept Videos
 00:59
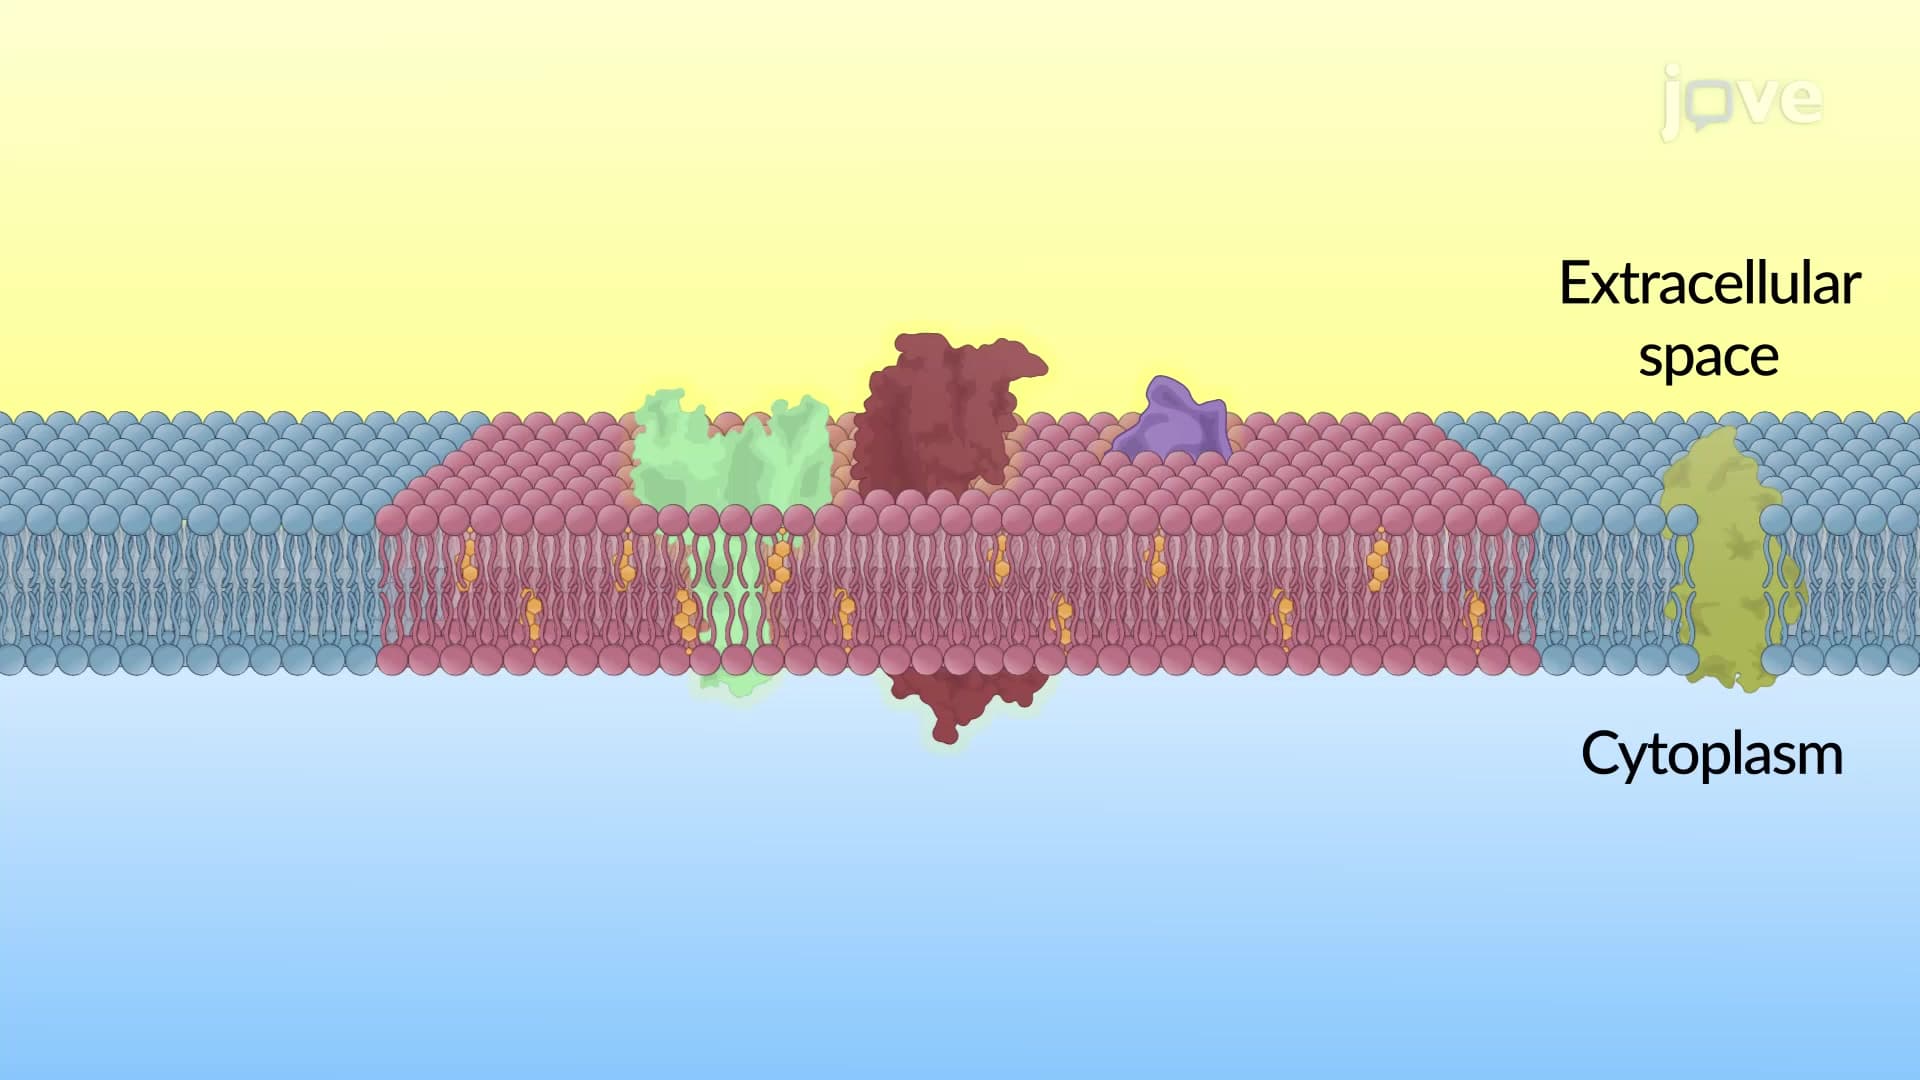
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with...
 01:12
Clathrin Coated Vesicles
 01:18
Membrane Domains
Protein Domains
The membrane comprises a group of distinct proteins responsible for carrying out a cell's specific function. For example, the plasma membrane of the human sperm, or a single germ cell, contains a unique set of proteins in the...
 01:19
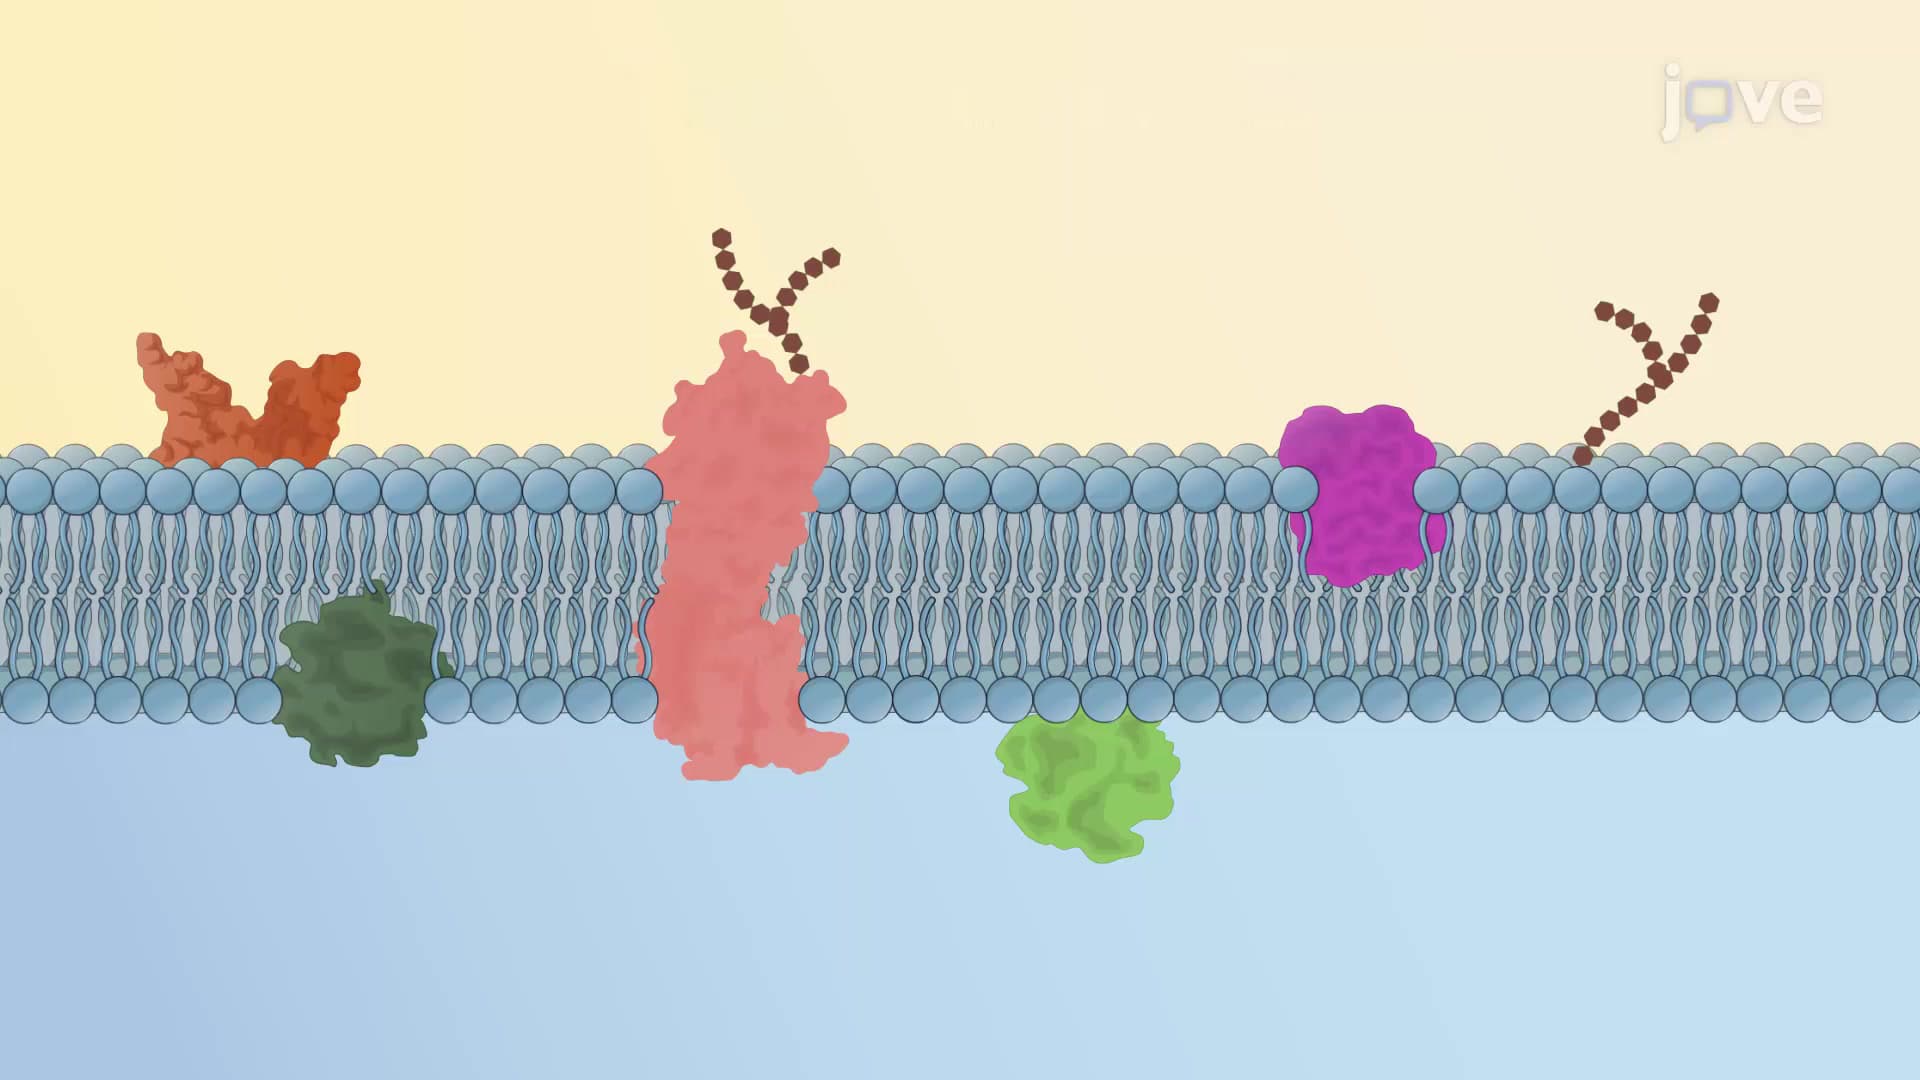
Fluid Mosaic Model
 01:26
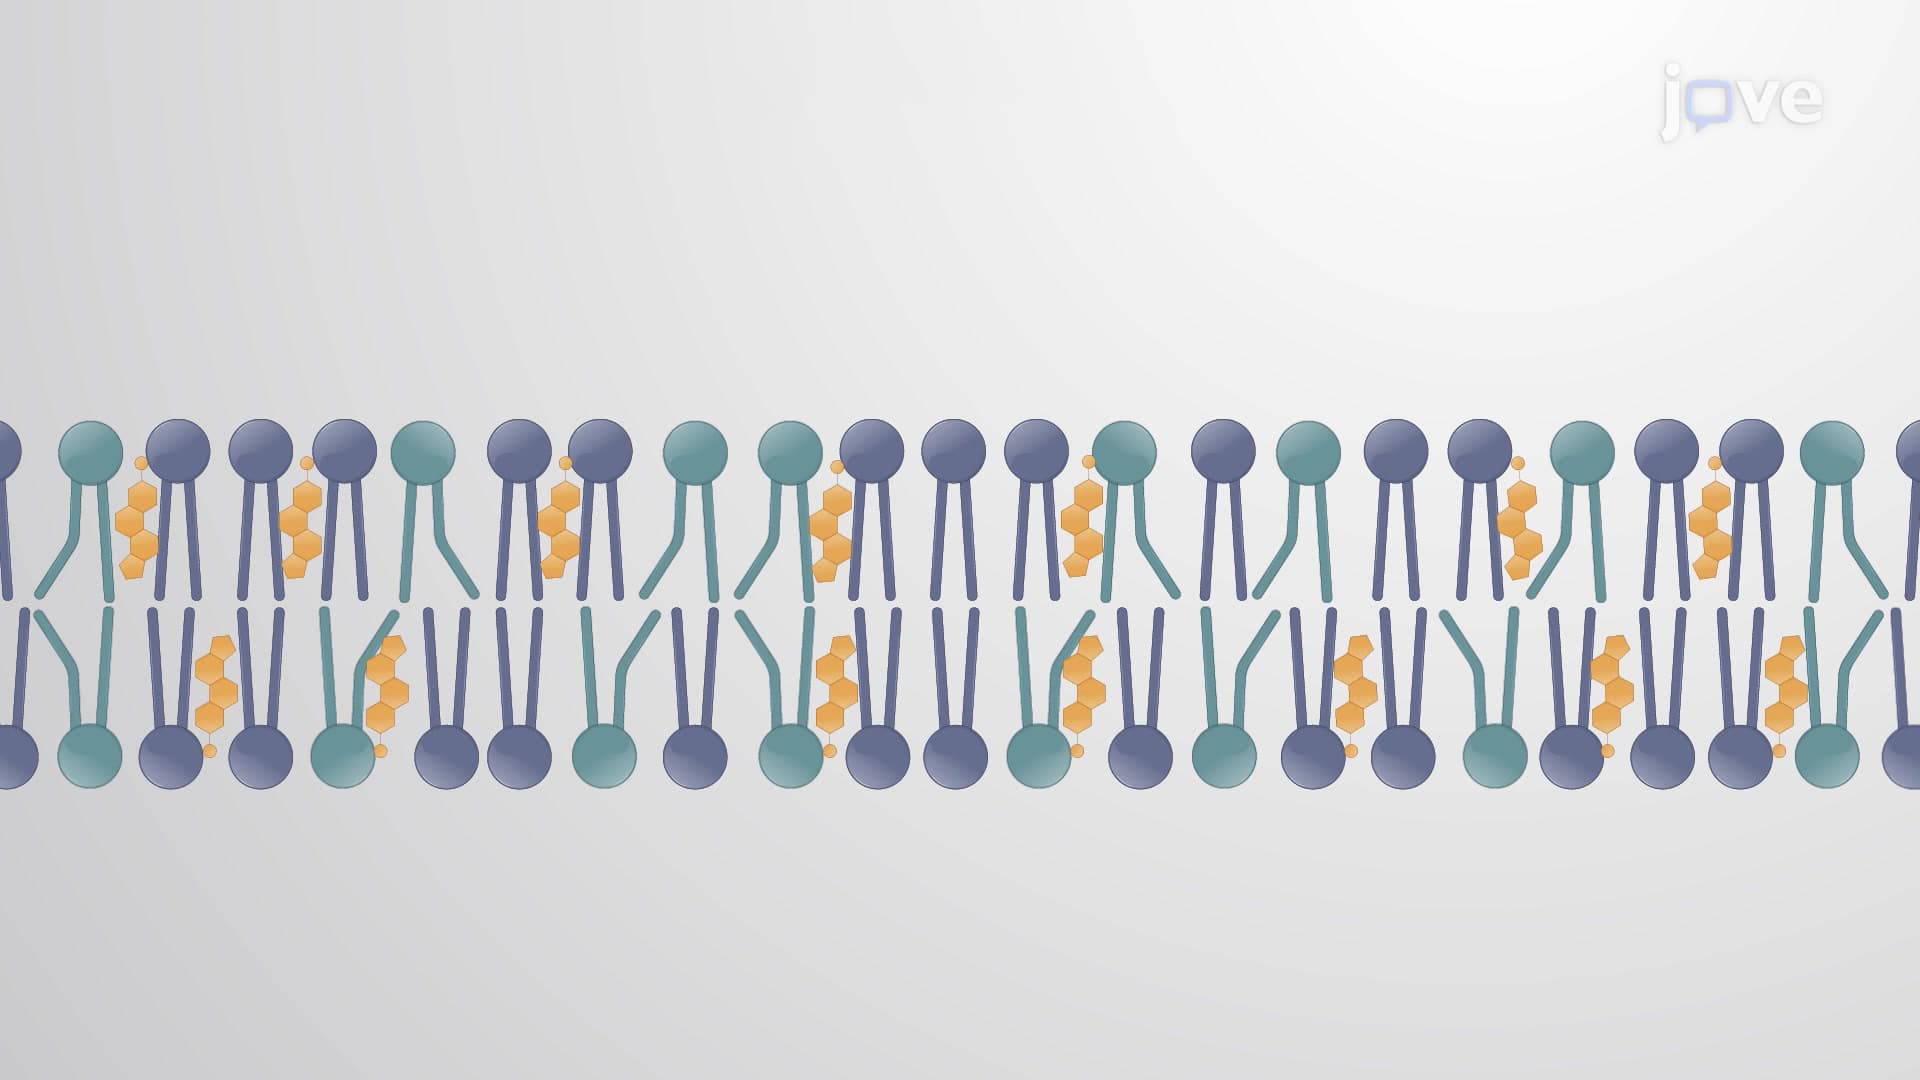
Membrane Fluidity
Mosaic nature of the membrane
The mosaic characteristic of the membrane helps the plasma membrane remain fluid. The integral proteins and lipids exist as separate but loosely-attached molecules in the membrane. The membrane is...
 01:45
Vesicular Tubular Clusters
With the help of motor proteins such...