Related Experiment Video
Updated: Apr 1, 2026
12:57

Investigating the Spreading and Toxicity of Prion-like Proteins Using the Metazoan Model Organism C. elegans
Published on: January 8, 2015
16.7K
Correction: Intracellular trafficking SNARE protein, syntaxin-6, modifies prion cellular phenotypes and risk of
Elizabeth Hill1, Mitali M Patel1, Juan M Ribes1
1MRC Prion Unit at UCL, UCL Institute of Prion Diseases, Courtauld Building, 33 Cleveland Street, London, W1W 7FF, UK.
Acta Neuropathologica
|March 30, 2026

Abstract
No abstract available in PubMed .
Related Concept Videos
 01:45
Regulation of Nuclear Protein Sorting
3.5K
Nuclear protein sorting regulates nucleus composition and gene expression, crucial for determining the fate of a eukaryotic cell. Hence, the entry and exit of molecules across the nuclear envelope is a tightly controlled process. Nuclear protein sorting can be inhibited by one of the following ways: 1) masking cargo signal sequences, 2) modifying the nuclear receptor's affinity for cargo, 3) controlling the nuclear pore size, 4) retaining the cargo during its transit to the cytosol or the...
3.5K
 01:43
SNAREs and Membrane Fusion
13.4K
Once a transport vesicle has recognized its target organelle, the vesicular membrane needs to fuse with the target membrane to unload the cargo. Transmembrane proteins called SNAREs present on organelle membranes and their vesicles, mediate vesicle fusion.
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
13.4K
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
19.4K
Proteins and neurotransmitters in secretory vesicles can be released from a cell upon vesicle docking, priming, and fusion with the plasma membrane. Vesicles are docked and primed in preparation for the quick exocytosis of their contents in response to a stimulus. The fusion process is mainly carried out by a SNAP Receptor or SNARE complex, consisting of synaptobrevin, syntaxin-1, and SNAP-25.
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
19.4K
 03:03
Amyloid Fibrils
13.0K
Amyloid fibrils are aggregates of misfolded proteins. Under most circumstances, misfolded proteins are either refolded by chaperone proteins or degraded by the proteasome. However, in the case of a mutation or a disease, these proteins can accumulate to form large clusters and often further assemble to form elongated fibers, called fibrils.
Amyloid deposits were observed as early as 1639 in the liver and the spleen. In 1854, Rudolph Virchow performed iodine staining,...
Amyloid deposits were observed as early as 1639 in the liver and the spleen. In 1854, Rudolph Virchow performed iodine staining,...
13.0K
 01:19
Translocation of Proteins into the Mitochondria
13.7K
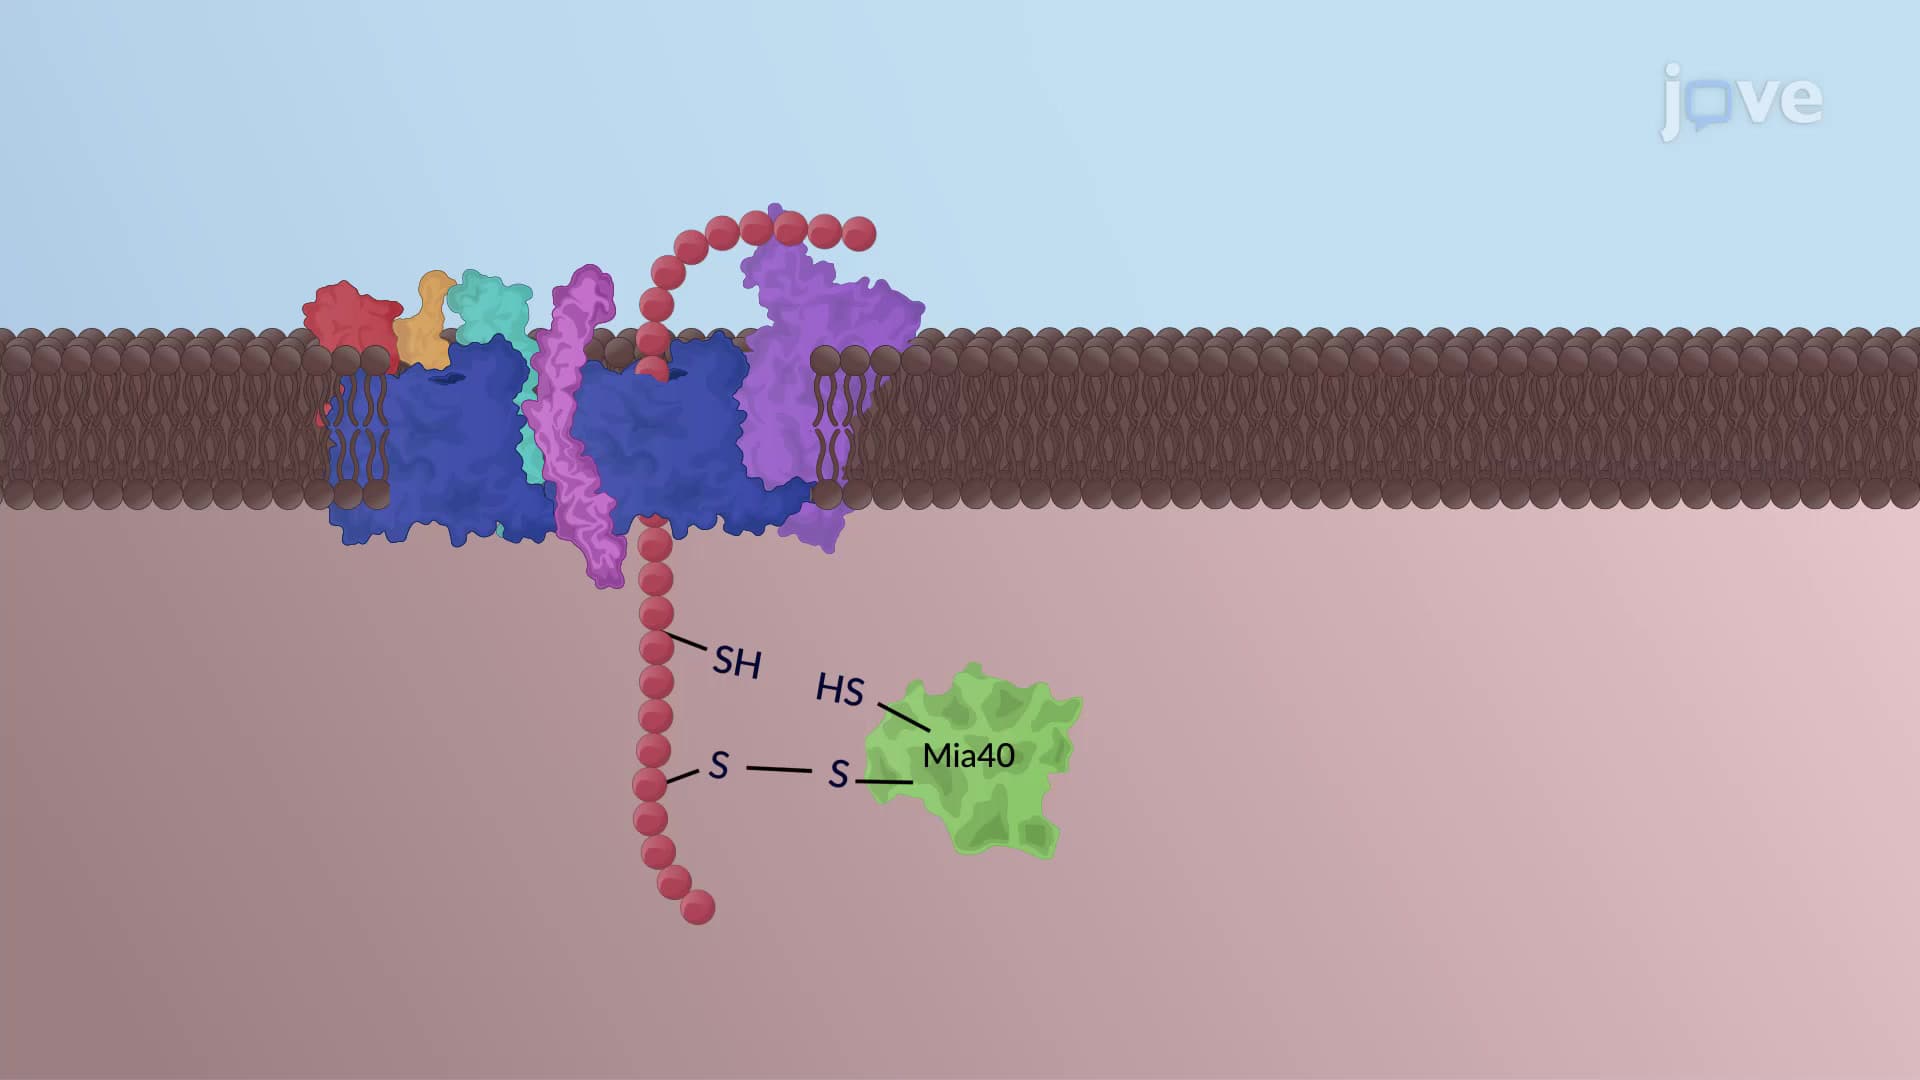
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
13.7K
 01:20
Cotranslational Protein Translocation
11.0K
Translocation of proteins across membranes is an ancient process that occurs even in bacteria and archaebacteria. In fact, the components of the translocation machinery are still conserved between prokaryotes and eukaryotes.
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
11.0K