Energy optimization and bifurcation angles in the microcirculation
Related Experiment Video
Updated: Aug 12, 2026
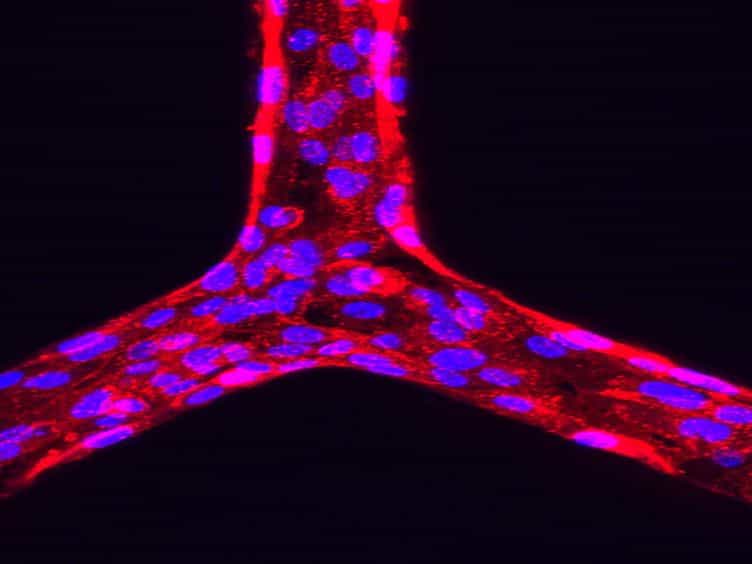
Procedure for the Development of Multi-depth Circular Cross-sectional Endothelialized Microchannels-on-a-chip
Published on: October 21, 2013
1Department of Biophysics, University of Rochester Medical Center, New York 14642, USA.

Abstract:
Our purpose was to examine the relationship between bifurcation angle and energy optimization in the arteriolar microcirculation. We measured bifurcation angles and diameters for sequential branches along a third-order feed arteriole (25 microns) in the superfused cremaster muscle of anesthetized (pentobarbital, 70 mg/kg) Golden hamsters (N = 51). Predicted bifurcation angles were calculated using the diameter data in a model designed to minimize total energy or using four different models each designed to minimize a specific energy cost (vessel wall surface area, vascular volume, wall shear stress, power losses), these models each assuming constant viscosity and that branching occurs with perfect space filling (i.e. junction exponent, x, = 3). The range of the predicted bifurcation angles for any model was small (+/- 10 degrees), and they were not different for the sequential junctions along the feed arteriole, where the observed angles significantly decreased in angle along the feed (first junction, 115 +/- 4.4 degrees; second, 88 +/- 5.2 degrees; third, 76 +/- 4.8 degrees; and last, 57 +/- 3.4 degrees). We next corrected for a nonconstant viscosity by using our in vivo tube hematocrit data and a published relationship among diameter, tube hematocrit, and apparent viscosity. Again assuming that x = 3, the total energy minimization model now predicted that the bifurcation angle was always obtuse and not different for the sequential branches along the feed arteriole (first, 125 +/- 3.3 degrees; second, 124 +/- 3.4 degrees; third, 120 +/- 6.6 degrees; and last, 132 +/- 2.7 degrees); the predicted angles were not correlated with the observed angles (r = 0.25). Using the geometric resistance (diameters) and the angles measured in vivo, and assuming constant viscosity, we next calculated the value of chi for each of the bifurcation junctions for each of the four models described above. The average value of x was not equal to 3 for any of the four models. The value of x decreased along the feed arteriole (first to last branch) from 2.7 +/- 0.26 to 1.6 +/- 0.22 (surface) and from 4.2 +/- 0.36 to 2.9 +/- 0.23 (volume), and x increased along the feed from 3.0 +/- 0.35 to 15.5 +/- 2.6 (shear stress) and from 40 +/- 31 to 82 +/- 49 (power loss). These calculations suggest that both changing viscosity and a changing value for the junction exponent are likely important when examining the energy optimization within the arteriolar microcirculation.
Related Concept Videos
 01:24
Regulation of Angiogenesis and Blood Supply
 01:16
Energy Conservation and Bernoulli's Equation
All the terms in the equation have the dimension of energy per unit volume. The kinetic energy per unit volume is called the kinetic energy density, and the potential energy per unit volume is...
 01:17
Autoregulation of Blood Flow
Chemical Signaling in Autoregulation
Chemical signaling operates at the precapillary sphincter level, inciting either contraction or relaxation.
 01:30
Bernoulli's Equation for Flow Along a Streamline
 01:27
Energy Considerations in Open Channel Flow
 01:27
Applications of Integration to Find Blood Flow