Related Experiment Video
Updated: Aug 15, 2026

Analysis of LINE-1 Retrotransposition at the Single Nucleus Level
Published on: April 23, 2016
A Ty1 integrase nuclear localization signal required for retrotransposition
S P Moore1, L A Rinckel, D J Garfinkel
1ABL-Basic Research Program, NCI-Frederick Cancer Research and Development Center, Maryland 21702-1201, USA.

Abstract:
Ty1 retrotransposition in Saccharomyces cerevisiae requires integrase (IN)-mediated insertion of Ty1 cDNA into the host genome. The transposition components are assembled in the cytoplasm and must cross the nuclear envelope to reach the genomic target, since, unlike animal cell nuclear membranes, the yeast cell nuclear membrane remains intact throughout the cell cycle. We have identified a bipartite nuclear localization signal (NLS) in IN required for Ty1 transposition (Ty1 IN) that directs IN to the nucleus. Mutations in the NLS that specifically abolish nuclear localization inactivate transpositional integration but do not affect reverse transcription, protein processing, or catalytic activity in vitro. No additional Ty1-encoded proteins are required for IN nuclear localization. Intragenic complementation experiments suggest that Ty1 IN functions as a multimer and contains two distinct domains, one required for integration and the other for nuclear localization. Nuclear targeting of the preintegration complex by an IN NLS may prove to be a general strategy used by retrotransposons and retroviruses that infect nondividing cells.
Related Concept Videos
 02:13
Overview of Transposition and Recombination
 02:57
DNA-only Transposons
The donor site from where the transposon is excised is either degraded or...
 03:08
LTR Retrotransposons
The internal coding region of LTR retrotransposons and their mechanism of transposition closely resembles a...
 03:18
Non-LTR Retrotransposons
 01:46
Nuclear Localization Signals and Import
 01:19
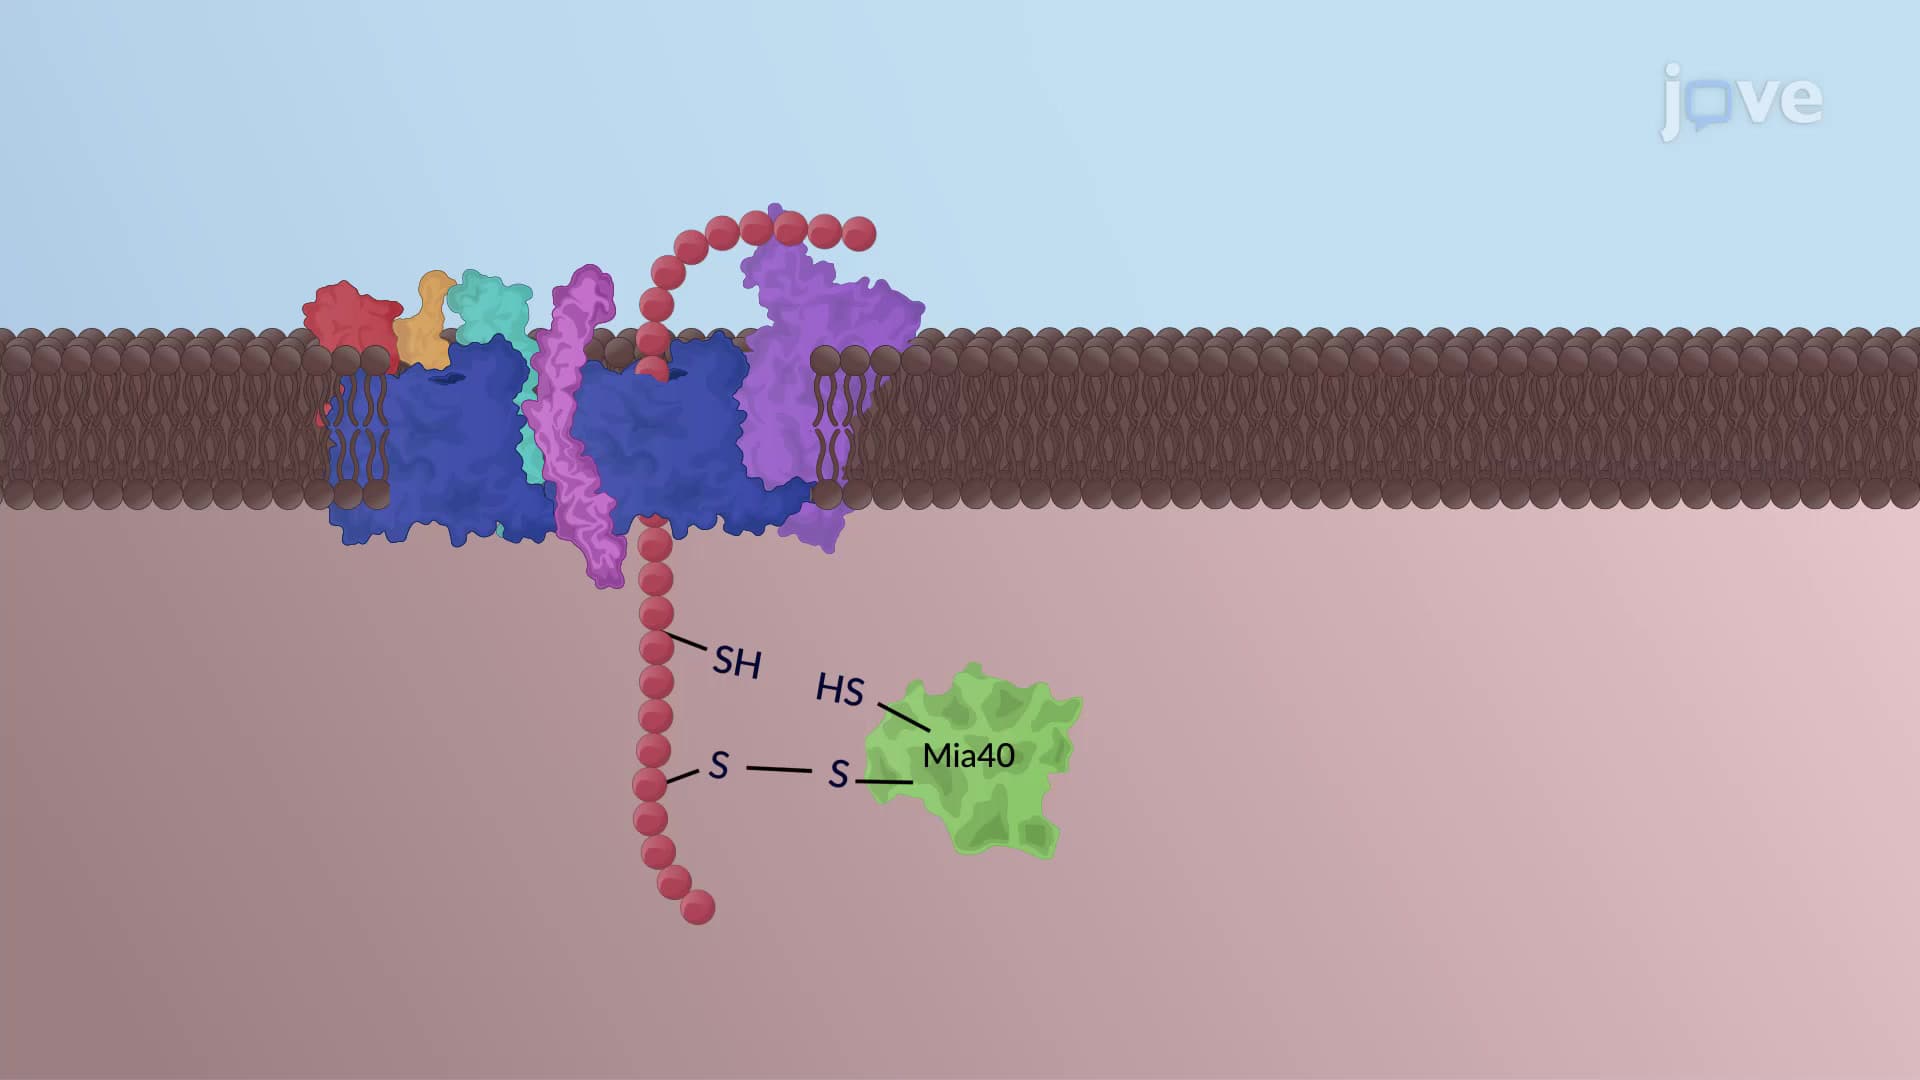
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...