Uncharged S4 residues and cooperativity in voltage-dependent potassium channel activation
Related Experiment Video
Updated: Oct 30, 2026
Recapitulation of an Ion Channel IV Curve Using Frequency Components
Published on: February 8, 2011
C J Smith-Maxwell1, J L Ledwell, R W Aldrich
1Department of Molecular and Cellular Physiology, Stanford University, Stanford, California 94305, USA.

Abstract:
Substitution of the S4 of Shaw into Shaker alters cooperativity in channel activation by slowing a cooperative transition late in the activation pathway. To determine the amino acids responsible for the functional changes in Shaw S4, we created several mutants by substituting amino acids from Shaw S4 into Shaker. The S4 amino acid sequences of Shaker and Shaw S4 differ at 11 positions. Simultaneous substitution of just three noncharged residues from Shaw S4 into Shaker (V369I, I372L, S376T; ILT) reproduces the kinetic and voltage-dependent properties of Shaw S4 channel activation. These substitutions cause very small changes in the structural and chemical properties of the amino acid side chains. In contrast, substituting the positively charged basic residues in the S4 of Shaker with neutral or negative residues from the S4 of Shaw S4 does not reproduce the shallow voltage dependence or other properties of Shaw S4 opening. Macroscopic ionic currents for ILT could be fit by modifying a single set of transitions in a model for Shaker channel gating (Zagotta, W.N., T. Hoshi, and R.W. Aldrich. 1994. J. Gen. Physiol. 103:321-362). Changing the rate and voltage dependence of a final cooperative step in activation successfully reproduces the kinetic, steady state, and voltage-dependent properties of ILT ionic currents. Consistent with the model, ILT gating currents activate at negative voltages where the channel does not open and, at more positive voltages, they precede the ionic currents, confirming the existence of voltage-dependent transitions between closed states in the activation pathway. Of the three substitutions in ILT, the I372L substitution is primarily responsible for the changes in cooperativity and voltage dependence. These results suggest that noncharged residues in the S4 play a crucial role in Shaker potassium channel gating and that small steric changes in these residues can lead to large changes in cooperativity within the channel protein.
More Related Videos
Related Concept Videos
 01:26
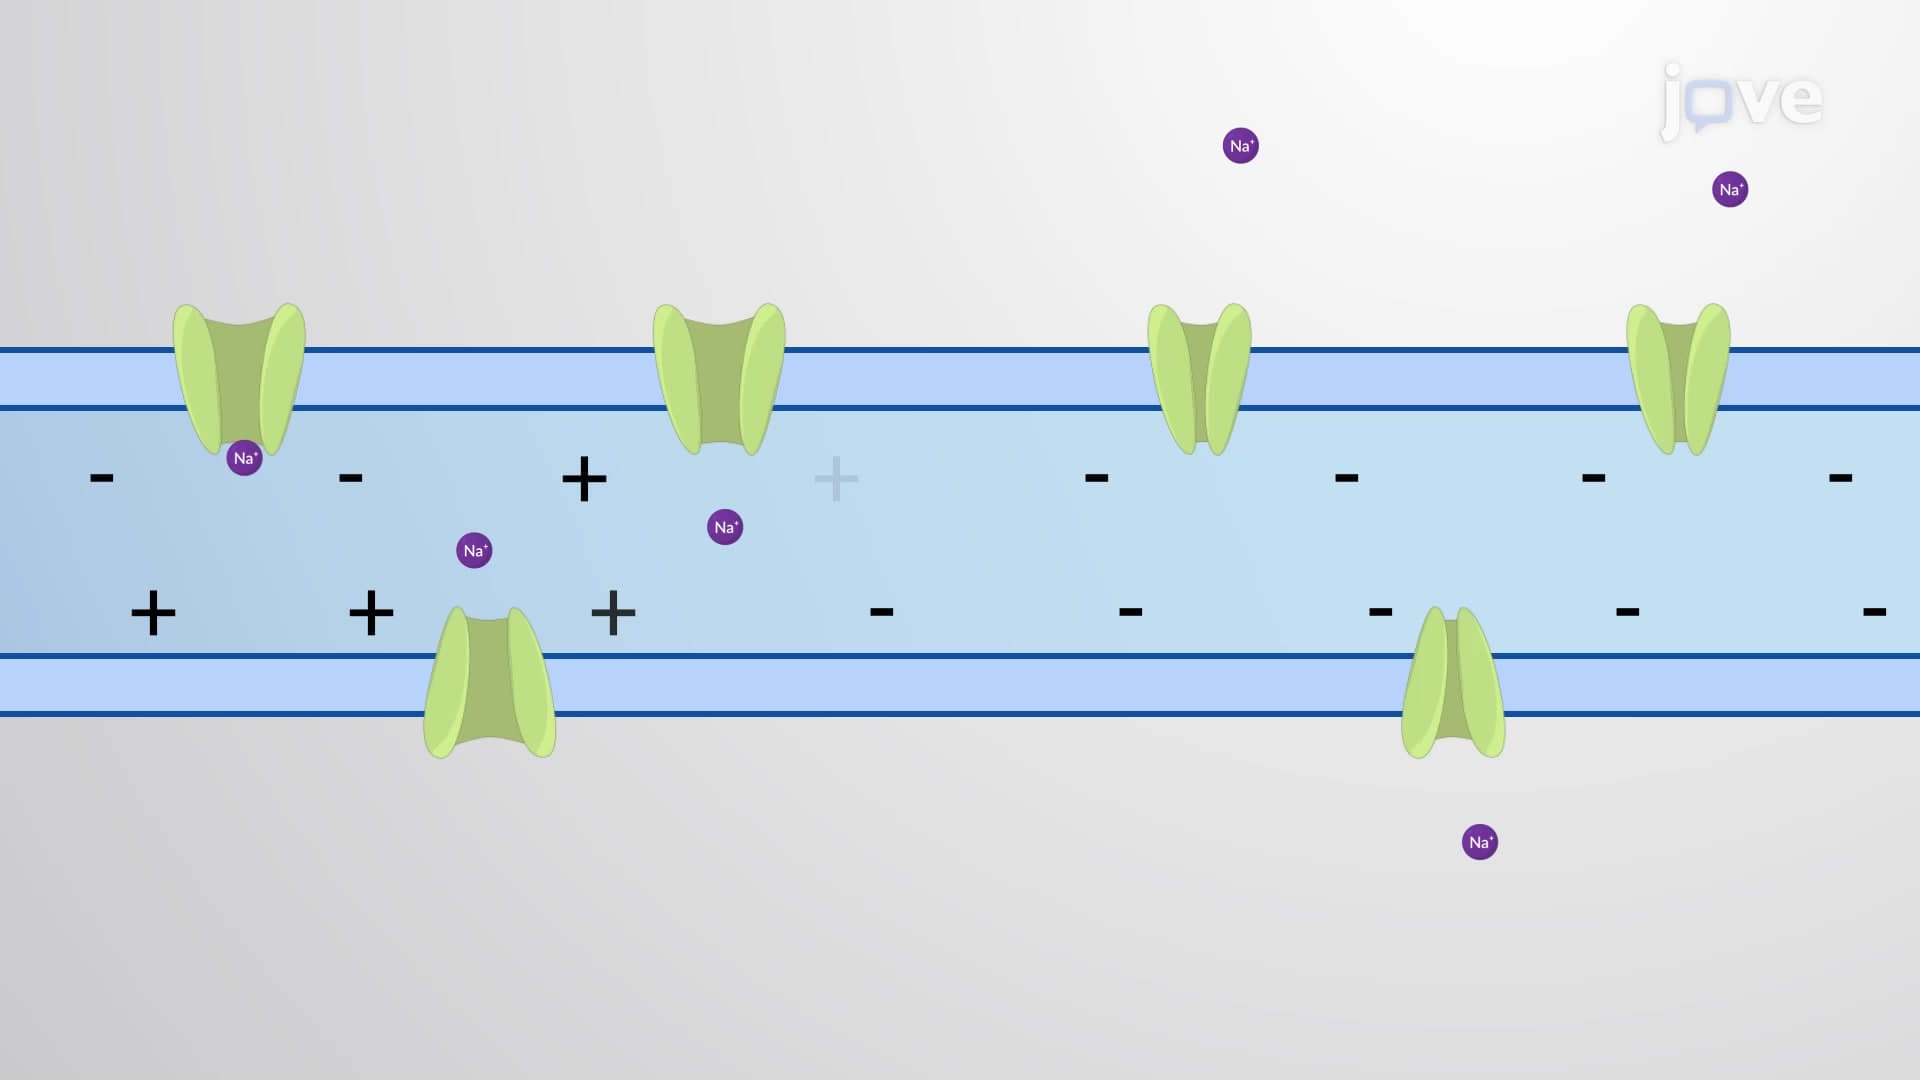
Voltage-gated Ion Channels
Generally, all voltage-gated ion channels have a 'voltage-sensing domain' that spans the lipid bilayer. The charged residues in the sensor move in response to the membrane potential changes that open the channel allowing ions movement. There are several types of...
01:26Voltage-gated Ion Channels
Generally, all voltage-gated ion channels have a 'voltage-sensing domain' that spans the lipid bilayer. The charged residues in the sensor move in response to the membrane potential changes that open the channel allowing ions movement. There are several types of...
 01:30
Ligand-Gated Ion Channel Receptor: Gating Mechanism
 01:19
The Role of Ion Channels in Neuronal Computation
Sometimes a single EPSP is strong enough to induce an action potential in the postsynaptic neuron. However, multiple presynaptic inputs must often create EPSPs around the same time for the postsynaptic neuron to be sufficiently depolarized to fire an action potential.
 01:19
Ligand-gated Ion Channels
Three Subfamilies of Ligand-gated Ion Channels
Ligand-gated ion channels fall into three subfamilies. The 'Cys-loop' includes the nicotinic acetylcholine receptors, γ-aminobutyric acid (GABA), glycine, and 5-hydroxytryptamine receptors. The second one is the 'Pore-loop' channels that include the...
01:19Ligand-gated Ion Channels
Three Subfamilies of Ligand-gated Ion Channels
Ligand-gated ion channels fall into three subfamilies. The 'Cys-loop' includes the nicotinic acetylcholine receptors, γ-aminobutyric acid (GABA), glycine, and 5-hydroxytryptamine receptors. The second one is the 'Pore-loop' channels that include the...