Related Experiment Video
Updated: Aug 11, 2026

Nuclear Migration in the Drosophila Oocyte
Published on: May 13, 2021
Domains of Importin-alpha2 required for ring canal assembly during Drosophila oogenesis
Mátyás Gorjánácz1, István Török, István Pomozi
1Institute of Genetics, Biological Research Center of the Hungarian Academy of Sciences, Szeged, Hungary.

Abstract:
Null-mutation in Drosophila importin-alpha2, such as the deficiency imp-alpha2(D14), causes recessive female sterility with the formation of dumpless eggs. In imp-alpha2(D14) the transfer of nurse cell components to the oocyte is interrupted and the Kelch protein, an oligomeric ring canal actin organizer, is normally produced but fails to associate with the ring canals resulting in their occlusion. To define domains regulating Kelch deposition on ring canals we performed site-directed mutagenesis on protein binding domains and putative phosphorylation sites of Imp-alpha2. Phenotypic analysis of the mutant transgenes in imp-alpha2(D14) revealed that mutations affecting the Imp-beta binding-domain, the dimerization domain, and specific serine residues of putative phosphorylation sites led to a normal or nearly normal oogenesis but arrested early embryonic development, whereas mutations in the nuclear localization signal (NLS) and CAS/exportin binding domains resulted in ring canal occlusion and a drastic nuclear accumulation of the mutant proteins. Deletion of the Imp-beta binding domain also gave rise to a nuclear localization of the mutant protein, which partially retained its function in ring canal assembly. Thus, we propose that mutations in NLS and CAS binding domains affect the deposition of Kelch onto the ring canals and prevent the association of Imp-alpha2 with a negative regulator of Kelch function.
Related Concept Videos
 01:46
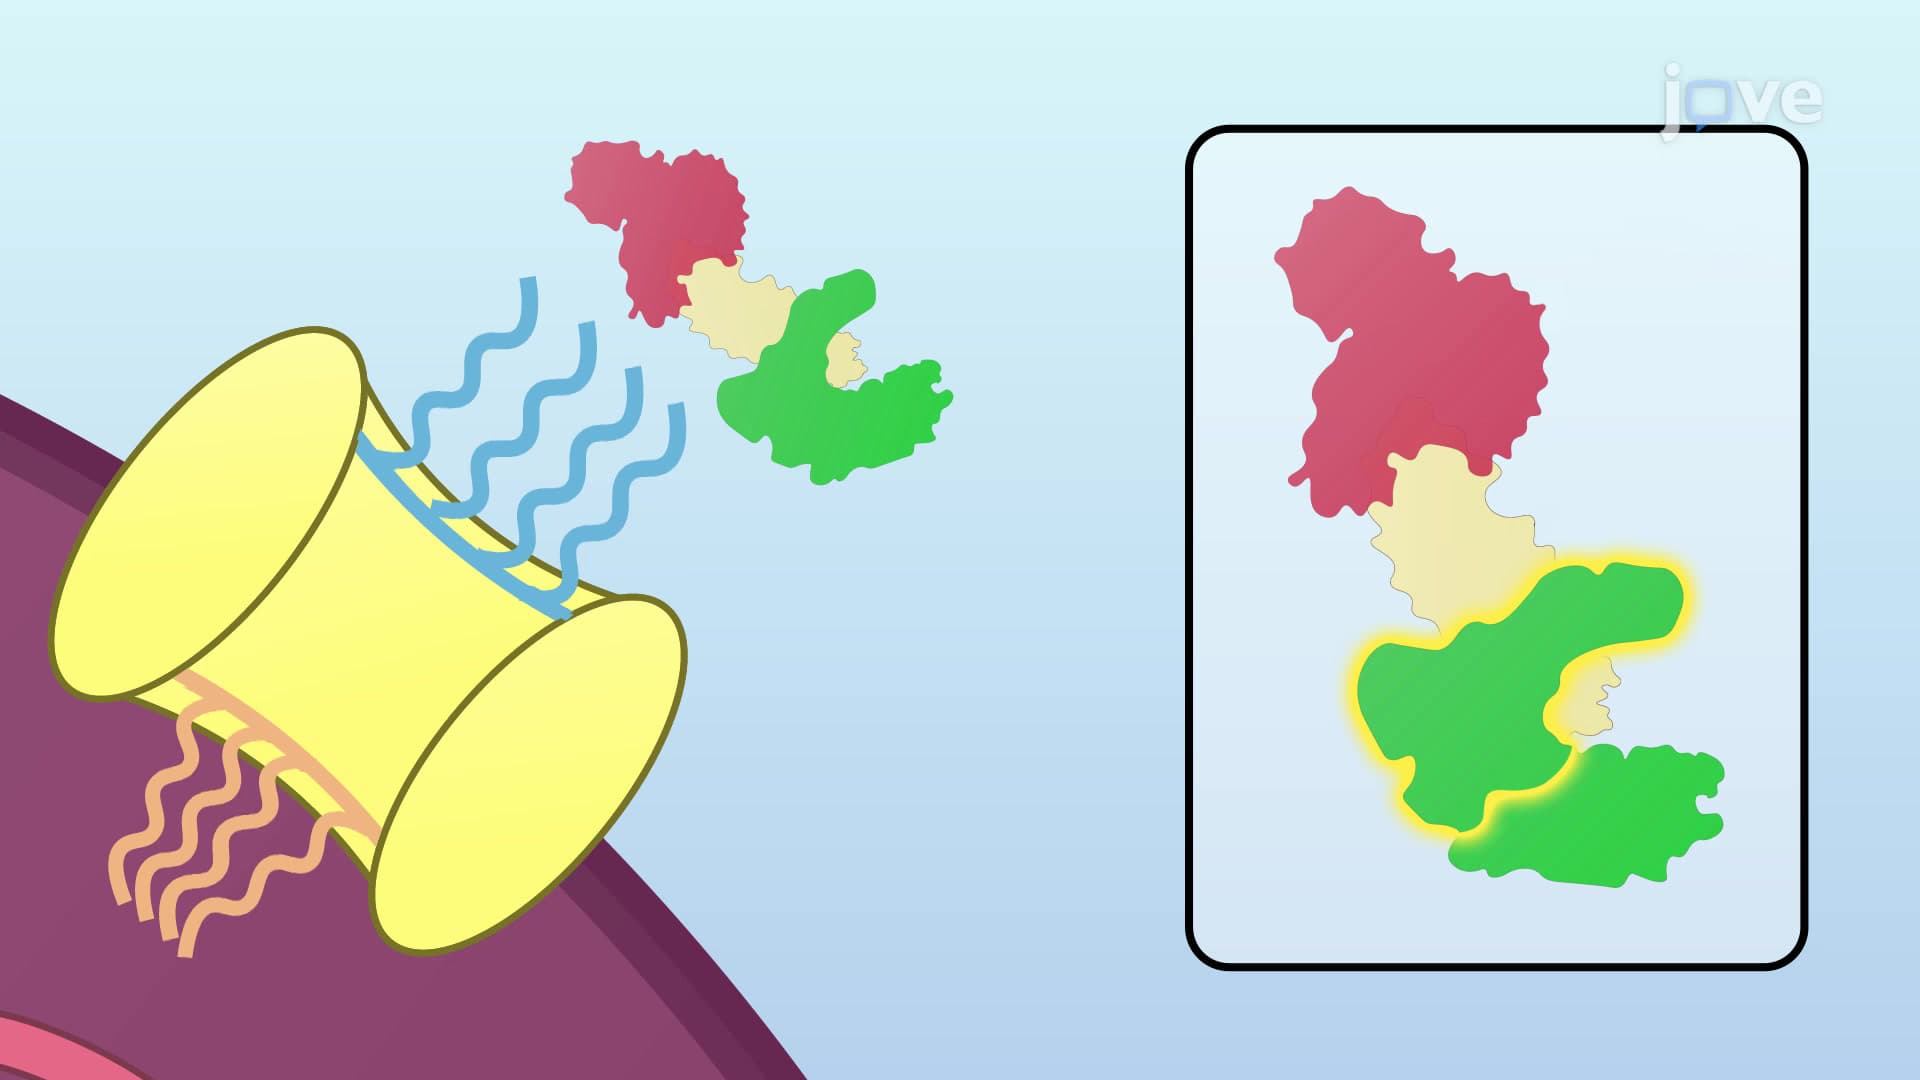
Nuclear Localization Signals and Import
 02:15
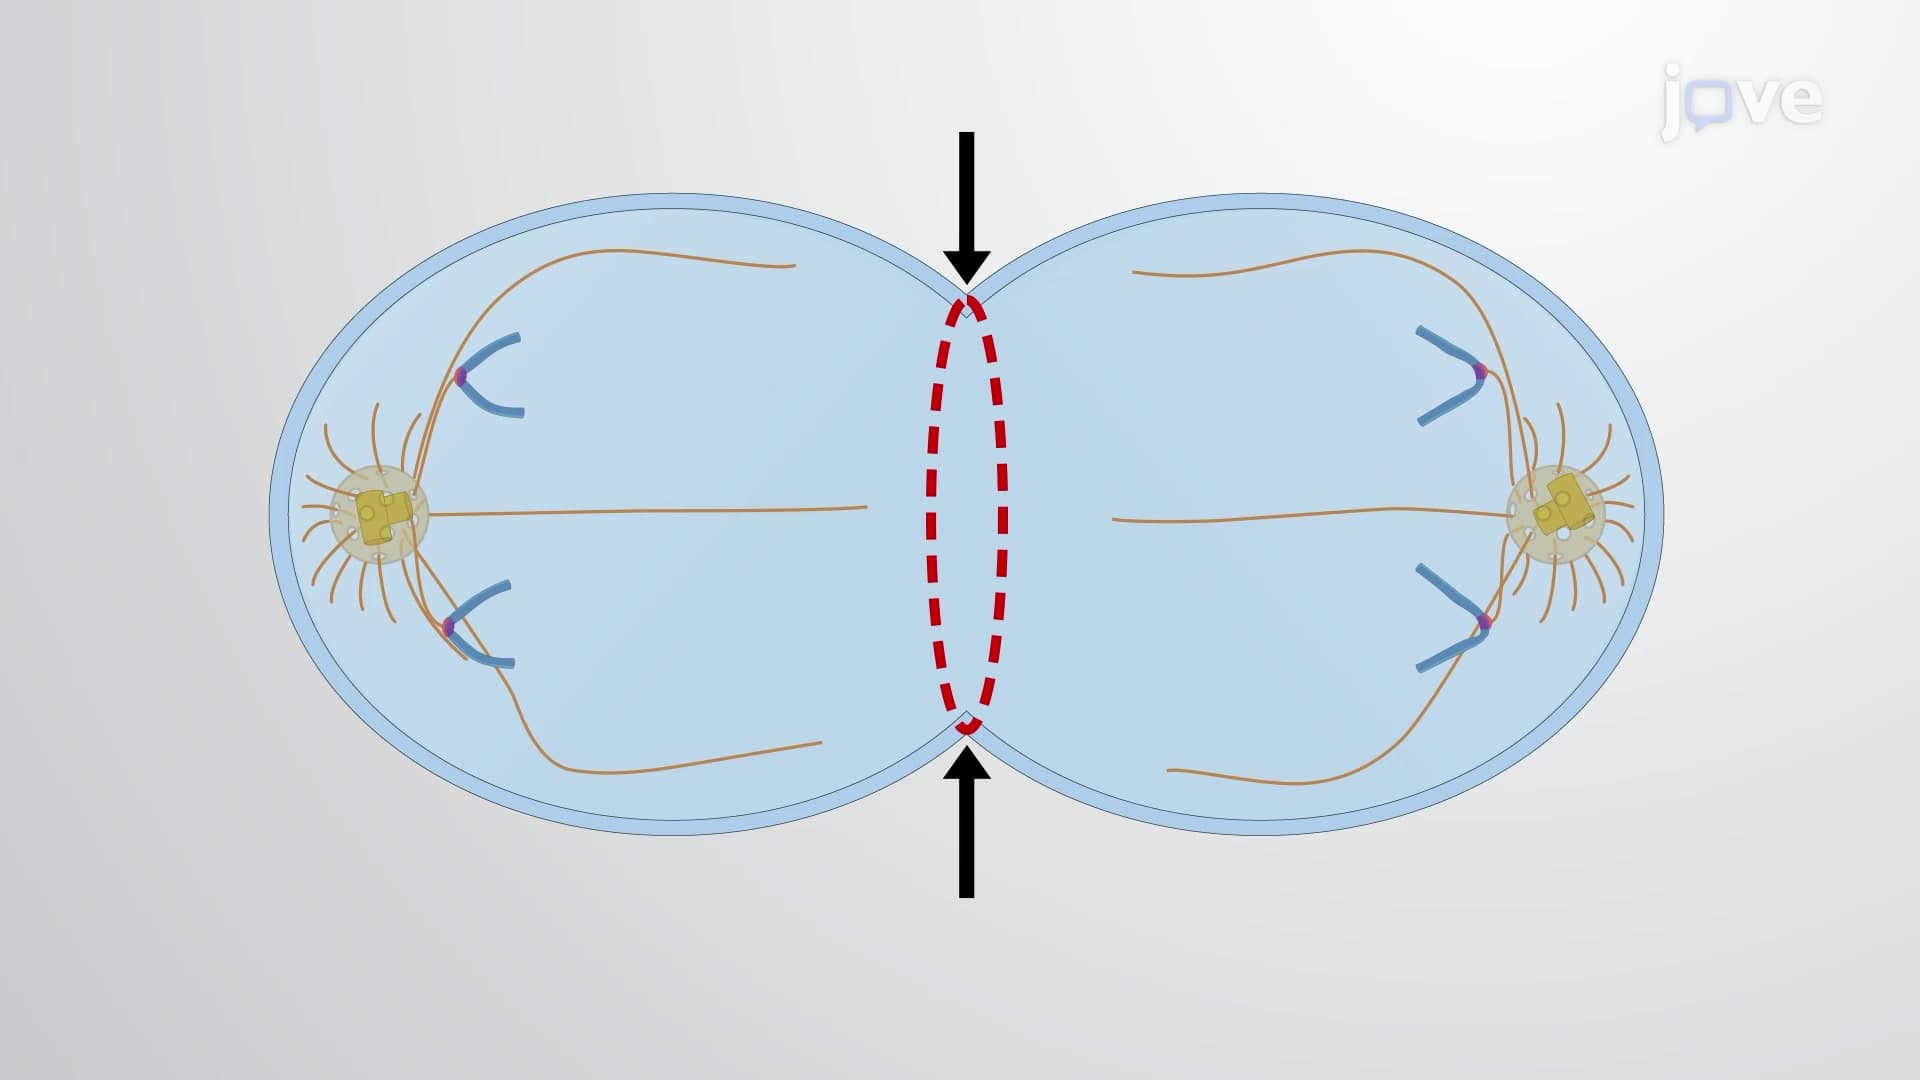
The Contractile Ring
A small GTPase, RhoA, controls the function and assembly of the contractile ring. RhoA belongs to the Ras superfamily of proteins. The activation of formins by RhoA promotes...
 01:27
Protein Import into the Peroxisomes
Peroxisomal Protein Import:
Peroxisomes lack the genetic machinery required to code for their own proteins. Hence, most peroxisomal membrane, lumenal and transmembrane proteins are synthesized in the cytoplasm or ER and transported to the peroxisome...
 01:33
Coat Assembly and GTPases
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
 01:23
Microtubule Formation
 01:12
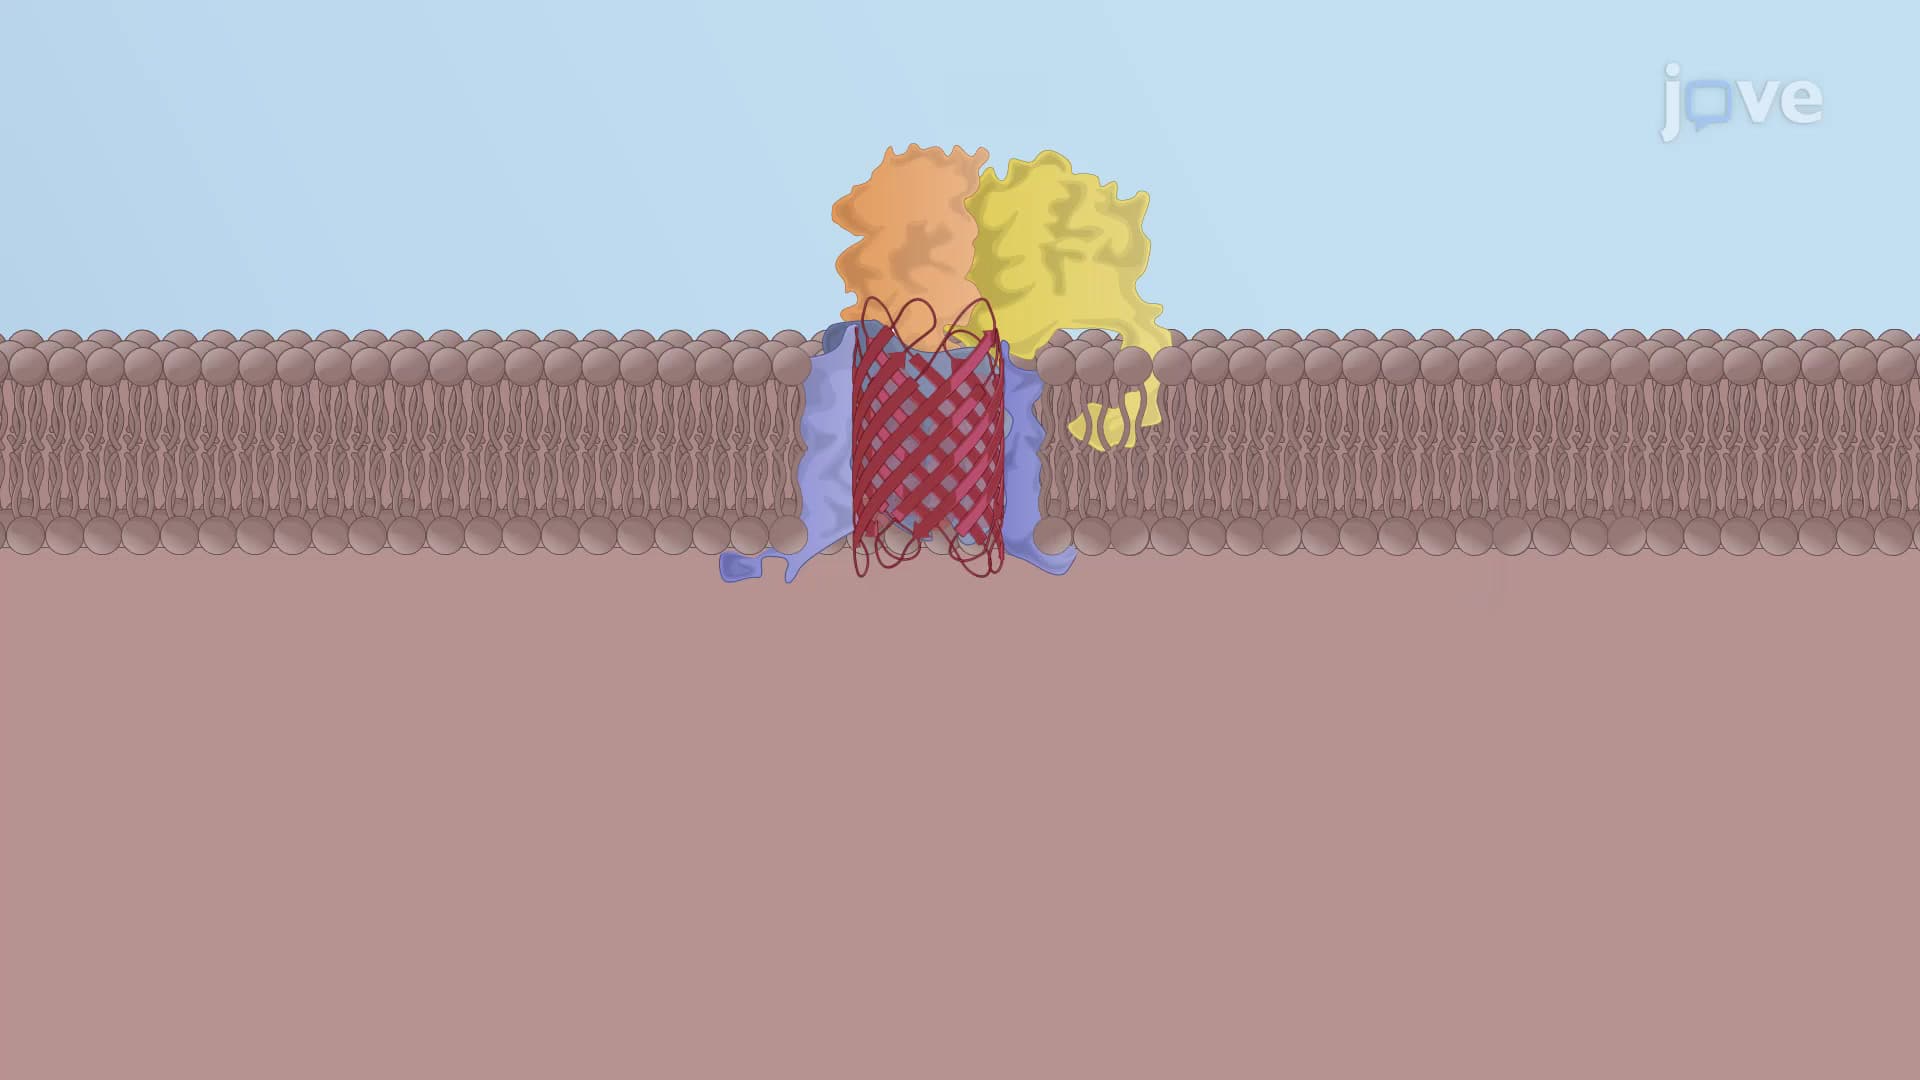
Porin Insertion in the Outer Mitochondrial Membrane
Three models describe the assembly of porins by the SAM complex and their insertion into the outer membrane. Model 1 suggests that porins are assembled outside the SAM channel as the...