Related Experiment Video
Updated: May 4, 2026

Interactions with and Membrane Permeabilization of Brain Mitochondria by Amyloid Fibrils
Published on: September 28, 2019
The N-terminus of α-synuclein is essential for both monomeric and oligomeric interactions with membranes
Nikolai Lorenzen1, Lasse Lemminger1, Jannik Nedergaard Pedersen1
1Interdisciplinary Nanoscience Center (iNANO), Department of Molecular Biology and Genetics, Center for Insoluble Protein Structures (inSPIN), Aarhus University, Gustav Wieds Vej 14, DK-8000 Aarhus C, Denmark.

Abstract:
The intrinsically disordered protein α-synuclein (αSN) is linked to Parkinson's Disease and forms both oligomeric species and amyloid fibrils. The N-terminal part of monomeric αSN interacts strongly with membranes and αSN cytotoxicity has been attributed to oligomers' ability to interact with and perturb membranes. We show that membrane folding of monomeric wt αSN and N-terminally truncated variants correlates with membrane permeabilization. Further, the first 11 N-terminal residues are crucial for monomers' and oligomers' interactions with and permeabilization of membranes. We attribute oligomer permeabilization both to cooperative electrostatic interactions through the N-terminus and interactions mediated by hydrophobic regions in the oligomer.
More Related Videos
 07:56
Utilizing Time-Resolved Protein-Induced Fluorescence Enhancement to Identify Stable Local Conformations One α-Synuclein Monomer at a Time
Published on: May 30, 2021
 08:40
Millisecond Hydrogen/Deuterium-Exchange Mass Spectrometry for the Study of Alpha-Synuclein Structural Dynamics Under Physiological Conditions
Published on: June 23, 2022
Related Concept Videos
 03:03
Amyloid Fibrils
Amyloid deposits were observed as early as 1639 in the liver and the spleen. In 1854, Rudolph Virchow performed iodine staining,...
 01:26
Insertion of Single-pass Transmembrane Proteins in the RER
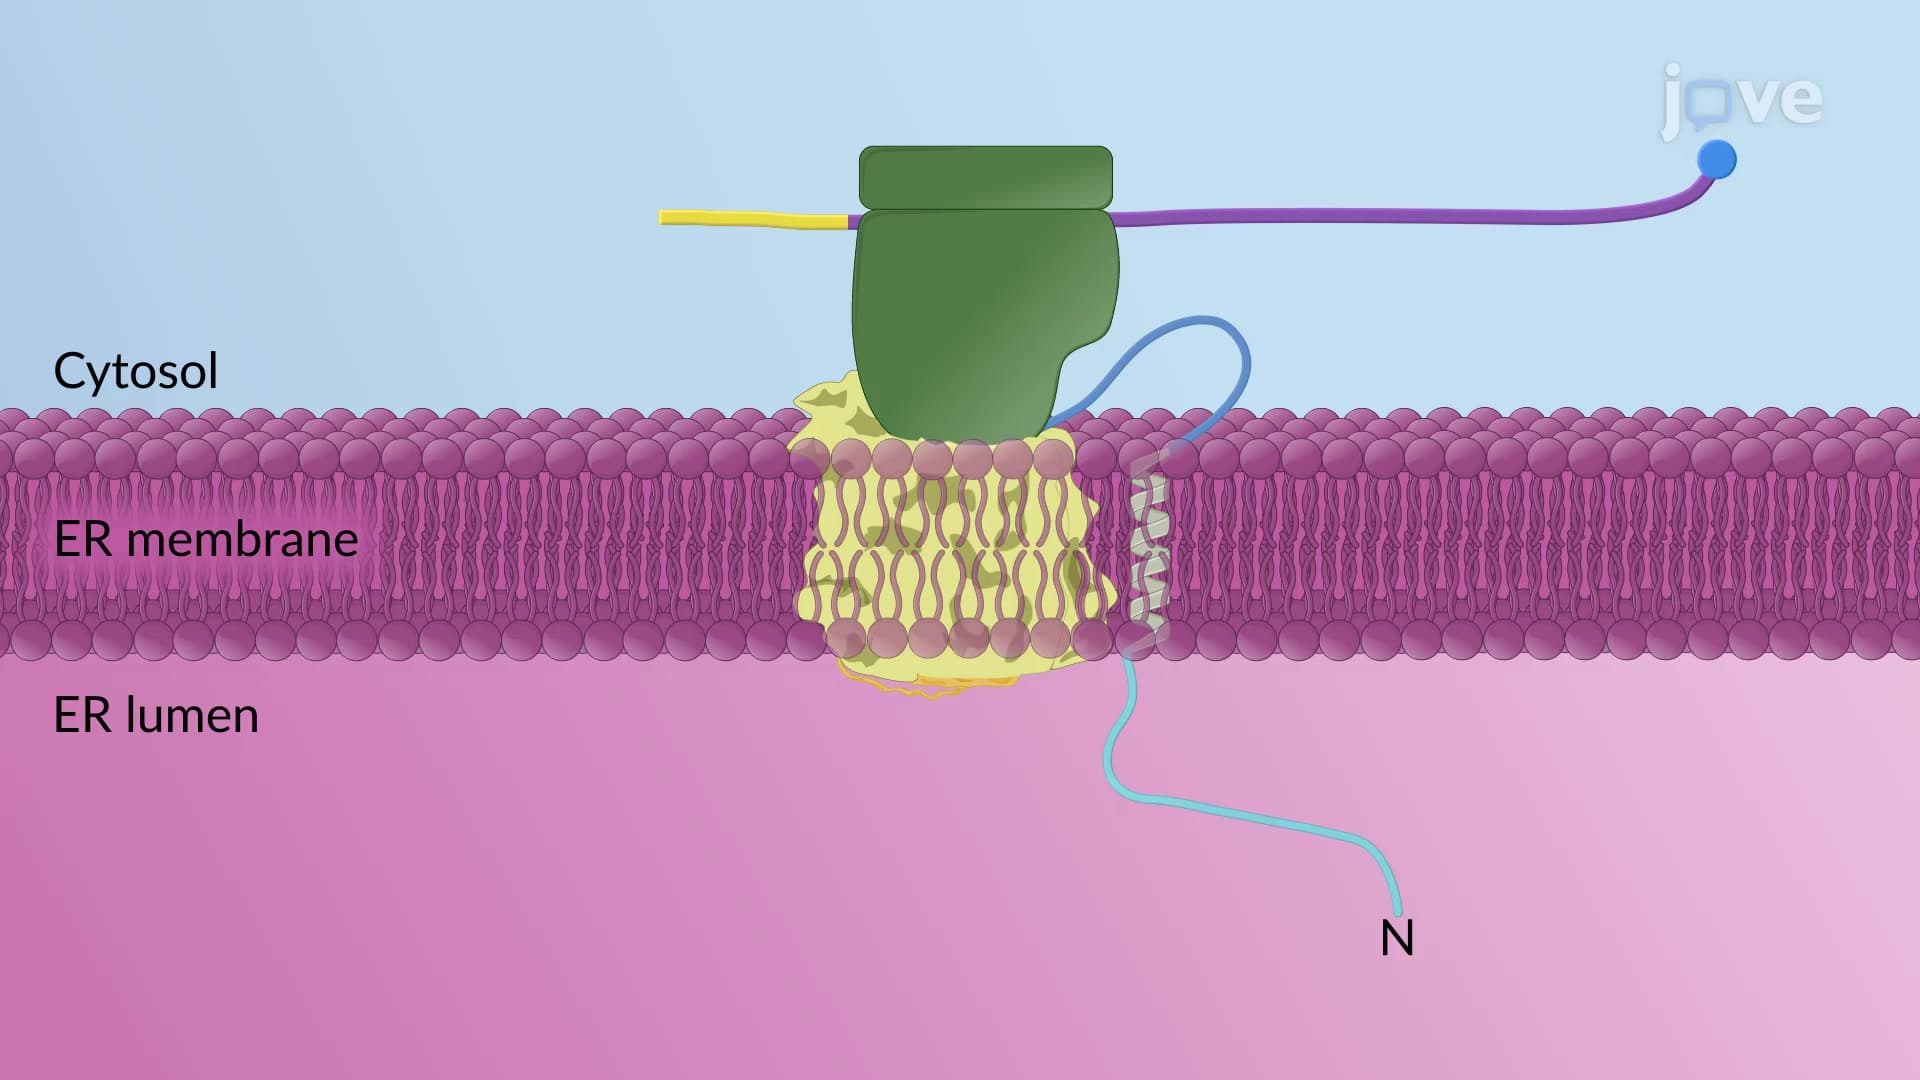
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:39
Mitochondrial Precursor Proteins
Most of the mitochondrial...
 01:45
Tail-anchoring of Proteins in the ER Membrane
 01:29
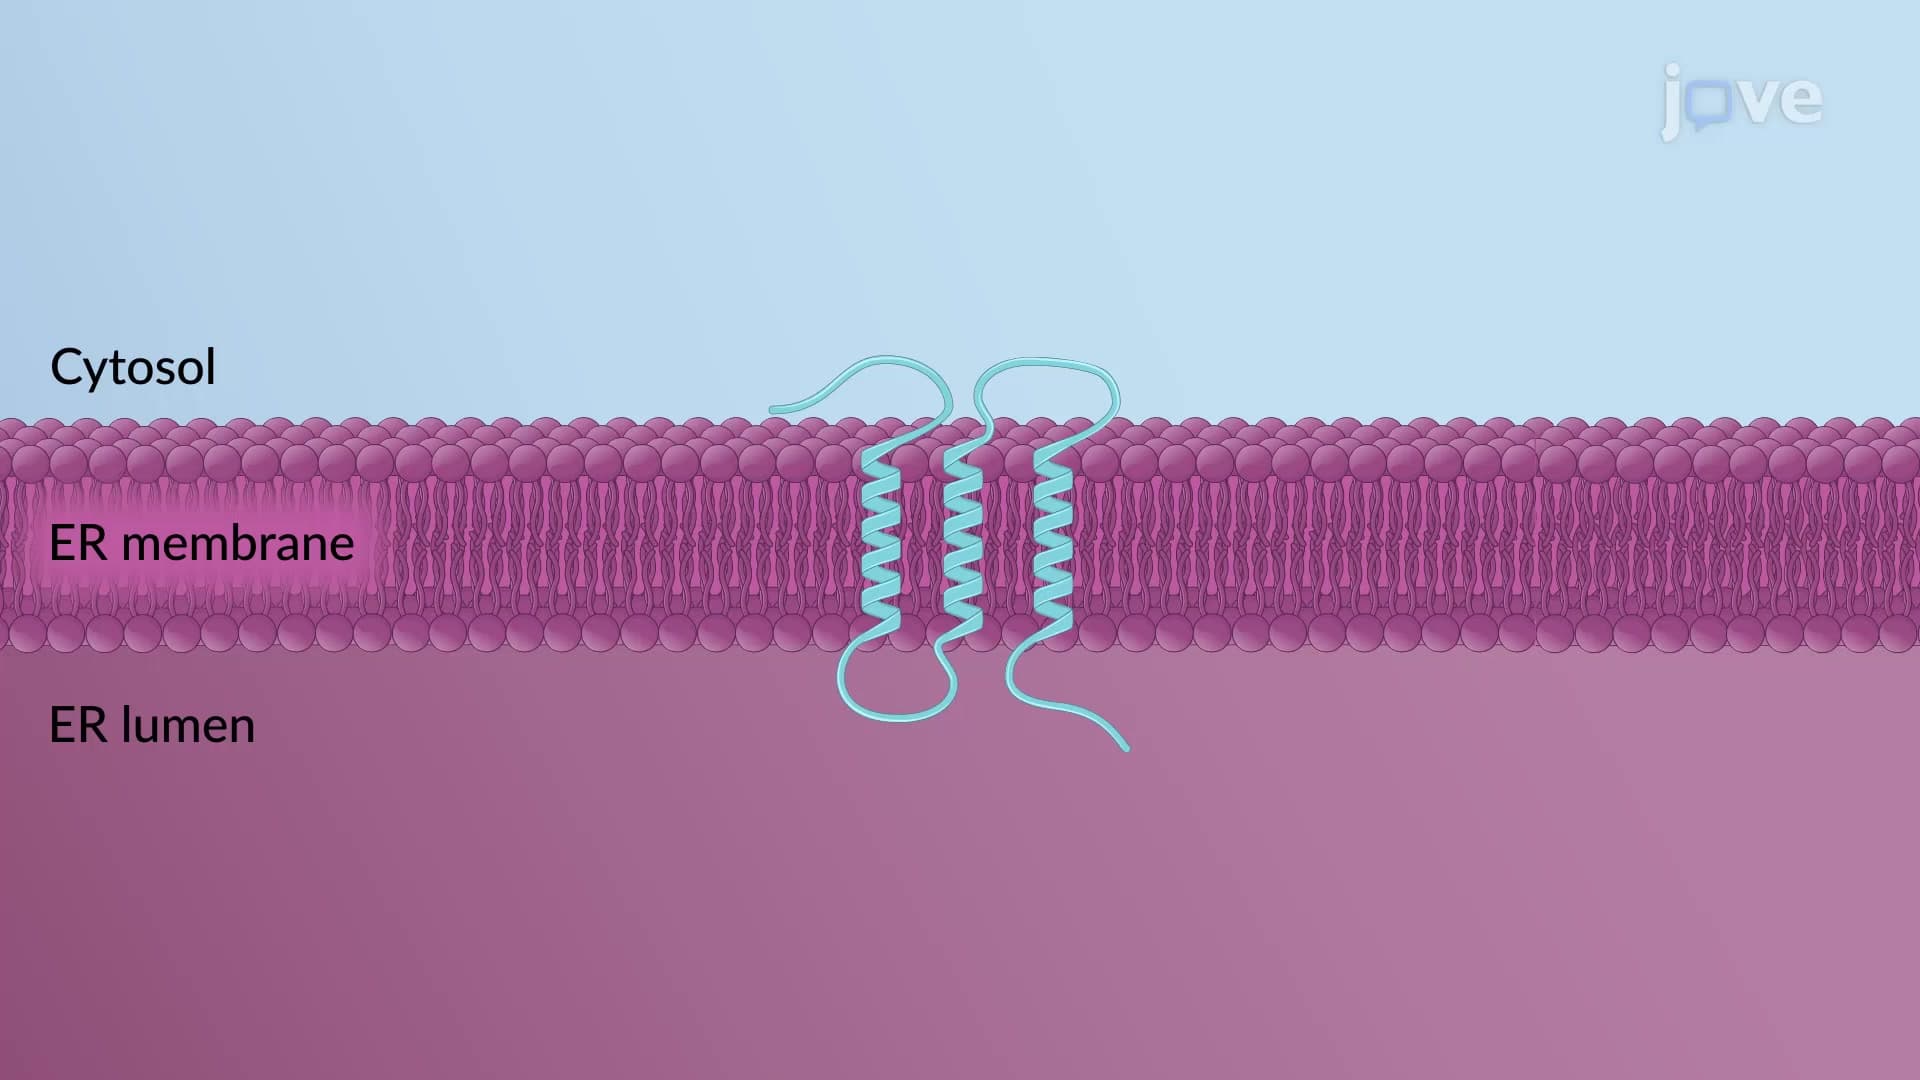
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...