Related Experiment Video
Updated: Feb 19, 2026

Author Spotlight: Advancements in Refractive Surgical Correction for Presbyopia and Exploring Postoperative Visual Acuity
Published on: September 20, 2024
The Relationship Between High-Order Aberration and Anterior Ocular Biometry During Accommodation in Young Healthy
Bilian Ke1,2, Xinjie Mao2,3, Hong Jiang2
1Department of Ophthalmology, Shanghai General Hospital, Shanghai Jiao Tong University School of Medicine, Shanghai, China.

Purpose:
This study investigated the anterior ocular anatomic origin of high-order aberration (HOA) components using optical coherence tomography and a Shack-Hartmann wavefront sensor.
Methods:
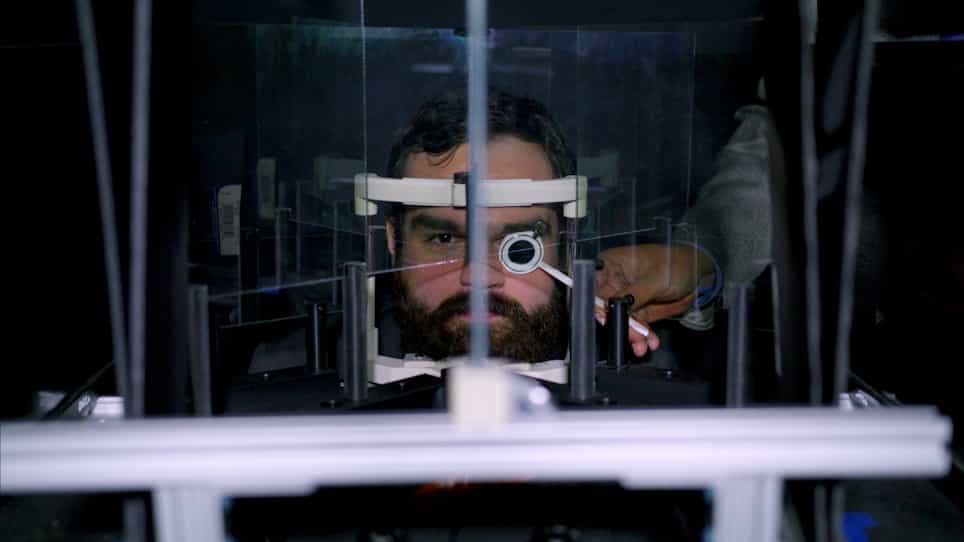
A customized system was built to simultaneously capture images of ocular wavefront aberrations and anterior ocular biometry. Relaxed, 2-diopter (D) and 4-D accommodative states were repeatedly measured in 30 young subjects. Custom software was used to correct optical distortions and measure biometric parameters from the images.
Results:
The anterior ocular biometry changed during 2-D accommodation, in which central lens thickness, ciliary muscle thicknesses at 1 mm posterior to the scleral spur (CMT1), and the maximum value of ciliary muscle thickness increased significantly, whereas anterior chamber depth, CMT3, radius of anterior lens surface curvature (RAL), and radius of posterior lens surface curvature (RPL) decreased significantly. The changes in the anterior ocular parameters during 4-D accommodation were similar to those for the 2-D accommodation. \(\def\upalpha{\unicode[Times]{x3B1}}\)\(\def\upbeta{\unicode[Times]{x3B2}}\)\(\def\upgamma{\unicode[Times]{x3B3}}\)\(\def\updelta{\unicode[Times]{x3B4}}\)\(\def\upvarepsilon{\unicode[Times]{x3B5}}\)\(\def\upzeta{\unicode[Times]{x3B6}}\)\(\def\upeta{\unicode[Times]{x3B7}}\)\(\def\uptheta{\unicode[Times]{x3B8}}\)\(\def\upiota{\unicode[Times]{x3B9}}\)\(\def\upkappa{\unicode[Times]{x3BA}}\)\(\def\uplambda{\unicode[Times]{x3BB}}\)\(\def\upmu{\unicode[Times]{x3BC}}\)\(\def\upnu{\unicode[Times]{x3BD}}\)\(\def\upxi{\unicode[Times]{x3BE}}\)\(\def\upomicron{\unicode[Times]{x3BF}}\)\(\def\uppi{\unicode[Times]{x3C0}}\)\(\def\uprho{\unicode[Times]{x3C1}}\)\(\def\upsigma{\unicode[Times]{x3C3}}\)\(\def\uptau{\unicode[Times]{x3C4}}\)\(\def\upupsilon{\unicode[Times]{x3C5}}\)\(\def\upphi{\unicode[Times]{x3C6}}\)\(\def\upchi{\unicode[Times]{x3C7}}\)\(\def\uppsy{\unicode[Times]{x3C8}}\)\(\def\upomega{\unicode[Times]{x3C9}}\)\(\def\bialpha{\boldsymbol{\alpha}}\)\(\def\bibeta{\boldsymbol{\beta}}\)\(\def\bigamma{\boldsymbol{\gamma}}\)\(\def\bidelta{\boldsymbol{\delta}}\)\(\def\bivarepsilon{\boldsymbol{\varepsilon}}\)\(\def\bizeta{\boldsymbol{\zeta}}\)\(\def\bieta{\boldsymbol{\eta}}\)\(\def\bitheta{\boldsymbol{\theta}}\)\(\def\biiota{\boldsymbol{\iota}}\)\(\def\bikappa{\boldsymbol{\kappa}}\)\(\def\bilambda{\boldsymbol{\lambda}}\)\(\def\bimu{\boldsymbol{\mu}}\)\(\def\binu{\boldsymbol{\nu}}\)\(\def\bixi{\boldsymbol{\xi}}\)\(\def\biomicron{\boldsymbol{\micron}}\)\(\def\bipi{\boldsymbol{\pi}}\)\(\def\birho{\boldsymbol{\rho}}\)\(\def\bisigma{\boldsymbol{\sigma}}\)\(\def\bitau{\boldsymbol{\tau}}\)\(\def\biupsilon{\boldsymbol{\upsilon}}\)\(\def\biphi{\boldsymbol{\phi}}\)\(\def\bichi{\boldsymbol{\chi}}\)\(\def\bipsy{\boldsymbol{\psy}}\)\(\def\biomega{\boldsymbol{\omega}}\)\(\def\bupalpha{\unicode[Times]{x1D6C2}}\)\(\def\bupbeta{\unicode[Times]{x1D6C3}}\)\(\def\bupgamma{\unicode[Times]{x1D6C4}}\)\(\def\bupdelta{\unicode[Times]{x1D6C5}}\)\(\def\bupepsilon{\unicode[Times]{x1D6C6}}\)\(\def\bupvarepsilon{\unicode[Times]{x1D6DC}}\)\(\def\bupzeta{\unicode[Times]{x1D6C7}}\)\(\def\bupeta{\unicode[Times]{x1D6C8}}\)\(\def\buptheta{\unicode[Times]{x1D6C9}}\)\(\def\bupiota{\unicode[Times]{x1D6CA}}\)\(\def\bupkappa{\unicode[Times]{x1D6CB}}\)\(\def\buplambda{\unicode[Times]{x1D6CC}}\)\(\def\bupmu{\unicode[Times]{x1D6CD}}\)\(\def\bupnu{\unicode[Times]{x1D6CE}}\)\(\def\bupxi{\unicode[Times]{x1D6CF}}\)\(\def\bupomicron{\unicode[Times]{x1D6D0}}\)\(\def\buppi{\unicode[Times]{x1D6D1}}\)\(\def\buprho{\unicode[Times]{x1D6D2}}\)\(\def\bupsigma{\unicode[Times]{x1D6D4}}\)\(\def\buptau{\unicode[Times]{x1D6D5}}\)\(\def\bupupsilon{\unicode[Times]{x1D6D6}}\)\(\def\bupphi{\unicode[Times]{x1D6D7}}\)\(\def\bupchi{\unicode[Times]{x1D6D8}}\)\(\def\buppsy{\unicode[Times]{x1D6D9}}\)\(\def\bupomega{\unicode[Times]{x1D6DA}}\)\(\def\bupvartheta{\unicode[Times]{x1D6DD}}\)\(\def\bGamma{\bf{\Gamma}}\)\(\def\bDelta{\bf{\Delta}}\)\(\def\bTheta{\bf{\Theta}}\)\(\def\bLambda{\bf{\Lambda}}\)\(\def\bXi{\bf{\Xi}}\)\(\def\bPi{\bf{\Pi}}\)\(\def\bSigma{\bf{\Sigma}}\)\(\def\bUpsilon{\bf{\Upsilon}}\)\(\def\bPhi{\bf{\Phi}}\)\(\def\bPsi{\bf{\Psi}}\)\(\def\bOmega{\bf{\Omega}}\)\(\def\iGamma{\unicode[Times]{x1D6E4}}\)\(\def\iDelta{\unicode[Times]{x1D6E5}}\)\(\def\iTheta{\unicode[Times]{x1D6E9}}\)\(\def\iLambda{\unicode[Times]{x1D6EC}}\)\(\def\iXi{\unicode[Times]{x1D6EF}}\)\(\def\iPi{\unicode[Times]{x1D6F1}}\)\(\def\iSigma{\unicode[Times]{x1D6F4}}\)\(\def\iUpsilon{\unicode[Times]{x1D6F6}}\)\(\def\iPhi{\unicode[Times]{x1D6F7}}\)\(\def\iPsi{\unicode[Times]{x1D6F9}}\)\(\def\iOmega{\unicode[Times]{x1D6FA}}\)\(\def\biGamma{\unicode[Times]{x1D71E}}\)\(\def\biDelta{\unicode[Times]{x1D71F}}\)\(\def\biTheta{\unicode[Times]{x1D723}}\)\(\def\biLambda{\unicode[Times]{x1D726}}\)\(\def\biXi{\unicode[Times]{x1D729}}\)\(\def\biPi{\unicode[Times]{x1D72B}}\)\(\def\biSigma{\unicode[Times]{x1D72E}}\)\(\def\biUpsilon{\unicode[Times]{x1D730}}\)\(\def\biPhi{\unicode[Times]{x1D731}}\)\(\def\biPsi{\unicode[Times]{x1D733}}\)\(\def\biOmega{\unicode[Times]{x1D734}}\)\({\rm{Z}}_4^0\) decreased significantly during 2-D accommodation, and \({\rm{Z}}_3^{ - 1}\), \({\rm{Z}}_3^1\), \({\rm{Z}}_4^0\), and \({\rm{Z}}_6^0\) shifted to negative values during 4-D accommodation. The change in \({\rm{Z}}_4^0\) negatively correlated with those in CMT1, and the negative change in \({\rm{Z}}_3^1\) correlated with changes in RAL and CMT1.
Conclusions:
HOA components altered during step-controlled accommodative stimuli. Ciliary muscle first contracted during stepwise accommodation, which may directly contribute to the reduction of spherical aberration (SA). The lens morphology was then altered, and the change in anterior lens surface curvature was related to the variation of coma.